欢迎访问作物学报,今天是
作物学报 ›› 2023, Vol. 49 ›› Issue (6): 1466-1479.doi: 10.3724/SP.J.1006.2023.22039
丁杰荣1,**( ), 马雅美1,**(), 潘发枝2, 江立群1, 黄文洁3, 孙炳蕊1, 张静1, 吕树伟1, 毛兴学1, 于航1, 李晨1,*(), 刘清1,*()
DING Jie-Rong1,**(), MA Ya-Mei1,**(), PAN Fa-Zhi2, JIANG Li-Qun1, HUANG Wen-Jie3, SUN Bing-Rui1, ZHANG Jing1, LYU Shu-Wei1, MAO Xing-Xue1, YU Hang1, LI Chen1,*(), LIU Qing1,*()
摘要:
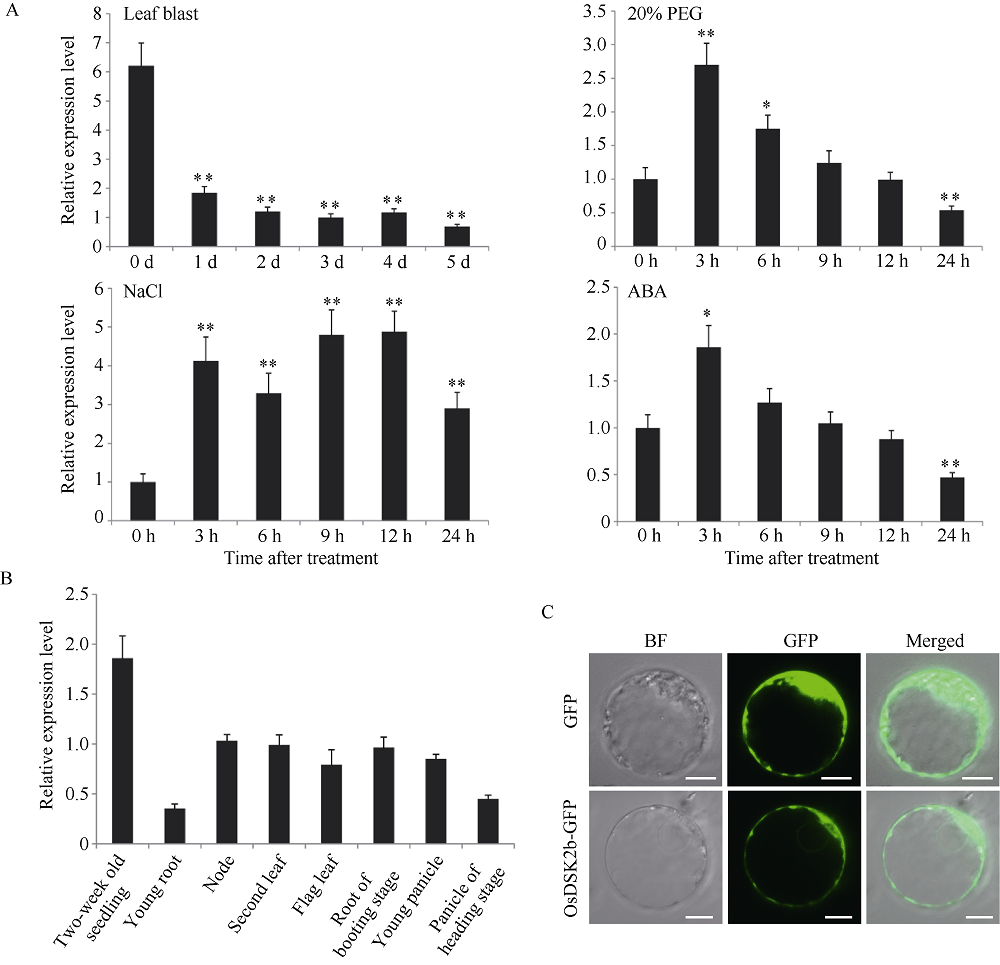
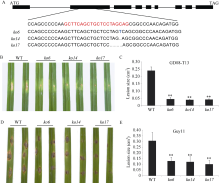
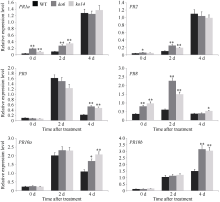
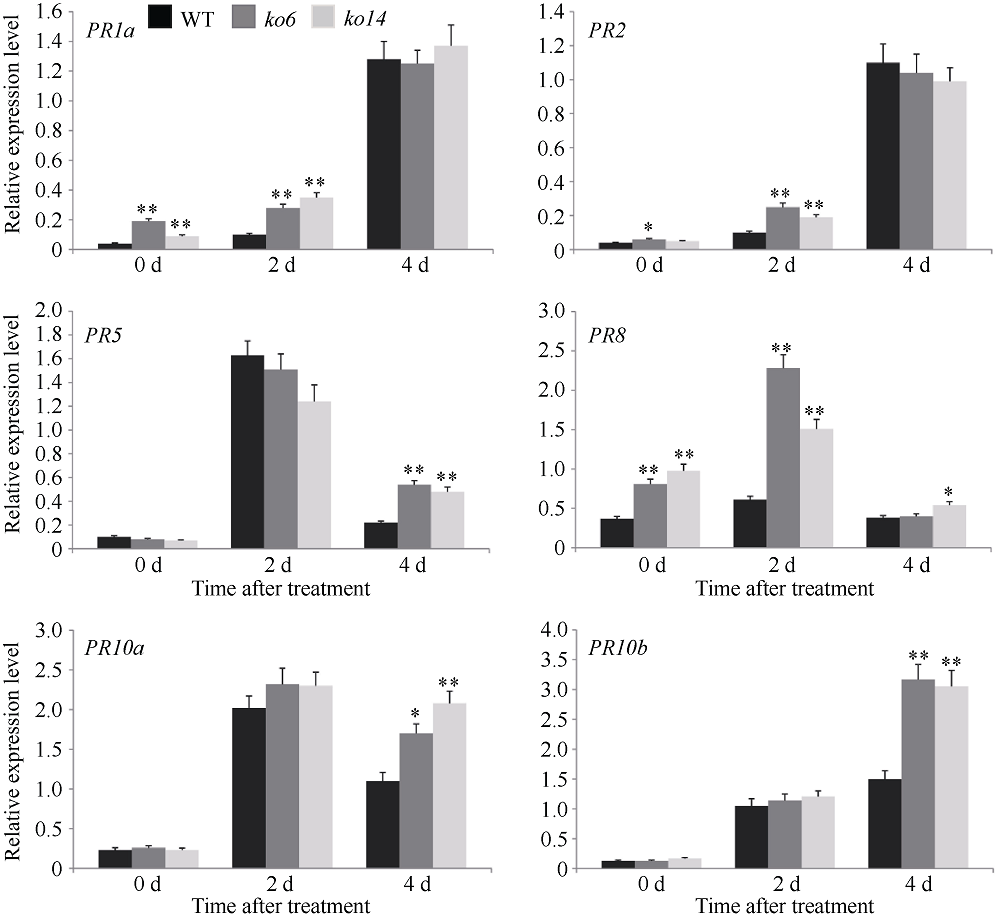
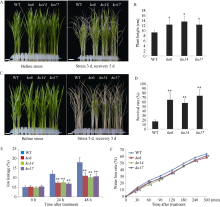
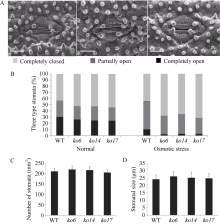
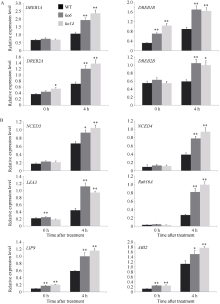
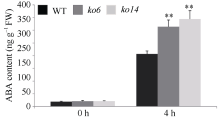
泛素受体蛋白DSK2 (dominant suppressor of KAR2)在植物生长发育和逆境胁迫中发挥重要作用, 但其在水稻抗病和渗透胁迫中的作用尚未见报道。本研究发现OsDSK2b受多种逆境的调控, 该基因的表达水平在稻瘟病菌侵染和20% PEG-6000处理后显著降低。时空表达分析表明OsDSK2b基因在三叶期幼苗中的表达水平最高, 亚细胞定位结果显示该蛋白定位于细胞质。接种稻瘟病菌(GD08-T13和Guy11)后, 敲除植株的病斑面积约为0.05 cm2和0.10~0.13 cm2, 远小于野生型植株的病斑面积(0.24 cm2和0.31 cm2)。敲除OsDSK2b显著增强水稻的叶瘟抗性。而且在病原菌侵染后, 敲除植株中病程相关蛋白(PR)基因的表达受到明显诱导。敲除OsDSK2b也显著增强水稻的渗透胁迫抗性, 20% PEG-6000模拟渗透胁迫处理后, OsDSK2b敲除植株的存活率为58.3%~74.0%, 显著高于野生型植株的存活率(17.0%)。OsDSK2b敲除植株的离子渗透率和植株失水率则显著低于野生型植株。扫描显微镜的结果表明, 无论在20% PEG-6000处理前后, 敲除OsDSK2b能够促进气孔的闭合, 且在20% PEG-6000处理后, 这种促进作用会更强。此外, qRT-PCR结果表明, 在20% PEG-6000处理后, OsDSK2b敲除植株中DREB基因以及脱落酸(ABA)合成或通路相关基因的表达水平显著高于野生型植株, 且敲除植株ko6和ko14的内源ABA含量分别为314.2 ng g-1和344.4 ng g-1, 显著高于野生型植株的内源ABA含量(206.8 ng g-1), 揭示OsDSK2b参与调控渗透胁迫的过程同时涉及ABA依赖和ABA非依赖途径。本研究通过解析OsDSK2b基因在水稻应对生物与非生物胁迫时所发挥的调控作用, 为水稻抗性品种的选育提供了新的候选基因。
| [1] |
王亦栖, 余炳伟, 颜爽爽, 邱正坤, 陈长明, 雷建军, 田时炳, 曹必好. 植物泛素基因研究进展. 中国农学通报, 2020, 36(20): 14-22.
doi: 10.11924/j.issn.1000-6850.casb20190500148 |
|
Wang Y Q, Yu B W, Yan S S, Qiu Z K, Chen C M, Tian S B, Cao B H. Advances in research on plant ubiquitin genes. Chin Agric Sci Bull, 2020, 36(20): 14-22. (in Chinese with English abstract)
doi: 10.11924/j.issn.1000-6850.casb20190500148 |
|
| [2] | 盛仙永. 泛素/蛋白酶体途径在青扦花粉萌发及花粉管生长过程中的作用. 西北大学博士学位论文, 陕西西安, 2006. |
| Sheng X Y. Roles of the Ubiquitin/Proteasome Pathway in Picea wilsonii Pollen Germination and Tube Growth. PhD Dissertation of Northwest University, Xi’an, Shaanxi, China, 2006. (in Chinese with English abstract) | |
| [3] |
Ko J H, Yang S H, Han K H. Upregulation of an Arabidopsis RING-H2 gene, XERICO, confers drought tolerance through increased abscisic acid biosynthesis. Plant J, 2006, 47: 343-355.
doi: 10.1111/tpj.2006.47.issue-3 |
| [4] |
Xie D X, Feys B F, James S, Nieto-Rostro M, Turner J G. COI1: an Arabidopsis gene required for jasmonate-regulated defense and fertility. Science, 1998, 280: 1091-1094.
doi: 10.1126/science.280.5366.1091 pmid: 9582125 |
| [5] |
Fu H, Lin Y L, Fatimababy A S. Proteasomal recognition of ubiquitylated substrates. Trends Plant Sci, 2010, 15: 375-386.
doi: 10.1016/j.tplants.2010.03.004 pmid: 20399133 |
| [6] |
Zhang H, Yang X, Ying Z, Liu J, Liu Q. Toxoplasma gondii UBL-UBA shuttle protein DSK2s are important for parasite intracellular replication. Int J Mol Sci, 2021, 22: 7943.
doi: 10.3390/ijms22157943 |
| [7] |
Wang J, Qin H, Zhou S, Wei P C, Zhang H W, Zhou Y, Miao Y C, Huang R F. The ubiquitin-binding protein OsDSK2a mediates seedling growth and salt responses by regulating gibberellin metabolism in rice. Plant Cell, 2020, 32: 414-428.
doi: 10.1105/tpc.19.00593 |
| [8] |
Fatimababy A S, Lin Y L, Usharani R, Radjacommare R, Wang H T, Tsai H L, Lee Y, Fu H. Cross-species divergence of the major recognition pathways of ubiquitylated substrates for ubiquitin/26S proteasome-mediated proteolysis. FEBS J, 2010, 277: 796-816.
doi: 10.1111/j.1742-4658.2009.07531.x pmid: 20059542 |
| [9] |
Díaz-Martínez L A, Kang Y, Walters K J, Clarke D J. Yeast UBL-UBA proteins have partially redundant functions in cell cycle control. Cell Div, 2006, 1: 28.
pmid: 17144915 |
| [10] |
Wang D Y, Lv C, Guan Y, Ni X Y, Wu F Z. Dsk2 involves in conidiation, multi-stress tolerance and thermal adaptation in Beauveria bassiana. Environ Microbiol Rep, 2021, 13: 384-393.
doi: 10.1111/emi4.v13.3 |
| [11] |
Kaur N, Zhao Q Z, Xie Q, Hu J P. Arabidopsis RING peroxins are E3 ubiquitin ligases that interact with two homologous ubiquitin receptor proteins. J Integr Plant Biol, 2013, 55: 108-120.
doi: 10.1111/jipb.12014 |
| [12] |
汪文娟, 苏菁, 陈深, 杨健源, 陈凯玲, 冯爱卿, 汪聪颖, 封金奇, 陈炳, 朱小源. 广东省侵染美香占2号的稻瘟病菌致病性及无毒基因变异分析. 中国农业科学, 2022, 55: 1346-1358.
doi: 10.3864/j.issn.0578-1752.2022.07.007 |
| Wang E J, Su J, Chen S, Yang J Y, Chen K L, Feng A Q, Wang C Y, Feng J Q, Chen B, Zhu X Y. Pathogenicity and avirulence genes variation of Magnaporthe oryzae from a rice variety Meixiangzhan 2 in Guangdong province. Sci Agric Sin, 2022, 55: 1346-1358. (in Chinese with English abstract) | |
| [13] |
Muthukrishnan S, Liang G H, Trick H N, Gill B S. Pathogenesis-related proteins and their genes in cereals. Plant Cell Tissue Organ Cult, 2001, 64: 93-114.
doi: 10.1023/A:1010763506802 |
| [14] |
Alexander D, Goodman R M, Gut-Rella M, Glascock C, Weymann K, Friedrich L, Maddox D, Ahl-Goy P, Luntz T, Ward E. Increased tolerance to two oomycete pathogens in transgenic tobacco expressing pathogenesis-related protein 1a. Proc Natl Acad Sci USA, 1993, 90: 7327-7331.
doi: 10.1073/pnas.90.15.7327 pmid: 8346252 |
| [15] |
Kauffmann S, Legrand M, Geoffroy P, Fritig B. Biological function of ‘pathogenesis-related’ proteins: four PR proteins of tobacco have 1,3-β-glucanase activity. EMBO J, 1987, 6: 3209-3212.
doi: 10.1002/j.1460-2075.1987.tb02637.x pmid: 16453802 |
| [16] |
Datta K, Velazhahan R, Oliva N, Ona I, Mew T, Khush G S, Muthukrishnan S, Datta S K. Over-expression of the cloned rice thaumatin-like protein (PR-5) gene in transgenic rice plants enhances environmental friendly resistance to Rhizoctonia solani causing sheath blight disease. Theor Appl Genet, 1999, 98: 1138-1145.
doi: 10.1007/s001220051178 |
| [17] | Park C H, Kim S, Park J Y, Ahn I P, Jwa N S, Im K H, Lee Y H. Molecular characterization of a pathogenesis-related protein 8 gene encoding a class III chitinase in rice. Mol Cells, 2004, 17: 144-150. |
| [18] |
Midoh N, Iwata M. Cloning and characterization of a probenazole-inducible gene for an intracellular pathogenesis-related protein in rice. Plant Cell Physiol, 1996, 37: 9-18.
doi: 10.1093/oxfordjournals.pcp.a028918 pmid: 8720923 |
| [19] | 侯明明. 病程相关蛋白质在水稻发育及与白叶枯病菌互作过程中的表达研究. 河北农业大学硕士论文, 河北保定, 2011. |
| Hou M M. Characteristic Expression of Pathogenesis-related Proteins in Rice Development and Interaction with Xanthomonas oryzae pv. oryzae. MS Thesis of Hebei Agricultural University, Baoding, Hebei, China, 2011. (in Chinese with English abstract) | |
| [20] | 郑家国, 任光俊, 陆贤军, 姜心禄. 花后水分亏缺对水稻产量和品质的影响. 中国水稻科学, 2003, 17: 239-243. |
| Zheng J G, Ren G J, Lu X J, Jiang X L. Effects of water stress on rice grain yield and quality after heading stage. Chin J Rice Sci, 2003, 17: 239-243. (in Chinese with English abstract) | |
| [21] | 王平荣, 邓晓建, 高晓玲, 陈静, 万佳, 姜华, 徐正君. DREB 转录因子研究进展. 遗传, 2006, 28: 369-374. |
| Wang P R, Deng X J, Guo X L, Chen J, Wang J, Jiang H, Xu Z J. Progress in the study on DREB transcription factor. Hereditas (Beijing), 2006, 28: 369-374. (in Chinese with English abstract) | |
| [22] |
Liu Q, Yan S J, Huang W J, Yang J Y, Dong J F, Zhang S H, Zhao J L, Yang T F, Mao X X, Zhu X Y, Liu B, 2018b. NAC transcription factor ONAC066 positively regulates disease resistance by suppressing the ABA signaling pathway in rice. Plant Mol Biol, 98: 289-302.
doi: 10.1007/s11103-018-0768-z |
| [23] | 王彬, 陈敏氡, 林亮, 叶新如, 朱海生, 温庆放. 植物干旱胁迫的信号通路及相关转录因子研究进展. 西北植物学报, 2020, 40: 792-1806. |
| Wang B, Chen M D, Lin L, Ye X R, Zhu H S, Wen Q F. Signal plant pathways and related transcription factors of drought stress in plants. Acta Bot Boreali-Occident Sin, 2020, 40: 1792-1806. (in Chinese with English abstract) | |
| [24] |
Xie X R, Ma X L, Zhu Q L, Zeng D C, Li G S, Liu Y G. CRISPR-GE: a convenient software toolkit for CRISPR-based genome editing. Mol Plant, 2017, 10: 1246-1249.
doi: 10.1016/j.molp.2017.06.004 |
| [25] | 曾栋昌, 马兴亮, 谢先荣, 祝钦泷, 刘耀光. 植物CRISPR/ Cas9多基因编辑载体构建和突变分析的操作方法. 中国科学: 生命科学, 2018, 48: 783-794. |
| Zeng D C, Ma X L, Xie X R, Zhu Q L, Liu Y G. A protocol for CRISPR/Cas9-based multi-gene editing and sequence decoding of mutant sites in plants. Sci Sin (Vitae), 2018, 48: 783-794. (in Chinese with English abstract) | |
| [26] |
Zhang Y, Su J B, Duan S, Ao Y, Dai J R, Liu J, Wang P, Li Y G, Liu B, Feng D R, Wang J F, Wang H B. A highly efficient rice green tissue protoplast system for transient gene expression and studying light/chloroplast-related processes. Plant Methods, 2011, 7: 30.
doi: 10.1186/1746-4811-7-30 pmid: 21961694 |
| [27] |
Ding B, Bellizzi M D R, Ning Y S, Meyers B C, Wang G L. HDT701, a histone H4 deacetylase, negatively regulates plant innate immunity by modulating histone H4 acetylation of defense-related genes in rice. Plant Cell, 2012, 24: 3783-3794.
doi: 10.1105/tpc.112.101972 |
| [28] |
Pan X Q, Welti R, Wang X M. Quantitative analysis of major plant hormones in crude plant extracts by high-performance liquid chromatography-mass spectrometry. Nat Prot, 2010, 5: 986-992.
doi: 10.1038/nprot.2010.37 |
| [29] |
Hui W K, Wang Y, Yan S J, Shi J F, Huang W J, Zayed M Z, Peng C C, Chen X Y, Wu G J. Simultaneous analysis of endogenous plant growth substances during floral sex differentiation in Jatropha curcas L. using HPLC-ESI-MS/MS. Sci Hortic (Amsterdam), 2018, 241: 209-217.
doi: 10.1016/j.scienta.2018.06.086 |
| [30] |
Zhao J H, Zhang W, Da S J, Liu X C, Duan J. Rice histone deacetylase HDA704 positively regulates drought and salt tolerance by controlling stomatal aperture and density. Planta, 2021, 254: 79.
doi: 10.1007/s00425-021-03729-7 pmid: 34542712 |
| [31] |
Park C J, Han S W, Chen X, Ronald P C. Elucidation of XA21- mediated innate immunity. Cell Microbiol, 2010, 12: 1017-1025.
doi: 10.1111/j.1462-5822.2010.01489.x |
| [32] |
Son S, An H K, Seol Y J, Park S R, Im J H. Rice transcription factor WRKY114 directly regulates the expression of OsPR1a and chitinase to enhance resistance against Xanthomonas oryzae pv. oryzae. Biochem Biophys Res Commun, 2020, 533: 1262-1268.
doi: 10.1016/j.bbrc.2020.09.141 |
| [33] |
Wang G N, Ding X H, Yuan M, Qiu D Y, Li X H, Xu C G, Wang S P. Dual function of rice OsDR8 gene in disease resistance and thiamine accumulation. Plant Mol Biol, 2006, 60: 437-449.
doi: 10.1007/s11103-005-4770-x |
| [34] | 赵慧. 水稻耐旱性调控网络关键调节基因的克隆及OsERF65的功能研究. 华中农业大学硕士学位论文, 湖北武汉, 2020. |
| Zhao H. Cloning of Key Regulatory Genes in Rice Drought Tolerance Regulatory Network and Functional Study of OsERF65. MS Thesis of Huazhong Agricultural University, Wuhan, Hubei, China, 2020. (in Chinese with English abstract) | |
| [35] |
Lata C, Prasad M. Role of DREBs in regulation of abiotic stress responses in plants. J Exp Bot, 2011, 62: 4731-4748.
doi: 10.1093/jxb/err210 pmid: 21737415 |
| [36] |
Assmann S M, Wang X Q. From milliseconds to millions of years: guard cells and environmental responses. Curr Opin Plant Biol, 2001, 4: 421-428.
pmid: 11597500 |
| [1] | 王懿涵, 李富昌, 刘意, 朱国鹏. 甘薯IbOPR2基因启动子克隆及调控因子的筛选[J]. 作物学报, 2026, 52(4): 1268-1276. |
| [2] | 陈伟, 卫万娟, 赵其兵, 常东伟, 余凌波, 翟鹏飞, 冯志明, 陈宗祥, 任仰涛, 杨鹏, 刘海浪, 李珍富, 杨永乐, 金彦刚, 左示敏. 利用CRISPR/Cas9编辑Hd6基因创制优质早熟水稻新种质[J]. 作物学报, 2026, 52(4): 1046-1056. |
| [3] | 张清怡, 肖义涛, 李秋霞, 张钰石, 张明才, 李召虎. 渗透胁迫下不同玉米品种幼苗ABA合成及生理生化响应差异[J]. 作物学报, 2026, 52(1): 221-232. |
| [4] | 张建鹏, 王国瑞, 别海, 叶飞宇, 马晨晨, 梁小菡, 鲁晓民, 尚霄丽, 曹丽茹. 转录因子ZmMYB153通过ABA信号调节气孔运动增强玉米苗期抗旱性[J]. 作物学报, 2025, 51(7): 1827-1837. |
| [5] | 凤舞剑, 冼晓青, 张新钵, 曹丹, 强承魁. 基于转录组和AlphaFold对稻瘟菌经典效应蛋白和水稻受体的快速鉴定[J]. 作物学报, 2025, 51(6): 1480-1488. |
| [6] | 雷松翰, 范骏扬, 车艳奕, 代永东, 郑雨萌, 田维江, 桑贤春, 王晓雯. 水稻内卷叶突变体acl3的鉴定及调控基因的功能分析[J]. 作物学报, 2025, 51(6): 1467-1479. |
| [7] | 黄梦欣, 庄灵玲, 程佩佩, 李秦, 徐建堂, 陶爱芬, 方平平, 祁建民, 张立武. 黄麻U6启动子克隆及其转录活性分析[J]. 作物学报, 2025, 51(5): 1156-1165. |
| [8] | 沈文杰, 陈晴晴, 胡逸群, 张爱芳, 张曼玉. 安徽省不同生理小种稻瘟病菌对稻瘟灵的敏感性研究[J]. 作物学报, 2025, 51(5): 1338-1346. |
| [9] | 陆雯佳, 汪军成, 姚立蓉, 张宏, 司二静, 杨轲, 孟亚雄, 李葆春, 马小乐, 王化俊. 大麦PRX基因家族全基因组鉴定及其干旱胁迫下的表达分析[J]. 作物学报, 2025, 51(5): 1198-1214. |
| [10] | 曹晓晴, 祁显涛, 刘昌林, 谢传晓. 编辑ZmCCT10、ZmCCT9、ZmGhd7基因的串联DsRed荧光表达盒的CRISPR/Cas9系统的构建及验证[J]. 作物学报, 2024, 50(8): 1961-1970. |
| [11] | 黄淑贤, 刘荣, 李冠, 疏琴, 徐斐, 宗绪晓, 杨涛. 通过CRISPR/Cas9建立豌豆基因组大片段敲除体系[J]. 作物学报, 2024, 50(7): 1658-1668. |
| [12] | 折萌, 郑登俞, 柯照, 吴忠义, 邹华文, 张中保. 玉米ZmGRAS13基因的克隆及功能研究[J]. 作物学报, 2024, 50(6): 1420-1434. |
| [13] | 万应春, 班义结, 蒋钰东, 王亚欣, 刘晶晶, 刘晓晴, 程育林, 王楠, 冯萍. 水稻雄性不育突变体tpa1的表型鉴定与精细定位[J]. 作物学报, 2024, 50(5): 1104-1114. |
| [14] | 毛燕, 郑名敏, 牟成香, 谢吴兵, 唐琦. 渗透胁迫下玉米自然反义转录本cis-NATZmNAC48启动子的功能分析[J]. 作物学报, 2024, 50(2): 354-362. |
| [15] | 武丽芬, 夏川, 张立超, 孔秀英, 陈景堂, 刘旭. TaEMF2调控小麦抽穗期的功能分析[J]. 作物学报, 2024, 50(12): 2940-2949. |
|
||