欢迎访问作物学报,今天是
作物学报 ›› 2026, Vol. 52 ›› Issue (10): 2875-2885.doi: 10.3724/SP.J.1006.2026.64047
崔一凡( ), 孙晓彤, 石瑛()
Cui Yi-Fan(), Sun Xiao-Tong, Shi Ying()
摘要:
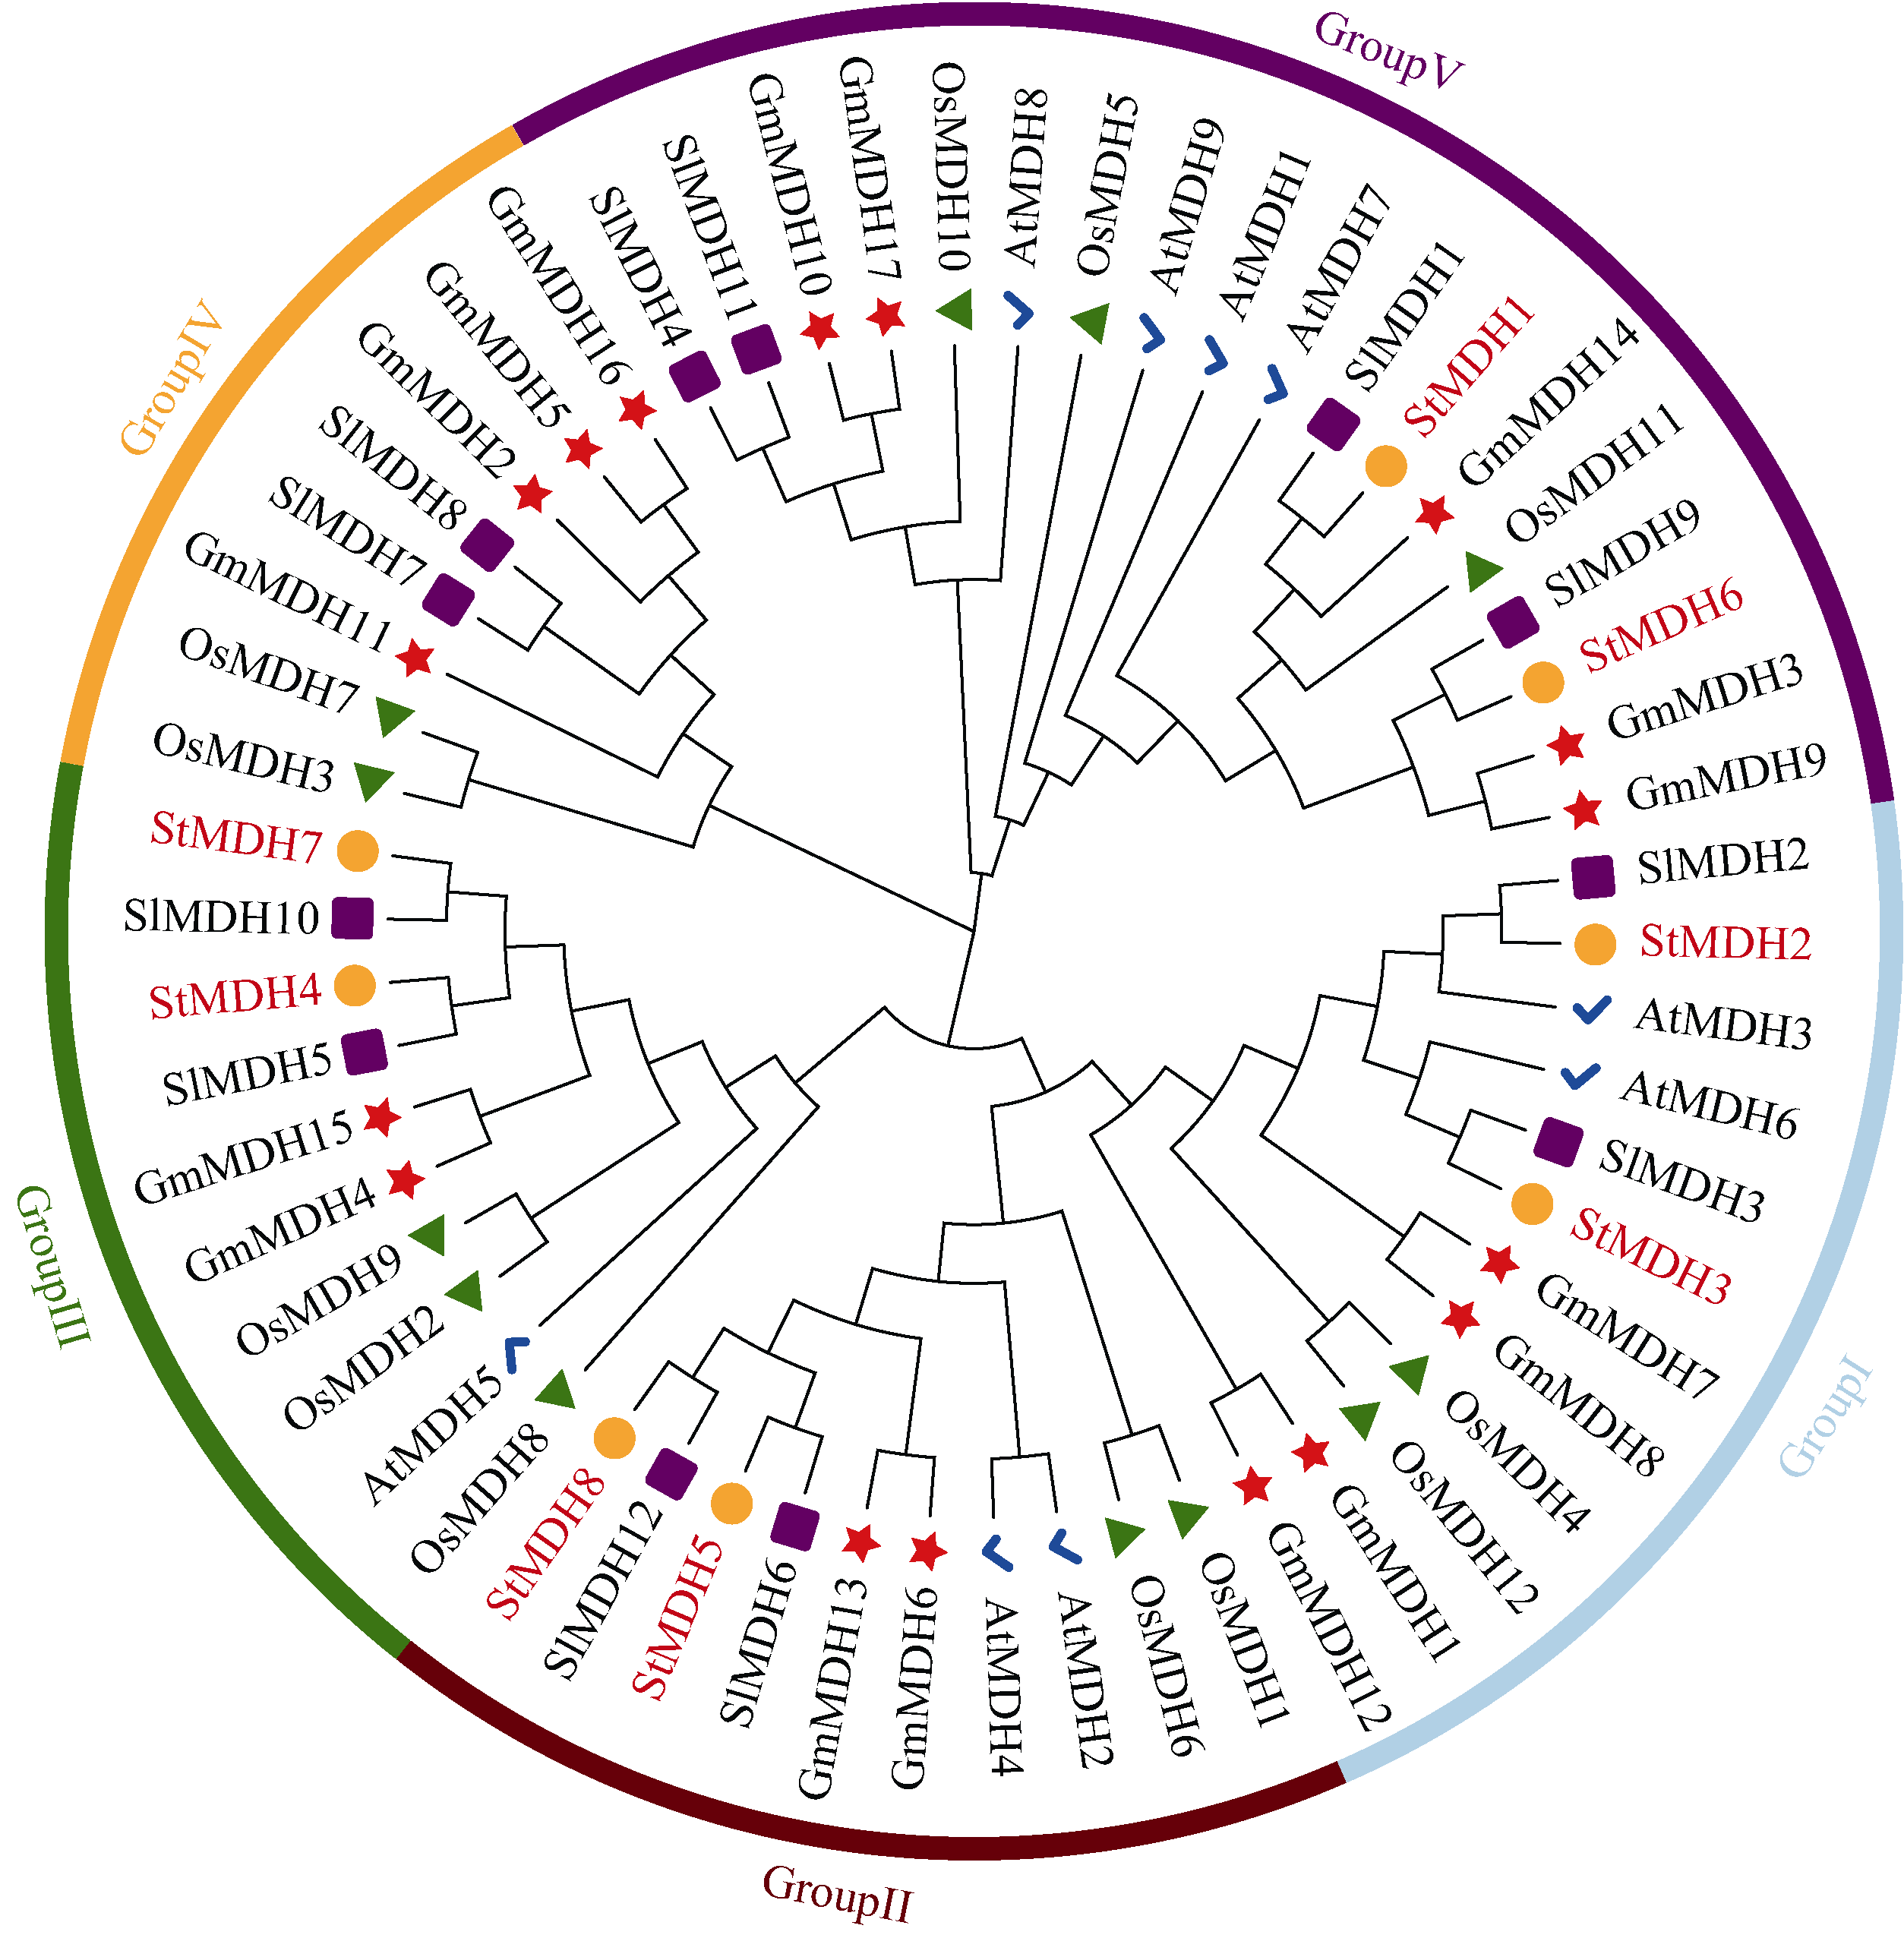
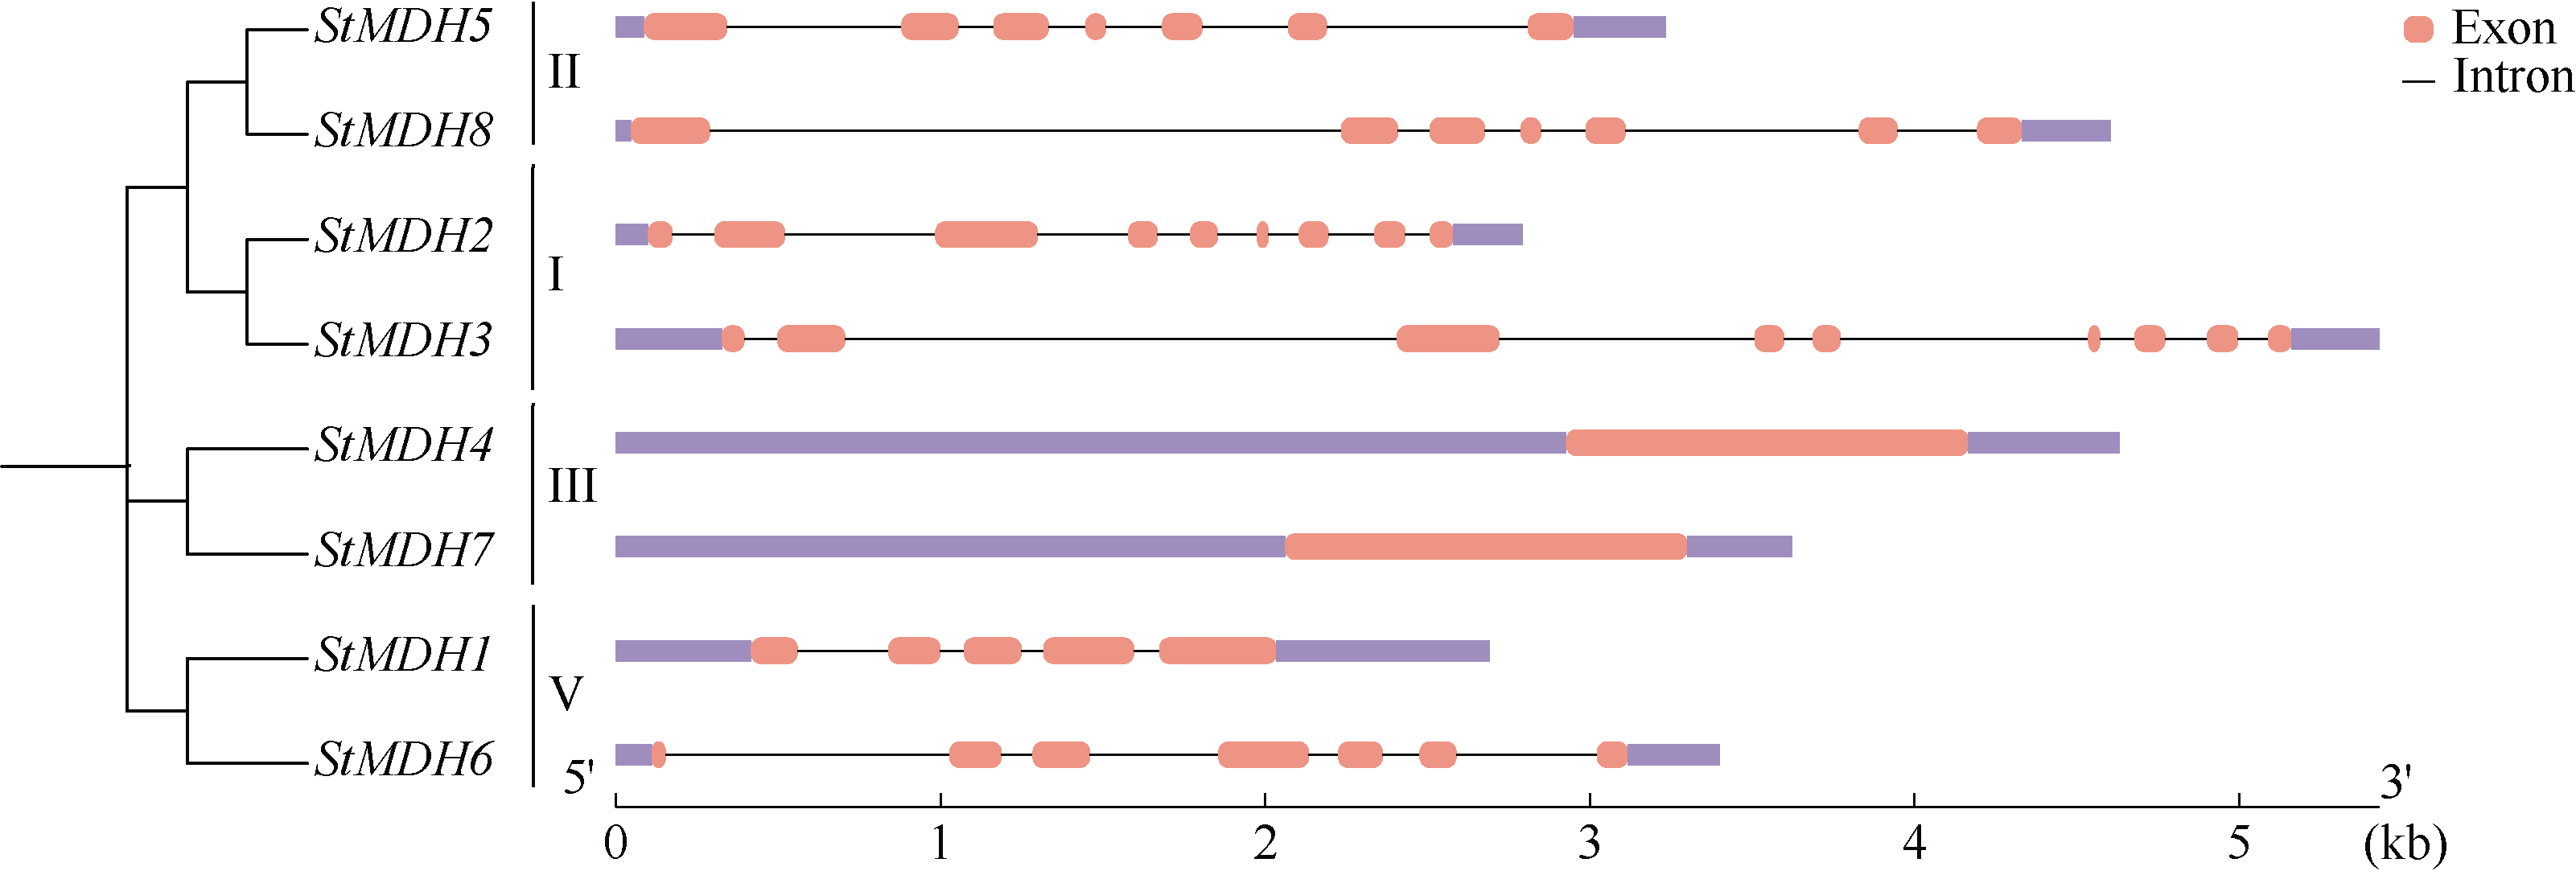
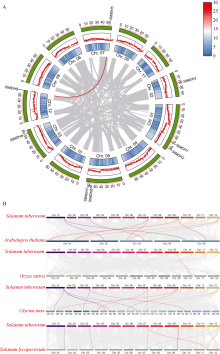
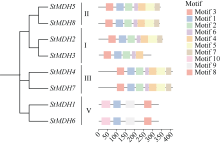
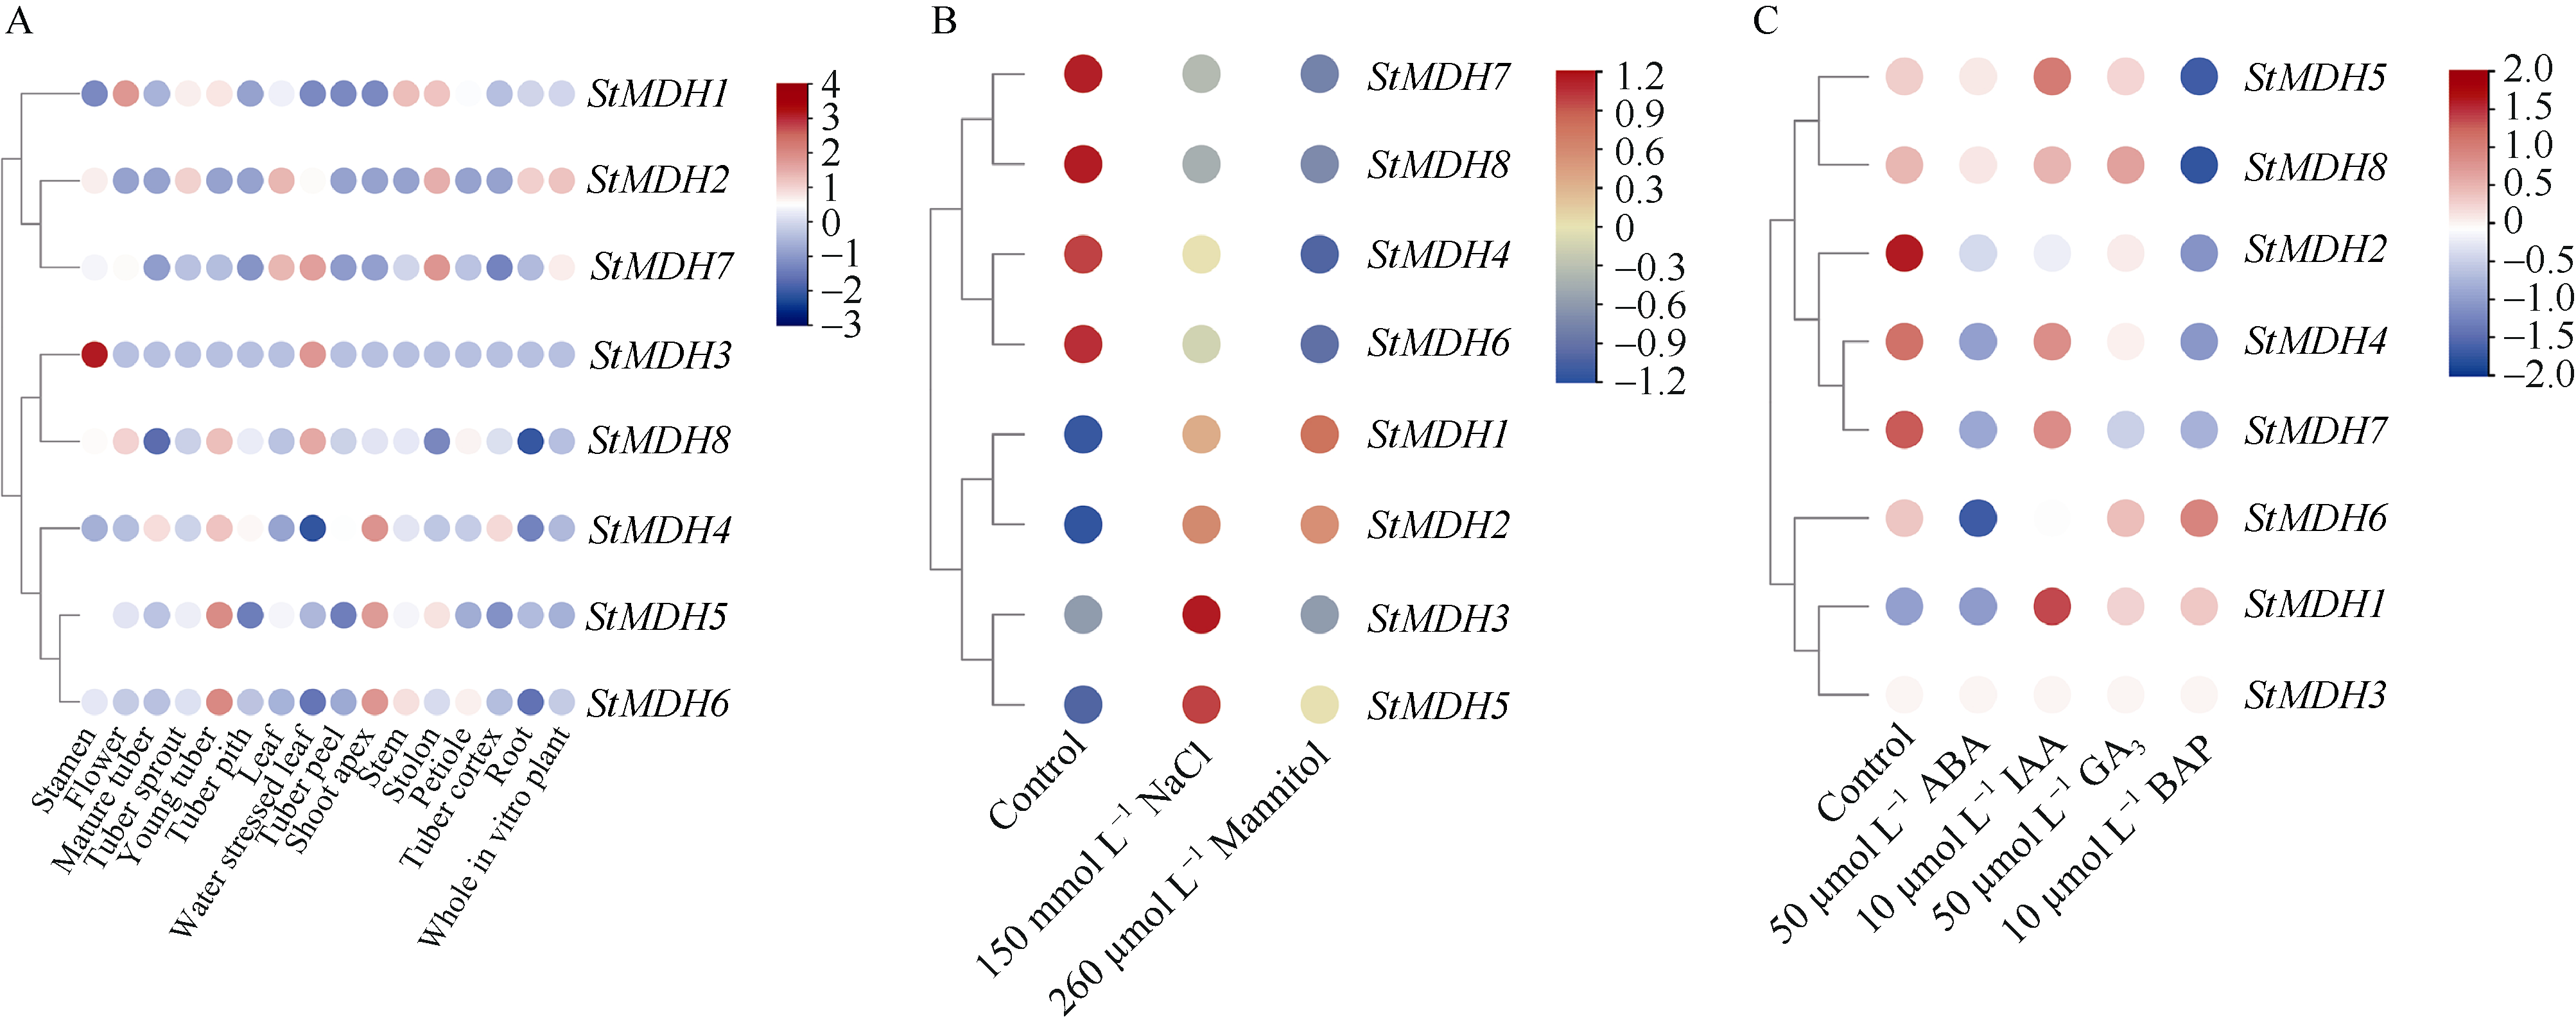
苹果酸脱氢酶(MDH; EC1.1.1.37)广泛存在于植物中, 能利用还原型烟酰胺腺嘌呤二核苷酸或还原型烟酰胺腺嘌呤二核苷酸磷酸催化苹果酸与草酰乙酸之间的转化, 参与三羧酸循环过程, 同时参与调控植物的生长发育及逆境响应等多种生理过程。本研究采用生物信息学方法, 在马铃薯基因组中鉴定出8个MDH家族成员, 依据染色体位置被命名为StMDH1~StMDH8, 并进一步将其划分为5个亚家族。理化性质分析显示, StMDHs编码蛋白的分子量介于30.11~43.85 kD之间, 等电点范围为5.91~9.00; 亚细胞定位预测表明, 这些蛋白主要分布于叶绿体和线粒体中。基因结构分析发现, 同一亚家族成员具有相似的外显子数目和保守的Motif组成。基于公开转录组数据的表达谱分析显示, 多数StMDHs基因对非生物胁迫及激素处理均有响应, 其中StMDH2对盐胁迫表现出最为显著的诱导表达模式。进一步通过酿酒酵母异源表达体系验证, StMDH2的过表达能够显著提高酵母细胞的耐盐性。本研究丰富了马铃薯MDH基因家族的理论认知, 为马铃薯抗逆分子育种提供了潜在的基因资源和候选靶点。
| [1] |
Liu N, Zhao R M, Qiao L, et al. Growth stages classification of potato crop based on analysis of spectral response and variables optimization. Sensors, 2020, 20: 3995.
doi: 10.3390/s20143995 |
| [2] |
Faried H N, Ayyub C M, Wattoo F M, et al. Assessing salt tolerance induction in potato by salicylic acid using morpho-physio- biochemical, ionic, and yield indices. Potato Res, 2022, 65: 677-691.
doi: 10.1007/s11540-021-09539-4 |
| [3] |
Machado M F, Prioli A J, Mangolin C A. Malate dehydrogenase (MDH; EC1.1.1.37) isozymes in tissues and callus cultures of Cereus peruvianus (Cactaceae). Biochem Genet, 1993, 31: 167-172.
pmid: 8363555 |
| [4] |
Scheibe R. Malate valves to balance cellular energy supply. Physiol Plant, 2004, 120: 21-26
doi: 10.1111/j.0031-9317.2004.0222.x pmid: 15032873 |
| [5] |
Gietl C. Malate dehydrogenase isoenzymes: cellular locations and role in the flow of metabolites between the cytoplasm and cell organelles. Biochim Biophys Acta Bioenerg, 1992, 1100: 217-234.
doi: 10.1016/0167-4838(92)90476-T |
| [6] |
Selinski J, König N, Wellmeyer B, et al. The plastid-localized NAD-dependent malate dehydrogenase is crucial for energy homeostasis in developing Arabidopsis thaliana seeds. Mol Plant, 2014, 7: 170-186.
doi: 10.1093/mp/sst151 |
| [7] |
Miller S S, Driscoll B T, Gregerson R G, et al. Alfalfa malate dehydrogenase (MDH): molecular cloning and characterization of five different forms reveals a unique nodule-enhanced MDH. Plant J, 1998, 15: 173-184.
doi: 10.1046/j.1365-313x.1998.00192.x pmid: 9721676 |
| [8] |
Baird L M, Berndsen C E, Monroe J D. Malate dehydrogenase in plants: evolution, structure, and a myriad of functions. Essays Biochem, 2024, 68: 221-233.
doi: 10.1042/EBC20230089 |
| [9] |
Huang J J, Niazi A K, Young D, et al. Self-protection of cytosolic malate dehydrogenase against oxidative stress in Arabidopsis. J Exp Bot, 2018, 69: 3491-3505.
doi: 10.1093/jxb/erx396 |
| [10] |
Beeler S, Liu H C, Stadler M, et al. Plastidial NAD-dependent malate dehydrogenase is critical for embryo development and heterotrophic metabolism in Arabidopsis. Plant Physiol, 2014, 164: 1175-1190.
doi: 10.1104/pp.113.233866 |
| [11] |
Tomaz T, Bagard M, Pracharoenwattana I, et al. Mitochondrial malate dehydrogenase lowers leaf respiration and alters photorespiration and plant growth in Arabidopsis. Plant Physiol, 2010, 154: 1143-1157.
doi: 10.1104/pp.110.161612 |
| [12] | Talla S K, Sunil B, Rao D E, et al. Redox basis of photosynthesis inhibition at supra-optimal bicarbonate in mesophyll protoplasts of Arabidopsis thaliana. J Plant Physiol, 2023, 287: 154047. |
| [13] | Yokochi Y, Yoshida K, Hahn F, et al. Redox regulation of NADP-malate dehydrogenase is vital for land plants under fluctuating light environment. Proc Natl Acad Sci USA, 2021, 118: e2016903118. |
| [14] |
Chen Y Q, Fu Z Y, Zhang H, et al. Cytosolic malate dehydrogenase 4 modulates cellular energetics and storage reserve accumulation in maize endosperm. Plant Biotechnol J, 2020, 18: 2420-2435.
doi: 10.1111/pbi.v18.12 |
| [15] |
Teng X, Zhong M S, Zhu X P, et al. FLOURY ENDOSPERM16 encoding a NAD-dependent cytosolic malate dehydrogenase plays an important role in starch synthesis and seed development in rice. Plant Biotechnol J, 2019, 17: 1914-1927.
doi: 10.1111/pbi.v17.10 |
| [16] |
Kandoi D, Mohanty S, Tripathy B C. Overexpression of plastidic maize NADP-malate dehydrogenase (ZmNADP-MDH) in Arabidopsis thaliana confers tolerance to salt stress. Protoplasma, 2018, 255: 547-563.
doi: 10.1007/s00709-017-1168-y |
| [17] |
Tesfaye M, Temple S J, Allan D L, et al. Overexpression of malate dehydrogenase in transgenic alfalfa enhances organic acid synthesis and confers tolerance to aluminum. Plant Physiol, 2001, 127: 1836-1844.
pmid: 11743127 |
| [18] |
Shi Y H, Feng J H, Wang L P, et al. OsMDH12: a peroxisomal malate dehydrogenase regulating tiller number and salt tolerance in rice. Plants, 2023, 12: 3558.
doi: 10.3390/plants12203558 |
| [19] |
Jiang M, Chen Z, Ansah E O, et al. Rice NADP-dependent malate dehydrogenase gene OsMDH8.2 is involved in heat tolerance. Fundam Res, 2025, 5: 2037-2044.
doi: 10.1016/j.fmre.2023.12.010 |
| [20] |
Nan N, Wang J, Shi Y J, et al. Rice plastidial NAD-dependent malate dehydrogenase 1 negatively regulates salt stress response by reducing the vitamin B6 content. Plant Biotechnol J, 2020, 18: 172-184.
doi: 10.1111/pbi.13184 pmid: 31161713 |
| [21] |
Wang Z A, Li Q, Ge X Y, et al. The mitochondrial malate dehydrogenase 1 gene GhmMDH1 is involved in plant and root growth under phosphorus deficiency conditions in cotton. Sci Rep, 2015, 5: 10343.
doi: 10.1038/srep10343 |
| [22] |
Li Z Q, Shi L, Lin X J, et al. Genome-wide identification and expression analysis of malate dehydrogenase gene family in sweet potato and its two diploid relatives. Int J Mol Sci, 2023, 24: 16549.
doi: 10.3390/ijms242316549 |
| [23] |
Song J L, Zou X Y, Liu P D, et al. Differential expressions and enzymatic properties of malate dehydrogenases in response to nutrient and metal stresses in Stylosanthes guianensis. Plant Physiol Biochem, 2022, 170: 325-337.
doi: 10.1016/j.plaphy.2021.12.012 |
| [24] |
Zhou R N, Wang S H, Liu P Y, et al. Genome-wide characterization of soybean malate dehydrogenase genes reveals a positive role for GmMDH2 in the salt stress response. J Integr Agric, 2025, 24: 2492-2510.
doi: 10.1016/j.jia.2023.12.036 |
| [25] |
Zhang Y H, Wang Y L, Sun X M, et al. Genome-wide identification of MDH family genes and their association with salt tolerance in rice. Plants, 2022, 11: 1498.
doi: 10.3390/plants11111498 |
| [26] | Imran M, Tang K, Liu J Y. Comparative genome-wide analysis of the malate dehydrogenase gene families in cotton. PLoS One, 2016, 11: e0166341. |
| [27] | Letunic I, Khedkar S, Bork P. SMART: recent updates, new developments and status in 2020. Nucleic Acids Res, 2021, 49: D458-D460. |
| [28] |
Bailey T L, Boden M, Buske F A, et al. MEME SUITE: tools for motif discovery and searching. Nucleic Acids Res, 2009, 37: W202-W208.
doi: 10.1093/nar/gkp335 |
| [29] |
Liu W Z, Xie Y B, Ma J Y, et al. IBS: an illustrator for the presentation and visualization of biological sequences. Bioinformatics, 2015, 31: 3359-3361.
doi: 10.1093/bioinformatics/btv362 pmid: 26069263 |
| [30] |
Nakashima K, Yamaguchi-Shinozaki K. ABA signaling in stress-response and seed development. Plant Cell Rep, 2013, 32: 959-970.
doi: 10.1007/s00299-013-1418-1 pmid: 23535869 |
| [31] |
Ohme-Takagi M, Shinshi H. Ethylene-inducible DNA binding proteins that interact with an ethylene-responsive element. Plant Cell, 1995, 7: 173-182.
doi: 10.1105/tpc.7.2.173 pmid: 7756828 |
| [32] |
Jores T, Tonnies J, Wrightsman T, et al. Synthetic promoter designs enabled by a comprehensive analysis of plant core promoters. Nat Plants, 2021, 7: 842-855.
doi: 10.1038/s41477-021-00932-y pmid: 34083762 |
| [33] |
Ma B Q, Yuan Y Y, Gao M, et al. Genome-wide identification, classification, molecular evolution and expression analysis of malate dehydrogenases in apple. Int J Mol Sci, 2018, 19: 3312.
doi: 10.3390/ijms19113312 |
| [1] | 张芮嘉, 吕建禹, 高源, 王浩宇, 王宇琦, 姜佳宁, 赵健雄, 王雪贺缘, 贺琳. 玉米ZmDREB53转录因子通过清除活性氧正调控植物的耐盐性[J]. 作物学报, 2026, 52(9): 2660-2670. |
| [2] | 赵海洋, 郭徐鹏, 罗杨, 杨钢, 蔡振良, 胡赞民, 陈宇红, 范成明, 张新永. 柠檬酸锌对作物耐盐能力及土壤电导率的调控[J]. 作物学报, 2026, 52(9): 2792-2808. |
| [3] | 吴张晶, 李世贵, 马俊, 张宁, 司怀军. 马铃薯淀粉含量相关SSR标记的遗传多样性分析及综合评价[J]. 作物学报, 2026, 52(8): 2509-2520. |
| [4] | 崔庆晗, 栗锦烨, 董亚瑞, 孙春燕, 贾玉鑫. 马铃薯单倍体种质资源的创制[J]. 作物学报, 2026, 52(7): 1966-1974. |
| [5] | 姜存仓, 窦佳艺, 鲁克嵩, 肖思赟, 刘冰, 毕嘉榆. 硼对作物盐胁迫的缓解效应及其机制研究进展[J]. 作物学报, 2026, 52(7): 1929-1942. |
| [6] | 马晨铭, 哈斯图亚, 常泓博, 梁擎天, 游乐, 吴尚蓉. 基于叶绿素荧光成像系统的马铃薯叶片叶绿素含量估测[J]. 作物学报, 2026, 52(7): 2193-2206. |
| [7] | 陈国欢, 张锐, 李艳迪, 赵佳琪, 任湧涛, 张天赐, 郭华春, 李俊, 杨芳. 外源硒叶面喷施对浅紫色马铃薯块茎花青素合成的影响[J]. 作物学报, 2026, 52(6): 1876-1890. |
| [8] | 王文辕, 燕雪嘉, 刘玉霖, 孙晓彤, 李亚楠, 唐鑫华, 石瑛. 耐弱光马铃薯品种筛选及转录因子编码基因StPIF3的克隆与功能分析[J]. 作物学报, 2026, 52(6): 1631-1645. |
| [9] | 邹仪妹, 徐敏, 汪海洋, 姚辉, 王加峰, 刘浩, 任代胜. 两系不育系水稻幼苗根系响应盐胁迫的转录因子调控网络鉴定[J]. 作物学报, 2026, 52(6): 1728-1742. |
| [10] | 宋裕祯, Bheel Chander Kumar, 王跃, 张颖星, 郭娟, Khound Rituraj, Santra Dipak Kumar, 曹晓宁, 王瑞云. 糜子AP2亚家族全基因组鉴定及PmAP2-1和PmAP2-9耐盐功能分析[J]. 作物学报, 2026, 52(4): 1127-1139. |
| [11] | 田立涛, 丁宁, 王树林, 齐恩芳, 张荣, 王蕊蕊, 马利雯, 李建武, 杨江伟. 马铃薯Argonaute基因家族鉴定及晚疫病诱导表达分析[J]. 作物学报, 2026, 52(4): 1116-1126. |
| [12] | 汪玲, 胡好, 宋家凤, 程洁蓝, 陈颖, 郑婷婷, 吕钊彦, 朱晓彪, 侯华兰. 马铃薯UDP-糖基转移酶基因StUGT52的克隆及功能验证[J]. 作物学报, 2026, 52(3): 665-676. |
| [13] | 张宇, 刘芳, 蔡诚诚, 杨小华, 吉阿么石扎, 杨元军, 王西瑶. 溴乙烷与赤霉素协同处理破除马铃薯块茎休眠的机理初探[J]. 作物学报, 2026, 52(3): 825-838. |
| [14] | 覃奕琰, 付瑶, 苏畅, 李娜, 徐静茹, 程笑然, 张琪, 赵明辉. OsST41调控水稻苗期耐盐性的功能分析[J]. 作物学报, 2026, 52(3): 802-812. |
| [15] | 刘吉昌, 李思烨, 李雪婷, 王洪章, 刘鹏, 张吉旺, 赵斌, 任佰朝, 任昊. 盐胁迫对不同耐盐型夏玉米品种根系生长及养分吸收效率的影响[J]. 作物学报, 2026, 52(2): 565-577. |
|
||