欢迎访问作物学报,今天是

作物学报 ›› 2018, Vol. 44 ›› Issue (04): 493-504.doi: 10.3724/SP.J.1006.2018.00493

• 作物遗传育种·种质资源·分子遗传学 • 上一篇    下一篇

玉米光合突变体hcf136 (high chlorophyll fluorescence 136)的转录组分析

吴庆飞1,**(), 秦磊1,**(), 董雷2, 丁泽红3, 李平华1,*(), 杜柏娟1,*()   

  1. 1 山东农业大学农学院, 山东泰安271018
    2 河南农业大学农学院, 河南郑州450002
    3 中国热带农业科学院热带生物技术研究所, 海南海口571101
  • 收稿日期:2017-03-27 接受日期:2018-01-08 出版日期:2018-01-30 网络出版日期:2018-01-30
  • 通讯作者: 吴庆飞,秦磊,李平华,杜柏娟
  • 作者简介:

    作者简介: 吴庆飞, E-mail: feiqw1234@163.com, Tel: 0538-8242995; 秦磊, E-mail: qinlei2012shandong@163.com, Tel: 0538-8242995

  • 基金资助:
    本研究由国家自然科学基金项目(31271393)资助

Transcriptome Analysis on a Maize Photosynthetic Mutant hcf136 (high chlorophyll fluorescence 136)

Qing-Fei WU1,**(), Lei QIN1,**(), Lei DONG2, Ze-Hong DING3, Ping-Hua LI1,*(), Bai-Juan DU1,*()   

  1. 1 College of Agronomy, Shandong Agricultural University, Tai’an 271018, Shandong, China;
    2 College of Agronomy, Henan Agricultural University, Zhengzhou 450002, Henan, China
    3 Institute of Tropical Bioscience and Biotechnology, Chinese Academy of Tropical Agricultural Science, Haikou 571101, Hainan, China
  • Received:2017-03-27 Accepted:2018-01-08 Published:2018-01-30 Published online:2018-01-30
  • Contact: Qing-Fei WU,Lei QIN,Ping-Hua LI,Bai-Juan DU
  • Supported by:
    This study was supported by the National Natural Science Foundation of China (31271393).

摘要:

玉米是典型的C4作物, 其光合作用由花环结构的两种细胞(叶肉细胞和维管束鞘细胞)共同完成。玉米hcf136 (high chlorophyll fluorescence 136)突变体叶肉细胞叶绿体不能形成基粒从而丧失了PSII活性, 但维管束鞘细胞的叶绿体发育不受影响, 是研究玉米C4光合机理的好材料。本研究利用转录组测序(RNA-Seq)技术, 通过对高光和低光下野生型和hcf136突变体不同叶片部位进行转录组分析发现, PSII相关基因的转录未发生明显差异, 表明PSII复合体的缺失是非转录水平变化所引起。此外, 突变体中淀粉合成受阻, 糖降解、糖转运及Cu2+转运等代谢过程加剧, 且一些转录因子表达发生显著变化。该结果对进一步深入研究玉米HCF136基因的功能提供了参考。

关键词: 玉米, hcf136突变体, RNA-Seq, C4光合

Abstract:

Maize (Zea mays) is a typical C4 plant, which photosynthetic activities are partitioned by the cooperating of Kranz anatomy—mesophyll (M) cell and bundle sheath (BS) cell. The maize high chlorophyll fluorescence 136 (hcf136) mutant is an ideal material for C4 photosynthesis study, due to it lacks PSII activity without normal thylakoid grana in M chloroplasts. However, the development of BS chloroplasts is not affected. In this study, we utilized RNA-Seq technology to monitor the transcriptome changes in different leaf sections between wild type and hcf136 mutant under different light intensities. The results indicated that the impairment of PSII is not caused by the transcription changes of PSII related genes. We also noticed that the starch biosynthesis was blocked in the mutant; and the sugar degradation, sugar transport and copper ion transport were triggered. In addition, the expression level of transcription factors was changed distinctly. These results provide valuable information for understanding a comprehensive function of HCF136 gene in future.

Key words: Zea mays, high chlorophyll fluorescence 136 mutant, RNA-Seq, C4 photosynthesis

图1

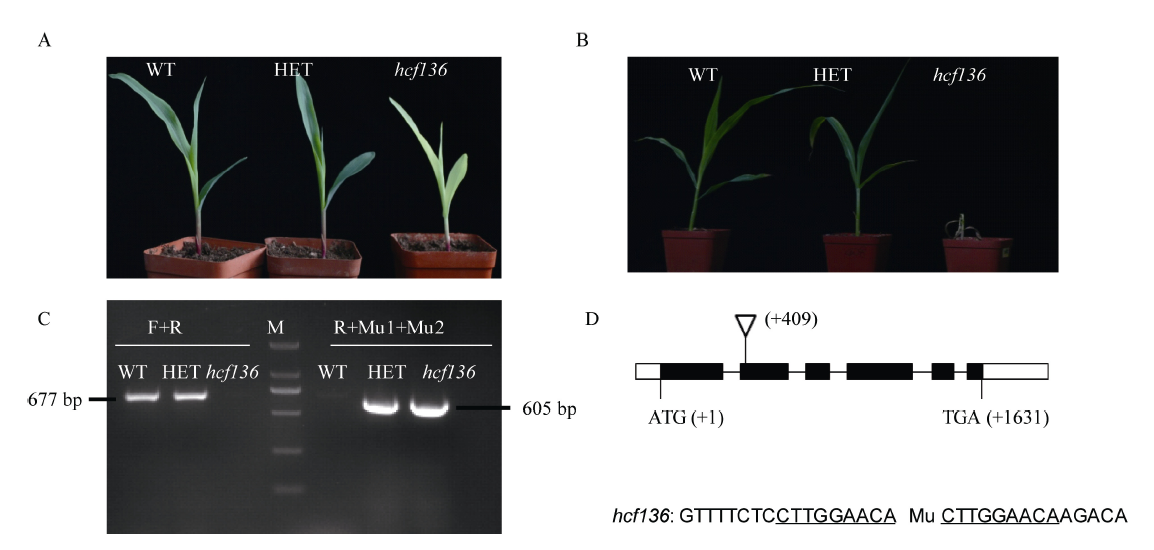
hcf136突变体的表型及基因型鉴定 A: 种植8 d后的玉米幼苗, WT代表野生型, HET代表杂合体, hcf136为突变体; B: 种植17 d后的幼苗; C: hcf136突变体的PCR鉴定, 用HCF136基因特异引物(F, R)与Mutator特异引物(Mu1, Mu2)进行PCR, M为DL2000 marker; D: Mu转座子的插入位置。下画线部分为插入造成的9 bp正向重复序列。"

表1

hcf136突变体光合参数"

材料
Material
胞间CO2浓度
Ci
蒸腾速率
E
气孔导度
Gs
净光合速率
Pn
叶绿素a的含量
Ca (mg L-1)
叶绿素b的含量
Cb (mg L-1)
野生型WT 182.56±16.38 1.54±0.12 159±16.38 14.80±1.67 28.54±1.77 14.21±3.78
杂合体HET 175.72±20.25 1.46±0.10 161±14.63 14.57±1.42 27.92±2.53 12.35±4.62
突变体hcf136 373.61±36.57* 0.67±0.22* 62±25.21* -2.34±1.29* 15.48±3.36* 5.61±0.86*

图2

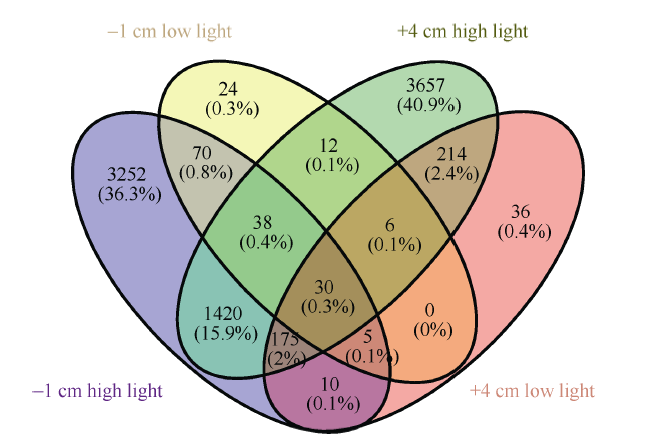
不同光照下不同叶片部位差异表达的基因数目"

表2

野生型和突变体植株中显著差异表达的基因"

基因编号
Gene ID
基因注释
Gene annotation
差异倍数 Fold of differentiation
-1 cm高光
-1 cm high light
-1 cm低光
-1 cm low light
+4 cm高光
+4 cm high light
+4 cm低光
+4 cm low light
GRMZM2G119865 EREB25 3.395 5.868 4.895 5.507
GRMZM2G416701 EREB81 -1.121 0.386 -2.032 0.006
GRMZM2G035502 DHAR2 -1.052 -0.609 -1.722 -0.590
GRMZM2G152777 GDSL-like Lipase super family -6.103 -3.297 -4.868 -1.597
GRMZM2G036966 GeBP15 -4.058 -2.808 -6.100 -5.987
GRMZM2G102838 HCF136 -2.635 -1.989 -1.005 -0.101
GRMZM2G175782 NAC 036 -0.997 -2.026 -4.821 -2.077
GRMZM2G065105 novel plant snare 11 1.400 2.243 2.305 5.053
GRMZM2G077837 PEX11 family -2.096 -1.119 -2.364 -0.932
GRMZM2G440605 SERPIN family -4.433 -3.536 -4.030 -1.765
GRMZM2G014055 TH7 -3.021 -4.203 -4.390 -3.148
GRMZM2G320298 α/β-Hydrolases super family 2.852 2.902 6.346 6.103
GRMZM5G848603 α/β-Hydrolases super family -1.411 -0.193 -2.830 0.020
GRMZM2G019018 Unknown -1.615 -2.612 -2.580 -2.172
GRMZM2G038570 Unknown 2.631 2.820 3.442 4.732
GRMZM2G100568 Unknown -2.655 -4.581 -4.803 -2.601
GRMZM2G103108 Unknown 4.154 5.141 4.077 5.266
GRMZM2G126900 Unknown 3.570 2.071 6.321 4.916
GRMZM2G130173 Unknown -3.533 -1.656 -1.454 -0.961
GRMZM2G134020 Unknown -3.388 -3.906 -4.870 -1.959
GRMZM2G140998 Unknown -0.885 -0.505 -1.155 -0.425
GRMZM2G152808 Unknown -0.755 -0.500 -2.393 -0.318
GRMZM2G156422 Unknown -2.033 -0.869 -3.605 -0.505
GRMZM2G161761 Unknown -4.532 -4.261 -5.043 -1.752
GRMZM2G307258 Unknown 2.870 4.177 5.357 6.317
GRMZM2G338406 Unknown 3.774 8.907 4.928 6.966
GRMZM2G430807 Unknown -2.359 -2.589 -3.808 -1.547
GRMZM2G473480 Unknown -2.406 0.586 -3.956 -0.926
GRMZM5G844094 Unknown -3.144 -12.202 -2.588 -2.947
GRMZM5G879789 Unknown -3.293 -1.208 -2.215 -1.200

表3

不同条件下差异表达基因的上调或下调数量"

不同组分
Different component
高光
High light
低光
Low light
高光和低光
High light and low light
-1 cm上调 -1 cm up-regulated 2979 70 60
-1 cm下调 -1 cm down-regulated 2021 115 41
+4 cm上调 +4 cm up-regulated 2838 347 272
+4 cm下调 +4 cm down-regulated 2714 129 117

图3

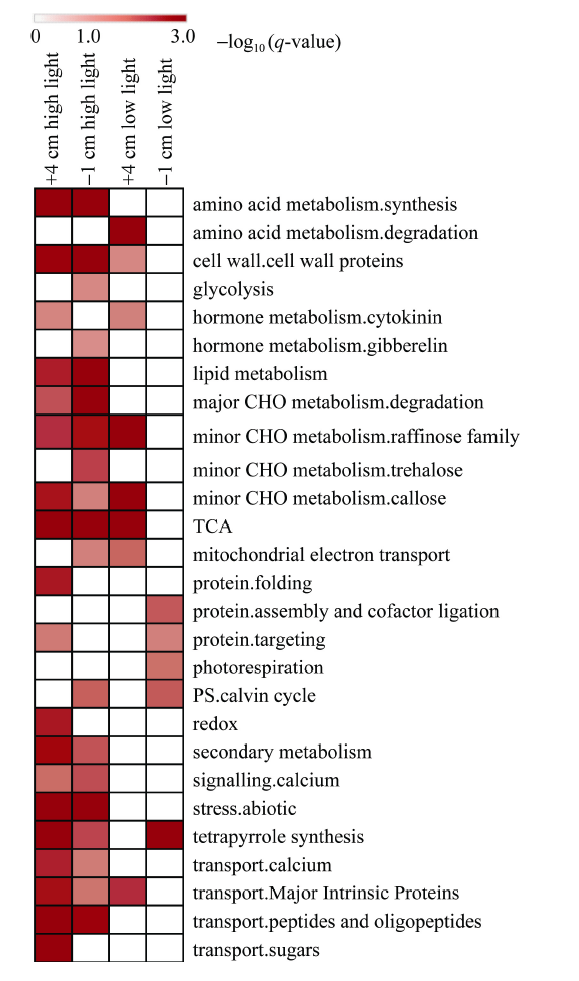
差异表达基因功能富集热图红色表示被富集的功能途径, 红色越深代表被富集的越显著。"

表4

光合相关基因的表达变化"

基因编号
Gene ID
基因注释
Gene annotation
差异倍数Fold of differentiation
-1 cm高光
-1 cm high light
-1 cm低光
-1 cm low light
+4 cm高光
+4 cm high light
+4 cm低光
+4 cm low light
GRMZM2G027955 APL2 0.363 0.014 -3.367 -0.712
GRMZM2G038335 ATL43 0.466 1.610 6.382 3.383
GRMZM2G055973 ATL5D 0.202 1.122 1.990 2.388
GRMZM5G803981 BAM6 -0.701 0.242 7.007 5.671
GRMZM2G035749 BMY8 2.264 3.059 3.913 2.411
GRMZM2G144782 CHYR1 1.399 1.730 3.491 3.889
GRMZM2G118737 CINV2 2.171 1.315 3.114 3.273
GRMZM2G170842 CINV2 1.900 1.495 4.975 3.865
GRMZM2G316136 CIPK1 0.177 -1.274 -3.614 -0.607
GRMZM2G412601 CIPK6 -2.724 1.050 -5.620 -0.632
GRMZM2G129399 Cu2+ transporter family 2.224 2.597 7.007 5.671
GRMZM2G092427 CP24 -1.268 1.812 1.223 0.921
GRMZM2G018798 DRIP2 1.574 1.353 3.985 4.302
GRMZM2G102838 HCF136 -2.635 -1.989 -1.005 -0.101
GRMZM2G107402 HEMA1 1.354 1.848 3.799 2.464
GRMZM2G092311 LHCA1 -0.452 1.233 0.342 1.112
GRMZM2G072280 LHCA2 -0.022 1.221 0.560 0.742
GRMZM2G160268 LHCA4 -0.821 1.270 0.318 1.076
GRMZM2G018627 LHCB2 -1.017 1.355 -0.778 1.679
GRMZM2G057281 LHCB3 -2.182 2.157 0.622 1.146
GRMZM2G033885 LHCB4 -1.523 1.234 0.073 1.189
GRMZM2G056270 MIEL1 0.884 0.851 1.419 2.535
GRMZM2G085019 NADP-ME 2.017 0.731 1.749 2.936
GRMZM2G463280 PRK 0.144 0.970 1.614 2.304
GRMZM2G016066 PSAE -0.828 1.610 0.273 1.321
GRMZM2G358180 PSBC 1.273 -2.181 1.263 -0.430
GRMZM5G831399 PSBH -0.391 -0.792 1.472 0.186
GRMZM2G113349 PSBO2 -0.358 1.042 1.063 1.448
GRMZM2G175562 PSBO2 -0.914 -0.302 -1.147 0.748
GRMZM5G870219 PsbQ-like 2 -0.061 0.929 0.768 1.382
GRMZM5G804323 QA -0.181 0.960 -0.524 1.436
GRMZM2G440259 RING/U-box super family 0.362 1.663 4.823 2.293
GRMZM2G127147 RS6 1.815 2.503 4.575 3.283
GRMZM2G440605 SERPIN1 -4.433 -3.536 -4.030 -1.765
GRMZM2G399484 SET7/9 family 1.659 1.377 6.716 4.757
GRMZM2G037265 SIP1 2.568 1.687 5.697 4.360
基因编号
Gene ID
基因注释
Gene annotation
差异倍数Fold of differentiation
-1 cm高光
-1 cm high light
-1 cm低光
-1 cm low light
+4 cm高光
+4 cm high light
+4 cm低光
+4 cm low light
GRMZM2G050177 SIP1 2.227 2.731 4.181 3.938
GRMZM2G050273 SIP1 1.597 1.929 4.194 4.096
GRMZM2G311756 SIP2 2.095 0.026 0.963 1.656
GRMZM2G010349 STN7 0.733 0.625 0.431 1.823
GRMZM2G701201 STN8 -0.394 1.410 0.638 1.336
GRMZM2G160460 sugar transporter family 2.639 0.955 4.748 3.755
GRMZM2G372297 TAP38 0.692 0.543 -0.052 1.396
GRMZM2G389118 TOC159 0.637 0.852 2.614 3.502
GRMZM2G123277 TPS7 1.995 0.794 3.352 3.394
GRMZM2G120674 UBC2 0.985 1.273 2.416 2.546

图4

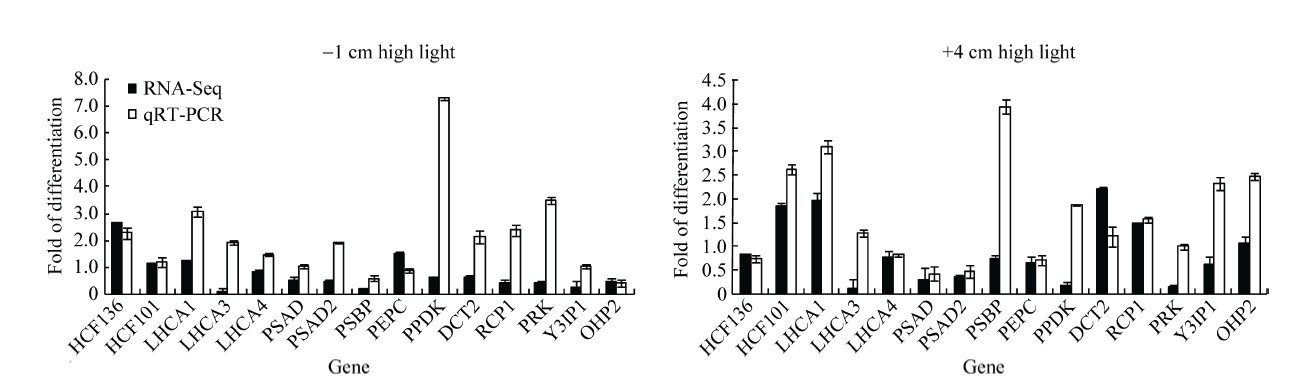
RNA-Seq与qRT-PCR结果比较 Fold of differentiation代表log2 (突变体表达量/野生型表达量)。"

表5

野生型及突变体转录因子表达比较"

基因编号
Gene ID
基因注释
Gene annotation
差异倍数Fold of differentiation
-1 cm高光
-1 cm high light
-1 cm低光
-1 cm low light
+4 cm高光
+4 cm high light
+4 cm低光
+4 cm low light
GRMZM2G119865 EREB25 3.395 5.868 4.895 5.507
GRMZM2G416701 EREB81 -1.121 0.386 -2.032 0.006
GRMZM2G390641 ARF21 -2.515 1.222 -1.175 0.441
GRMZM2G030710 ARF24 0.523 0.488 -0.654 0.263
GRMZM2G145146 bHLH107 -1.942 1.531 0.450 2.132
GRMZM2G083504 bHLH121 -1.198 1.049 -1.339 0.186
GRMZM2G144275 bHLH136 -0.999 0.794 -1.633 0.319
GRMZM2G479885 bZIP39 -1.030 1.001 -1.996 0.247
GRMZM2G311665 C3H20 -1.447 1.247 -2.148 -0.910
GRMZM2G426154 EMB2219 1.397 0.681 0.784 0.919
GRMZM2G457562 EREB113 -0.211 0.335 8.063 5.344
GRMZM2G421033 EREB156 -1.105 3.042 2.755 3.012
GRMZM2G119865 EREB25 3.395 58.418 4.895 5.507
GRMZM2G031983 GATA21 -2.090 0.577 -2.982 -0.184
GRMZM2G036966 GBP15 -4.058 0.143 -6.100 -9.310
GRMZM2G036966 GeBP15 -4.058 -2.808 -6.100 -2.467
GRMZM2G026833 GLK1 -1.780 1.072 -1.934 0.114
GRMZM2G056600 HB120 -2.236 0.706 -3.776 -0.039
GRMZM2G137046 HY5 -0.400 1.143 2.085 2.266
GRMZM2G044902 LBD6 0.993 1.143 2.556 2.376
GRMZM2G078820 MYB158 -2.055 0.609 -0.700 2.263
GRMZM2G048136 MYB59 0.376 0.665 -2.822 -0.298
GRMZM2G049378 MYBR115 -1.092 -1.268 -4.646 -2.738
GRMZM2G175782 NAC 36 -1.034 -2.033 -4.821 -2.081
GRMZM2G114850 NAC1 1.014 3.187 2.749 2.706
GRMZM2G167018 NAC110 -0.046 1.303 -0.666 -0.054
基因编号
Gene ID
基因注释
Gene annotation
差异倍数Fold of differentiation
-1 cm高光
-1 cm high light
-1 cm低光
-1 cm low light
+4 cm高光
+4 cm high light
+4 cm低光
+4 cm low light
GRMZM2G127379 NAC25 5.827 2.426 8.537 4.905
GRMZM5G898290 NAC40 -0.827 0.612 -1.000 -0.273
GRMZM2G162739 NAC5 0.588 1.387 4.264 3.045
GRMZM2G155370 Orphan28 -1.049 1.049 0.054 -1.533
GRMZM2G350711 Orphan307 0.301 1.242 2.251 3.453
GRMZM2G016756 PIL5 -1.352 1.159 -5.544 -0.196
GRMZM2G065374 PIL6 -0.267 0.539 -1.561 0.101
GRMZM2G023872 RGA1 6.869 1.363 9.580 7.073
GRMZM2G046816 TUB3 0.056 0.152 -2.410 0.116
GRMZM2G064775 ZIM29 8.189 4.106 10.844 3.384
[1] Furbank R T, Hatch M D.Mechanism of C4 photosynthesis: the size and composition of the inorganic carbon pool in bundle sheath cells.Plant Physiol, 1987, 85: 958-964
[2] Hatch M D.C4 photosynthesis: a unique blend of modified biochemistry, anatomy and ultrastructure.Biochim Biophy Acta, 1987, 895: 81-106
[3] Edwards G E, Franceschi V R, Ku M S, Voznesenskaya E V, Pyankov V I, Andreo C S.Compartmentation of photosynthesis in cells and tissues of C4 plants.J Exp Bot, 2001, 52: 577-590
[4] Majeran W, Friso G, Ponnala L, Connolly B, Huang M, Reidel E.Structural and metabolic transitions of C4 leaf development and differentiation defined by microscopy and quantitative proteomics in maize.Plant Cell, 2010, 22: 3509-3542
[5] Gregory R P, Droppa M, Horváth G, Evans E H.A comparison based on delayed light emission and fluorescence induction of intact chloroplasts isolated from mesophyll protoplasts and bundle-sheath cells of maize.Biochem J, 1979, 180: 253-256
[6] Takabayashi A, Kishine M, Asada K, Endo T, Sato F.Differential use of two cyclic electron flows around photo-system I for driving CO2-concentration mechanism in C4 photosynthesis.Proc Natl Acad Sci USA, 2005, 102: 16898-16903
[7] Richard R A.Selectable traits to increase crop photosynthesis and yield of grain crops.J Exp Bot, 2000, 51: 447-458
[8] Zhu X G, Long S P, Ort D R.What is the maximum efficiency with which photosynthesis can convert solar energy into biomass.Curr Opin Biotechnol, 2008, 19: 153-159
[9] Stern D B, Hanson M R, Barkan A.Genetics and genomics of chloroplast biogenesis: maize as a model system.Trends Plant Sci, 2004, 9: 293-301
[10] 李保珠, 赵孝亮, 彭雷. 植物叶绿体发育及调控研究进展. 植物学报, 2014, 49: 337-345
Li B Z, Zhao X L, Peng L.Research advances in the development and regulation of plant chloroplasts.Chin Bull Bot, 2014, 49: 337-345 (in Chinese with English abstract)
[11] Belcher S, Williams-Carrier R, Stiffler N, Barkan A.Large-scale genetic analysis of chloroplast biogenesis in maize.Biochim Biophys Acta, 2015, 1847: 1004-1016
[12] Covshoff S, Majeran W, Liu P, Kolkman J M, van Wijk K J, Brutnell T P. Deregulation of maize C4 photosynthetic development in a mesophyll cell-defective mutant.Plant Physiol, 2008, 146: 1469-1481
[13] Plucken H, Muller B, Grohmann D, Westhoff P, Eichacker L A.The HCF136 protein is essential for assembly of the photosystem II reaction center in Arabidopsis thaliana. FEBS Lett, 2002, 532: 85-90
[14] Schuster S C.Next-generation sequencing transforms today’s biology.Nat Methods, 2008, 5: 16-18
[15] Chang Y M, Liu W Y, Shi A C, Shen M N, Lu C H, Lu M Y.Characterizing regulatory and functional differentiation between maize mesophyll and bundle sheath cells by transcriptomic analysis.Plant Physiol, 2012, 160: 165-177
[16] John C R, Smith-Unna R D, Woodfield H, Covshoff S, Hibberd J M. Evolutionary convergence of cell-specific gene expression in in-dependent lineages of C4 grasses.Plant Physiol, 2014, 165: 62-75
[17] Tausta S L, Li P, Si Y T, Gandotra N, Liu P, Sun Q.Developmental dynamics of Kranz cell transcriptional specificity in maize leaf reveals early onset of C4-related processes. J Exp Bot, 2014, 65: 3543-3555
[18] 江芳, 丁泽红, 董雷, 李平华. 玉米光合突变体bsd2 (bundle sheath defective II)的转录组分析. 植物生理学报, 2016, 52: 1214-1222
Jiang F, Ding Z H, Dong L, Li P H.Transcriptome analysis on the maize photosynthetic mutant bsd2 (bundle sheath defective II). Plant Physiol J, 2016, 52: 1214-1222 (in Chinese with English abstract)
[19] Porra R J.The chequered history of the development and use of simultaneous equations for the accurate determination of chlorophyll a and b. Photosynth Res, 2002, 73: 149-156
[20] Wang L, Si Y, Dedow L K, Shao Y, Liu P, Brutnell T P.A low cost library construction protocol and data analysis pipeline for Illumina-based strand-specific multiplex RNA-seq.PLoS One, 2011, 6: e26426
[21] Robinson M D, McCarthy D J, Smyth G K. Edge R: a bioconductor package for differential expression analysis of digital gene expression data.Bioinformatics, 2010, 26: 139-140
[22] Li P, Ponnala L, Gandotra N, Wang L, Si Y, Tausta S L, Kebrom T H, Provart N, Patel R, Brutnell T P.The developmental dynamics of the maize leaf transcriptome.Nat Genet, 2010, 42: 1060-1067
[23] Suresh V K, Tellabati M, Nelli R K, White G A, Perez B B, Sebastian S, Slomka M J, Brown I H, Stephen P D, Kin C C.18S rRNA is a reliable normalisation gene for real time PCR based on influenza virus infected cells.Virl J, 2012, 9: 230
[24] Yruela I, Montoya G, Picorel R.The inhibitory mechanism of Cu(II) on the photosystem II electron transport from higher plants.Photosynth Res, 1992, 33: 227-233
[25] Ouzounidou G, Mousbakas M, Karataglis S.Responses of maize (Zea mays L.) plants to copper stress: IR growth, mineral content and ultrastructure of roots. Environ Exp Bot, 1995, 2: 167-176
[26] Meurer J, Plücken H, Kowallik K V, Westhoff P.A nuclear-encoded protein of prokaryotic origin is essential for the stability of photosystem II in Arabidopsis thaliana. EMBO J, 1998, 17: 5286-5297
[27] Maxwell K, Johnson G N.Chlorophyll fluorescence: a practical guide.J Exp Bot, 2000, 51: 659-668
[28] Meurer J, Meierhoff K, Westhoff P.Isolation of high-chlorophyll- fluorescence mutants of Arabidopsis thaliana and their characterization by spectroscopy, immunoblotting and Northern hybridization.Planta, 1996, 198: 385-396
[29] Varotto C, Pesaresi P, Maiwald D.Identification of photosynthetic mutants of Arabidopsis by automatic screening for altered effective quantum yield of photosystem II.Photosynthetica, 2000, 38: 497-504
[1] 刘恩波, 陈静, 李红星, 于宁宁, 任佰朝, 赵斌, 刘鹏, 张吉旺. 遮阴改变源-库平衡和调节碳水化合物代谢进而抑制夏玉米幼穗发育[J]. 作物学报, 2026, 52(6): 1891-1901.
[2] 梁进宇, 尹嘉德, 王红丽, 张国平, 侯慧芝, 董博, 马明生. 基于无人机高光谱和机器学习的旱地饲用玉米叶片氮含量估测[J]. 作物学报, 2026, 52(6): 1788-1801.
[3] 孙淑凤, 许振南, 黄嘉鑫, 翁建峰, 李新海. 玉米MAPK家族全基因组鉴定及其对拟轮枝镰孢菌感染的响应[J]. 作物学报, 2026, 52(5): 1291-1308.
[4] 张宁宁, 滕雨菲, 任娜娜, 魏兴卓, 闫书豪, 樊可心, 王永宏, 陈文康, 张兴华, 朱万超, 徐淑兔, 薛吉全. 201份玉米自交系抗旱表型评价及可塑性分析[J]. 作物学报, 2026, 52(5): 1309-1325.
[5] 杨欣雨, 崔文涛, 迪力尼格尔·阿力木, 汪凯翔, 吴鹏昊, 任姣姣. 玉米穗上叶片数全基因组关联分析和全基因组选择[J]. 作物学报, 2026, 52(5): 1573-1590.
[6] 韩亚鑫, 何冠华, 张小琼, 张登峰, 李永祥, 刘旭洋, 王天宇, 黎裕, 邹华文, 李春辉. 基于RNA-Seq和BSA-Seq联合分析挖掘玉米侧根密度基因资源[J]. 作物学报, 2026, 52(5): 1341-1352.
[7] 张鸿蓉, 王菲儿, 李盼, 仇海龙, 朱静, 赵连豪, 南运有, 何蔚, 樊志龙, 胡发龙, 柴强, 殷文. 减量20%灌水与25%有机肥替代化肥提高青贮玉米产量的光合特性[J]. 作物学报, 2026, 52(5): 1487-1500.
[8] 杨扬, 常诗惠, 田红丽, 易红梅, 王璐, 任洁, 范亚明, 刘亚维, 王凤格, 赵久然. 不同生态区国审玉米品种的遗传多样性分析[J]. 作物学报, 2026, 52(5): 1352-1364.
[9] 蔡宏玮, 于爱忠, 姜科强, 王鹏飞, 王玉珑, 霍建喆, 庞小能, 尹波, 尚永盼. 干旱灌区有机肥替代部分化肥促进甜玉米产量提升的关键机制[J]. 作物学报, 2026, 52(4): 1166-1180.
[10] 田红丽, 杨扬, 范亚明, 易红梅, 郭丹丹, 王凤格, 赵久然. 适于玉米品种鉴定的一套三等位变异SNP新型标记组合[J]. 作物学报, 2026, 52(4): 993-1005.
[11] 杨亚莉, 徐明睿, 马越飞, 海艺蕊, 刘凯栋, 刘万茂, 孙颖. 玉米根尖及整根响应缺铁的转录组比较研究[J]. 作物学报, 2026, 52(4): 1006-1021.
[12] 张超, 郭欢, 李忠玲, 岳淑宁, 赵娜. 基于BSA-seq技术定位玉米籽粒花青素关联基因[J]. 作物学报, 2026, 52(3): 780-789.
[13] 郭向阳, 涂亮, 王栋, 刘鹏飞, 王安贵, 易强, 任洪, 李刚, 祝云芳, 吴迅, 蒋喻林, 田丰, 陈泽辉. 热带Suwan种质在我国玉米种质改良中的创新与利用[J]. 作物学报, 2026, 52(3): 655-664.
[14] 孟成, 王哲. 玉米ZmPFK基因家族全基因组鉴定及响应胁迫表达分析[J]. 作物学报, 2026, 52(3): 764-779.
[15] 李新浩, 邢梦柯, 周梓惠, 李思烨, 任昊, 王洪章, 赖华江. 外源褪黑素通过协调光反应与暗反应增强玉米苗期的耐热性[J]. 作物学报, 2026, 52(3): 839-856.
Viewed
Full text


Abstract

Cited

  Shared   
  Discussed   
No Suggested Reading articles found!