欢迎访问作物学报,今天是
作物学报 ›› 2022, Vol. 48 ›› Issue (7): 1601-1613.doi: 10.3724/SP.J.1006.2022.14130
李旭娟1( ), 李纯佳1, 吴转娣1, 田春艳1, 胡鑫1, 丘立杭2, 吴建明2, 刘新龙1,*()
LI Xu-Juan1(), LI Chun-Jia1, WU Zhuan-Di1, TIAN Chun-Yan1, HU Xin1, QIU Li-Hang2, WU Jian-Ming2, LIU Xin-Long1,*()
摘要:
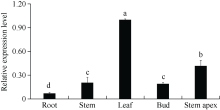
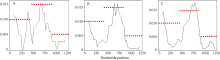
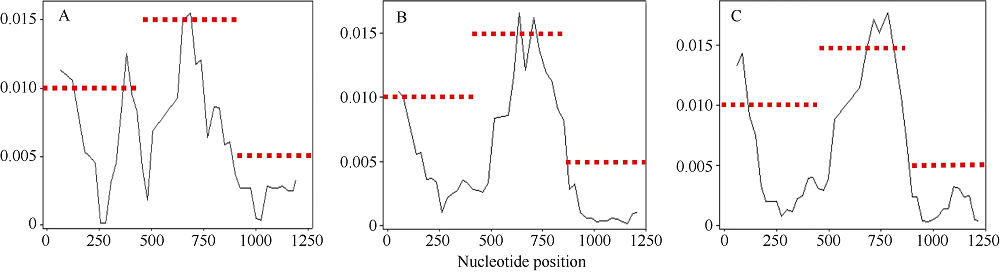
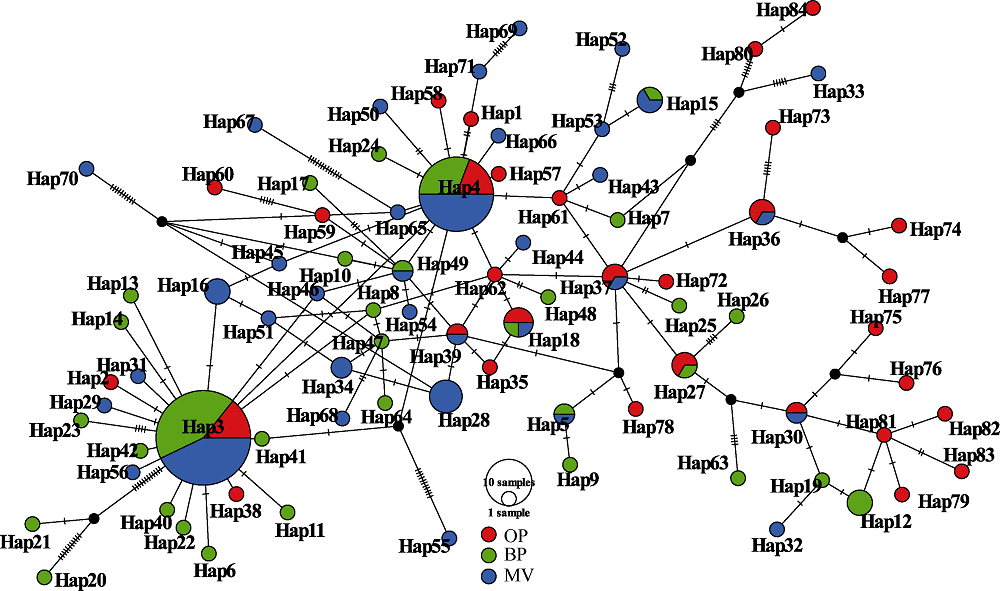
分蘖是无性繁殖经济作物-甘蔗最重要的农艺性状之一, 挖掘分蘖关键基因用于甘蔗理想株型调控是增加品种产量的重要途径。本研究使用实时荧光定量PCR技术对前期从甘蔗中获得的与水稻分蘖关键基因HTD2高度同源的ScHTD2基因开展表达特征分析, 然后探讨其在甘蔗种质资源群体中的基因多态性情况, 筛选与分蘖性状相关的变异位点。结果显示, 该基因表达具有组织特异性, 在叶中表达最高; 腋芽萌动发育过程中, 在休眠芽中表达量最高, 随着蔗芽萌动, 开始显著下调表达, 负调控蔗芽的萌动发育; 植物激动素、生长素和独脚金内酯都能显著诱导该基因在萌动蔗芽和蔗苗分蘖芽中的表达, 结合激素处理的表型变化特征, 预示生长素和独脚金内酯诱导该基因的高表达会抑制萌动蔗芽的继续发育和延迟蔗苗的分蘖, 但植物激动素诱导的高表达并没有这种抑制效应。对从26份甘蔗种质资源中获得的520条HTD2基因组DNA克隆序列开展基因多态性分析表明, 在基因组结构上, 该基因具有2个外显子和1个内含子, 其中内含子区域变异最为丰富。从群体基因多态性看, 原始种亲本群体在外显子1和2区域表现出较高的核苷酸多样性, 而主栽品种群体在内含子区域表现出较高的核苷酸多样性。从编码区单倍型多样性来看, 原始种亲本群体间单倍型多样性最为丰富, 其次为主栽品种群体。基因选择性测验中, 原始种亲本群体受正向选择, 选择压力较大, 基因进化速度快, 而骨干亲本群体和主栽品种群体受负向选择, 向纯化方向发展。编码区单倍型演化分析表明, Hap3和Hap4处于单倍型演化的辐射中心, 属于较为原始的类型。基因编码区变异位点与分蘖率相关性检测揭示该基因有23个SNP位点和5个InDel位点不同变异类型剂量与甘蔗种质资源分蘖率呈显著相关, 变异类型剂量效应将是未来甘蔗分子辅助育种重要的关注点。研究为进一步深入解析甘蔗分蘖调控关键基因的功能作用和开发功能性标记奠定了重要基础。
| [1] | Pribil M, Hermann S R, Dun G D, Karno Ngo C, O’Neill S, Wang L, Bonnett G D, Chandler P M, Beveridge C A, Lakshmanan P. Altering sugarcane shoot architecture through genetic engineering:prospects for increasing cane and sugar yield. In: Proceedings of the 2007 Conference of the Australian Society of Sugar Cane Technologists. Cairns, Queensland, Australia: Australian Society of Sugar Cane Technologists, 2007. pp 251-257. |
| [2] |
Vasantha S, Shekinah D E, Gupta C, Rakkiyappan P. Tiller production, regulation and senescence in sugarcane (Saccharum species hybrid) genotypes. Sugar Technol, 2012, 14: 156-160.
doi: 10.1007/s12355-011-0129-6 |
| [3] |
Liu W Z, Chao W, Fu Y P, Hu G C, Si H M, Zhu L, Luan W J, He Z Q, Sun Z X. Identification and characterization of HTD2: a novel gene negatively regulating tiller bud outgrowth in rice. Planta, 2009, 230: 649-658.
doi: 10.1007/s00425-009-0975-6 |
| [4] |
Gao Z Y, Qian Q, Liu X H, Yan M X, Feng Q, Dong G J, Liu J, Han B. Dwarf 88, a novel putative esterase gene affecting architecture of rice plant. Plant Mol Biol, 2009, 71: 265-276.
doi: 10.1007/s11103-009-9522-x |
| [5] |
Zhou F, Lin Q B, Zhu L H, Ren Y L, Zhou K N, Shabek N, Wu F Q, Mao H B, Dong W, Gan L, Ma W W, Gao H, Chen J, Yang C, Wang D, Tan J J, Zhang X, Guo X P, Wang J L, Jiang L, Liu X, Chen W Q, Chu J F, Yan C Y, Ueno K, Ito S, Asami T, Cheng Z J, Wang J, Lei C, Zhai H Q, Wu C Y, Wang H Y, Zheng N, Wan J M. D14-SCFD3-dependent degradation of D53 regulates strigolactone signalling. Nature, 2013, 504: 406-410.
doi: 10.1038/nature12878 |
| [6] | 吕爱丽, 李旭娟, 刘洪博, 吴才文, 曾千春, 刘新龙. 甘蔗ScHTD2基因的克隆及生物信息学分析. 热带作物学报, 2016, 37: 1133-1140. |
| Lyu A L, Li X J, Liu H B, Wu C W, Zeng Q C, Liu X L. Cloning and bioinformatics analysis of full-Length cDNA sequence of ScHTD2 gene from sugarcane. Chin J Trop Crops, 2016, 37: 1133-1140. (in Chinese with English abstract) | |
| [7] | 陈迪文, 黄莹, 卢颖林, 江永, 李奇伟. 不同营养液配方对甘蔗组培幼苗生长的影响. 广东农业科学, 2013, 40(21): 28-31. |
| Chen D W, Huang Y, Lu Y L, Jiang Y, Li Q W. Effect of different nutrient solutions on the growth of sugarcane tissue culture seedlings. Guangdong Agric Sci, 2013, 40(21): 28-31. (in Chinese with English abstract) | |
| [8] |
Ling H, Wu Q B, Guo J L, Xu L P, Que Y X. Comprehensive selection of reference genes for gene expression normalization in sugarcane by real time quantitative RT-PCR. PLoS One, 2014, 9: e97469.
doi: 10.1371/journal.pone.0097469 |
| [9] |
McIntyre C L, Jackson M, Cordeiro G M, Amouyal O, Hermann S, Aitken K S, Eliott F, Henry R J, Casu R E, Bonnett G D. The identification and characterisation of alleles of sucrose phosphate synthase gene family III in sugarcane. Mol Breed, 2006, 18: 39-50.
doi: 10.1007/s11032-006-9012-7 |
| [10] |
Zhang J, Arro J, Chen Y Q, Ming R. Haplotype analysis of sucrose synthase gene family in three Saccharum species. BMC Genomics, 2013, 14: 314.
doi: 10.1186/1471-2164-14-314 |
| [11] |
Kumar S, Stecher G, Tamura K. MEGA7: molecular evolutionary genetics analysis version 7.0 for bigger datasets. Mol Biol Evol, 2016, 33: 1870-1874.
doi: 10.1093/molbev/msw054 |
| [12] |
Librado P, Rozas J. DnaSP v5: a software for comprehensive analysis of DNA polymorphism data. Bioinformatics, 2009, 25: 1451-1452.
doi: 10.1093/bioinformatics/btp187 pmid: 19346325 |
| [13] |
Leigh J W, Bryant D. PopART: full-feature software for haplotype network construction. Methods Ecol Evol, 2015, 6: 1110-1116.
doi: 10.1111/2041-210X.12410 |
| [14] |
张洪映, 毛新国, 景蕊莲, 谢惠民, 昌小平. 小麦TaPK7基因单核苷酸多态性与抗旱性的关系. 作物学报, 2008, 34: 1537-1543.
doi: 10.3724/SP.J.1006.2008.01537 |
|
Zhang H Y, Mao X G, Jing R L, Xie H M, Chang X P. Relationship between single nucleotide polymorphism of TaPK7 gene and drought tolerance in wheat. Acta Agron Sin, 2008, 34: 1537-1543. (in Chinese with English abstract)
doi: 10.3724/SP.J.1006.2008.01537 |
|
| [15] | 俎鲁霞, 徐国恒. tRNA的结构、功能及合成简介. 生物学通报, 2008, 43(1): 19-20. |
| Zu L X, Xu G H. Introduction to the structure, function and synthesis of tRNA. Bull Biol, 2008, 43(1): 19-20. | |
| [16] |
Arite T, Umehara M, Ishikawa S, Hanada A, Maekawa M, Yamaguchi S, Kyozuka J. d14, a strigolactone-insensitive mutant of rice, shows an accelerated outgrowth of tillers. Plant Cell Physiol, 2009, 50: 1416-1424.
doi: 10.1093/pcp/pcp091 |
| [17] |
Abe S, Sado A, Tanaka K, Kisugi T, Asami K, Ota S, Kim H I, Yoneyama K, Xie X N, Ohnishi T, Seto Y, Yamaguchi S, Akiyama K, Yoneyama K, Nomura T. Carlactone is converted to carlactonoic acid by MAX1 in Arabidopsis and its methyl ester can directly interact with AtD14 in vitro. Proc Natl Acad Sci USA, 2014, 111: 18084-18089.
doi: 10.1073/pnas.1410801111 |
| [18] |
Hamiaux C, Drummond R S M, Janssen B J, Ledger S E, Cooney J M, Newcomb R D, Snowden K C. DAD2 is an alpha/beta hydrolase likely to be involved in the perception of the plant branching hormone, strigolactone. Curr Biol, 2012, 22: 2032-2036.
doi: 10.1016/j.cub.2012.08.007 pmid: 22959345 |
| [19] |
Germain A, Clavé G, Badet-Denisot M A, Pillot J P, Cornu D, Le Caer J P, Burger M, Pelissier Frank, Retailleau P, Turnbull C, Bonhomme S, Chory J, Rameau C, Boyer F D. An histidine covalent receptor and butenolide complex mediates strigolactone perception. Nat Chem Biol, 2016, 12: 787-794.
doi: 10.1038/nchembio.2147 |
| [20] | 田彦挺. 杨树独脚金内酯信号转导关键基因D14的克隆及功能研究. 山东农业大学硕士学位论文, 山东泰安, 2018. |
| Tian Y T. Cloning and Functional Study of D14, a Key Gene for Signal Transduction of Poplar Strigolactone. MS Thesis of Shandong Agricultural University, Tai’an, Shandong, China, 2018. (in Chinese with English abstract) | |
| [21] | 李炎坤, 卓一南, 曾湘达, 何瑞. 青天葵独脚金内酯信号转导关键基因D14的克隆与亚细胞定位分析. 热带作物学报, 2019, 40: 504-513. |
| Li Y K, Zhuo Y N, Zeng X D, He R.Cloning and expression analysis of D14, the key gene in the signal transduction of strigolactones from Nervilia fordii. Chin J Trop Crops, 2019, 40: 504-513. (in Chinese with English abstract) | |
| [22] | 谢兆辉. 基因概念的演绎. 遗传, 2010, 32: 448-454. |
| Xie Z H. The development of gene concepts. Hereditas, 2010, 32: 448-454. | |
| [23] | 张志鹏, 王晓玥, 黄少雄, 张昭. 植物功能基因单核苷酸多态性的研究进展. 中国农学通报, 2016, 32(20): 25-29. |
| Zhang Z P, Wang X Y, Huang S X, Zhang Z. Research progress of single nucleotide polymorphism in plant functional genes. Chin Agric Sci Bull, 2016, 32(20): 25-29. (in Chinese with English abstract) | |
| [24] |
Zhang J S, Nagai C, Yu Q Y, Pan Y B, Ayala-Silva T, Schnell R J, ComstocK J C, Arumuganathan A K, Ming R. Genome size variation in three Saccharum species. Euphytica, 2012, 185: 511-519.
doi: 10.1007/s10681-012-0664-6 |
| [25] |
Bundock P C, Eliott F G, Ablett G, Benson A D, Casu R E, Aitken K S, Henry R J. Targeted single nucleotide polymorphism (SNP) discovery in a highly polyploid plant species using 454 sequencing. Plant Biotechnol J, 2009, 7: 347-354.
doi: 10.1111/j.1467-7652.2009.00401.x pmid: 19386042 |
| [26] |
McIntyre C L, Jackson M, Cordeiro G M, Amouyal O, Hermann S, Aitken K S, Eliott F, Henry R J, Casu R E, Bonnett G D. The identification and characterisation of alleles of sucrose phosphate synthase gene family III in sugarcane. Mol Breed, 2006, 18: 39-50.
doi: 10.1007/s11032-006-9012-7 |
| [27] | 龚莺, 陈虹君, 许在恩, 郭小勤. 竹类植物Dwarf14 (D14)基因的多态性分析. 核农学报, 2018, 32: 48-57. |
| Gong Y, Chen H J, Xu Z E, Guo X Q.Polymorphisms of Dwarf14 (D14) gene in Bambusoideae. J Nuclear Agric Sci, 2018, 32: 48-57. (in Chinese with English abstract) |
| [1] | 崔致远, 秦晨展, 刘星雨, 张海, 曾康, 黄国强, 徐景升. 甘蔗类四跨膜蛋白ScTSPAN18与6K2互作应答SCMV侵染研究[J]. 作物学报, 2026, 52(6): 1618-1630. |
| [2] | 田春艳, 陆鑫, 吴才文, 徐超华, 刘家勇, 边芯, 桃联安. 基于荧光SSR的甘蔗创新种质遗传多样性分析及育种潜力评估[J]. 作物学报, 2026, 52(4): 1057-1072. |
| [3] | 杨宗桃, 杨婷, 王禹童, 艾静, 李燕烨, 刘家勇, 邓军, 赵勇, 张跃彬. 甘蔗CLC基因家族鉴定与表达分析[J]. 作物学报, 2026, 52(3): 722-734. |
| [4] | 詹戈锐, 余文, 李锋, 武明珠, 徐馨, 罗朝鹏, 巫升鑫, 杨军, 张智强, 王中. 烟草NtWRKY6基因响应ABA表达及其调控多酚合成的功能研究[J]. 作物学报, 2026, 52(2): 446-458. |
| [5] | 景秀清, 蔡永朵, 邓宁, 赵晓东, 翟飞红, 曾群. 藜麦RopGEF家族基因的鉴定及表达模式分析[J]. 作物学报, 2026, 52(1): 28-43. |
| [6] | 万慧兰, 吴华英, 曾丹, 钱禛锋, 赵昌祖, 廖然超, 何丽莲, 李富生. 蔗茅耐寒相关基因EfWRKY51克隆分析及功能验证[J]. 作物学报, 2025, 51(8): 2048-2059. |
| [7] | 张恒, 冯雅岚, 田文仲, 郭彬彬, 张均, 马超. 小麦TaSnRK基因家族鉴定及在局部根区干旱下的表达分析[J]. 作物学报, 2025, 51(3): 632-649. |
| [8] | 匡博文, 韦妳, 刘金典, 陈美燕, 毛兴洁, 段维兴, 杨细平. 基于甘蔗及其近缘属参考基因组开发SSR标记及数据库[J]. 作物学报, 2025, 51(1): 103-116. |
| [9] | 肖明昆, 严炜, 宋记明, 张林辉, 刘倩, 段春芳, 李月仙, 姜太玲, 沈绍斌, 周迎春, 沈正松, 熊贤坤, 罗鑫, 白丽娜, 刘光华. 卷叶木薯及其突变体叶片的比较转录组分析[J]. 作物学报, 2024, 50(8): 2143-2156. |
| [10] | 高维东, 胡城祯, 张龙, 张艳艳, 张沛沛, 杨德龙, 陈涛. 小麦泛素结合酶TaUBC16基因的克隆与功能分析[J]. 作物学报, 2024, 50(8): 1971-1988. |
| [11] | 李旭娟, 李纯佳, 田春艳, 孔春艳, 徐超华, 刘新龙. 甘蔗硝酸盐转运蛋白1/肽转运蛋白家族6.4基因(ScNPF6.4)克隆及其调控分蘖功能分析[J]. 作物学报, 2024, 50(8): 2131-2142. |
| [12] | 玉泉馨, 杨宗桃, 张海, 程光远, 焦文迪, 曾康, 罗廷绪, 黄国强, 王璐, 徐景升. 甘蔗类钙调素ScCML13与SCMV运动蛋白P3N-PIPO的互作研究[J]. 作物学报, 2024, 50(7): 1855-1866. |
| [13] | 王亚琪, 徐海风, 李曙光, 傅蒙蒙, 余希文, 赵志鑫, 杨加银, 赵团结. 大豆类病变皱叶突变体NT301遗传分析和2对基因定位[J]. 作物学报, 2024, 50(4): 808-819. |
| [14] | 琚吉浩, 马超, 王添宁, 吴毅, 董钟, 方美娥, 陈钰姝, 张均, 付国占. 小麦TaPOD家族的全基因组鉴定及表达分析[J]. 作物学报, 2024, 50(3): 779-792. |
| [15] | 薛丽, 李心怡, 黄勇泰, 欧财篮, 吴小青, 余泽怀, 崔泽田, 张木清, 邓祖湖, 余凡. 甘蔗与斑茅杂交染色体组构成特征研究[J]. 作物学报, 2024, 50(3): 633-644. |
|
||