欢迎访问作物学报,今天是

作物学报 ›› 2019, Vol. 45 ›› Issue (10): 1604-1612.doi: 10.3724/SP.J.1006.2019.81091

• 研究简报 • 上一篇    

基于高通量GBS-SNP标记的栽培燕麦六倍体起源研究

周萍萍1,2,颜红海1,2,3,*(),彭远英2,*()   

  1. 1西华师范大学生命科学学院, 四川南充 637009
    2四川农业大学小麦研究所, 四川成都 611130
    3西华师范大学组织修复材料工程技术中心, 四川南充 637009
  • 收稿日期:2018-12-24 接受日期:2019-05-12 出版日期:2019-10-12 网络出版日期:2019-09-10
  • 通讯作者: 颜红海,彭远英
  • 基金资助:
    本研究由国家自然科学基金项目(31571739);西华师范大学博士科研启动基金项目资助(17E081)

Hexaploid ancestor of cultivated hexaploid oats inferred from high throughput GBS-SNP markers

ZHOU Ping-Ping1,2,YAN Hong-Hai1,2,3,*(),PENG Yuan-Ying2,*()   

  1. 1College of Life Sciences, China West Normal University, Nanchong 637009, Sichuan, China
    2Triticeae Research Institute, Sichuan Agricultural University, Chengdu 611130, Sichuan, China
    3Collaboration and Innovation Center of Tissue Repair Material Engineering Technology, China West Normal University, Nanchong 637009, Sichuan, China
  • Received:2018-12-24 Accepted:2019-05-12 Published:2019-10-12 Published online:2019-09-10
  • Contact: Hong-Hai YAN,Yuan-Ying PENG
  • Supported by:
    This study was supported by the National Natural Science Foundation of China(31571739);the Doctoral Scientific Research Foundation of West China Normal University(17E081)

摘要:

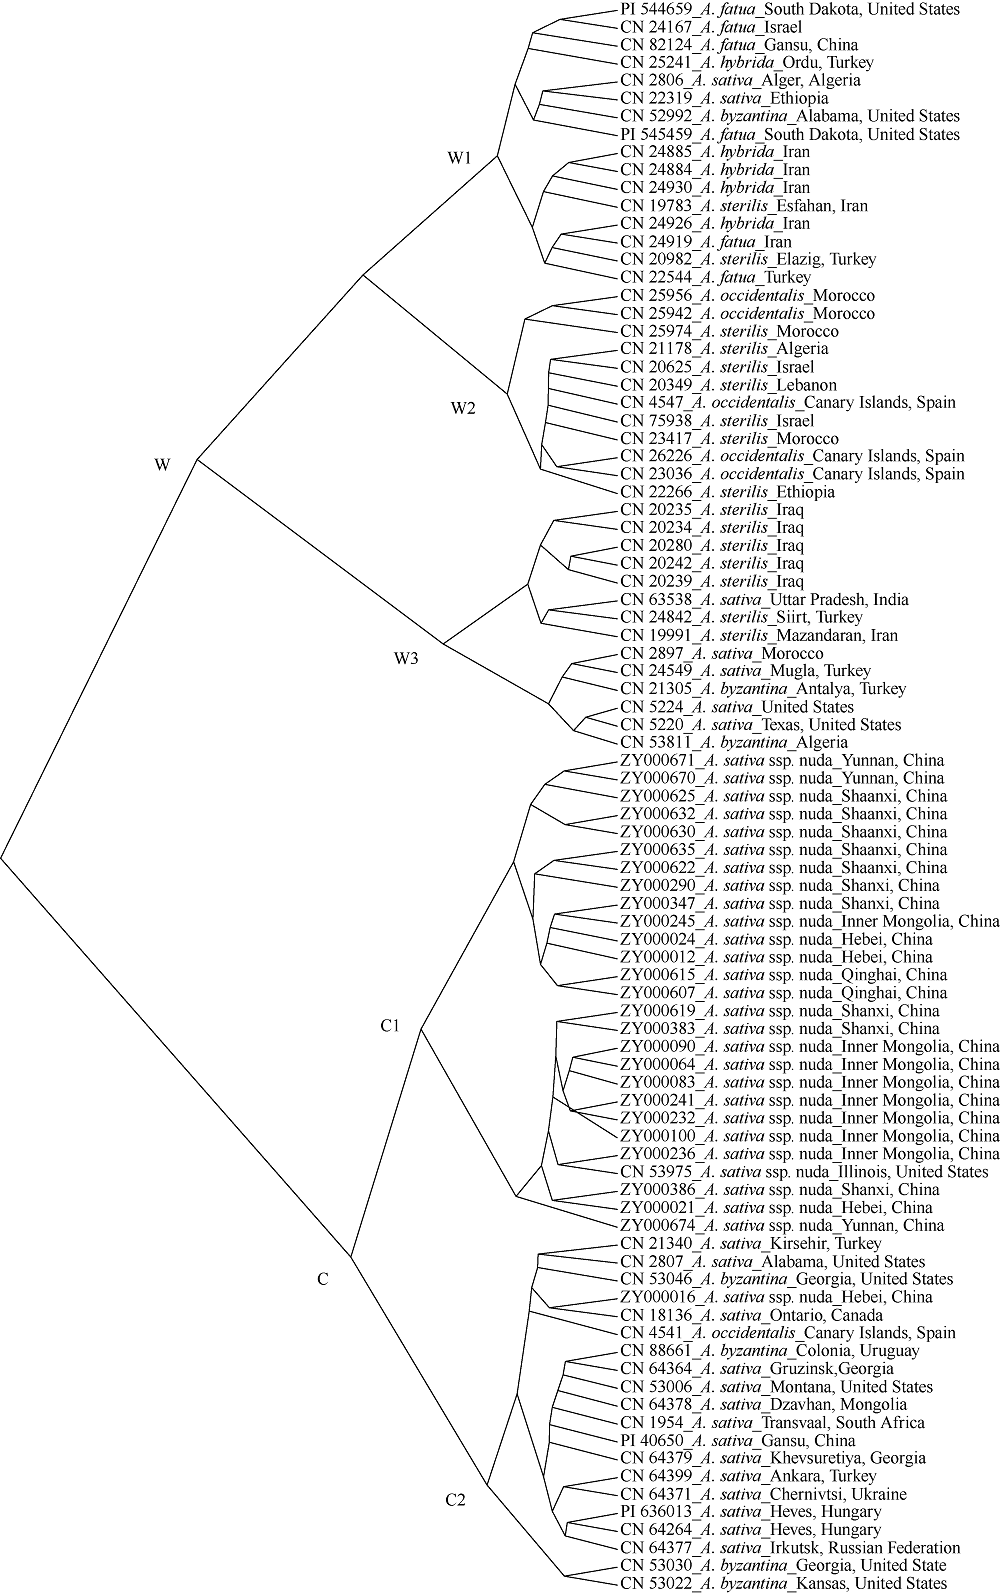
栽培六倍体燕麦是世界重要粮食作物, 理清其起源对燕麦种质资源的高效利用和保护具有重要意义。本研究利用GBS (genotyping by sequencing)对27份来自中国的大粒裸燕麦材料测序, 结合先前发表的包括6个六倍体燕麦种在内的66份燕麦材料的GBS数据进行SNP挖掘。UNEAK管道挖掘共计得到MAF大于0.5, call rate大于0.95的SNP标记8902个。进一步剔除缺失值大于0.15的4个燕麦材料后, 对其余89份材料进行PCA分析、STRUCTURE分析以及UPGMA聚类分析。结果表明, 在野生种中, 除A. sterilis外, 大多数来自同一物种的材料聚为一类, 不同物种间能够较好地分开, 表明这些物种之间存在较强的遗传分化。聚类分析将供试材料分为分别代表野生种和栽培种的2支, 表明野生种和栽培种之间存在明显的遗传差异; 在栽培种中, A. sativaA. byzantina具有较高的遗传多样性, 分散在不同的类群中, 二者未出现明显的遗传分化, 具有较高的遗传同质性, A. sativa ssp. nuda与A. sativa亲缘关系较近, 但存在一定的遗传分化, 因此形成独立的类群。值得注意的是, 来自野生种A. sterilis的材料被分在2个类群中, 其中来自西南亚地区(伊朗-伊拉克-土耳其地区)的居群与A. sativaA. byzantina聚在一起, 揭示此地区的A. sterilis居群可能是A. sativaA. byzantina的祖先种。野生种A. hybrida显示出与A. fatua较高的遗传同质性, 因此将其作为A. fatua的亚种较为合理。本研究为栽培六倍体燕麦起源提供了理论依据。

关键词: 栽培六倍体燕麦, GBS测序, 驯化, 起源, SNP标记

Abstract:

Cultivated hexaploid oat is one of the most important cereal crops in the word, clearing its hexaploid ancestor would substantially improve the utilization efficiency of the genetic resources of oat, and therefore provide theoretical reference for oat germplasm conservation. In this study, 27 naked oats originated from China were sequenced by using GBS (genotyping by sequencing). SNPs were calling by combining the previously published GBS data of another 66 hexaploid oats including six species using UNEAK pipeline. A total of 8902 SNPs with MAF > 0.5, call rate > 0.95 were obtained. Four taxa with missing value greater than 15% were excluded for further analyses. Finally, 89 oat taxa meeting the requirement were used for PCA, STRUCTURE and UPGMA clustering analyses. All three analyses revealed some consistent results as follows: most wild hexaploid oats with the exception of A. sterilis showed strong genetic differentiations among each other, resulting in a grouping by species. Clustering analysis divided all the taxa into two clusters representing wild species and cultivated species, respectively, indicating some significant genetic differences existed between this two types of hexaploids. Within cultivated hexaploid oats, A. byzantina showed a high degree of genetic homogeneity with A. sativa, while naked oats differed from the others and formed an independent subcluster with close relationships with A. sativa. The taxa from the wild hexaploid species A. sterilis were mainly subdivided into two groups. Notably, these accessions of A. sterilis originated from western Asia (Iran-lraq-Turkey region) were clustered with the cultivated oats A. sativa and A. byzantina, suggesting that A. sativa and A. byzantina might be derived from progenitor germplasm from Iran-lraq-Turkey region. Another wild hexaploid species A. hybrida showed high degree of genetic homogeneity with A. fatua, is better to consider as a subspecies of A. fatua. This research contributes to clarifying the hexaploid origin of cultivated hexaploid oats.

Key words: cultivated hexaploid oat, GBS, domestication, origin, SNPs

表1

六倍体燕麦种质材料的种名、材料编号、来源地及种质类型"

种名a
Speciesa
材料编号b
Accession numberb
来源地
Origin
种质类型
Germplasm type
A. byzantina CN 21305 Antalya, Turkey Cultivated material
A. byzantina CN 52992 Alabama, United States Cultivar
A. byzantina CN 53022 Kansas, United States Cultivar
A. byzantina CN 53030 Georgia, United State Cultivar
A. byzantina CN 53046 Georgia, United States Cultivar
A. byzantina CN 53811 Algeria Cultivated material
A. byzantina CN 88661 Colonia, Uruguay Cultivar
A. fatua CN 21269 Iraq Wild species
A. fatua CN 22544 Turkey Wild species
A. fatua CN 24167 Israel Wild species
A. fatua CN 24919 Iran Wild species
A. fatua CN 82124 Gansu, China Wild species
A. fatua PI 545459 South Dakota United States Wild species
A. fatua PI 560776 Van Turkey Wild species
A. fatua PI 544659 South Dakota, United States Wild species
A. hybrida CN 24884 Iran Wild species
A. hybrida CN 24885 Iran Wild species
A. hybrida CN 24926 Iran Wild species
A. hybrida CN 24930 Iran Wild species
A. hybrida CN 25241 Ordu, Turkey Wild species
A. occidentalis CN 23036 Canary Islands, Spain Wild species
A. occidentalis CN 25942 Morocco Wild species
A. occidentalis CN 4541 Canary Islands, Spain Wild species
A. occidentalis CN 4547 Canary Islands, Spain Wild species
A. occidentalis CN 25956 Morocco Wild species
A. occidentalis CN 26226 Canary Islands, Spain Wild species
A. sativa CN 18136 Ontario, Canada Cultivar
A. sativa CN 1954 Transvaal, South Africa Cultivated material
A. sativa CN 22319 Ethiopia Cultivated material
A. sativa CN 24549 Mugla, Turkey Cultivated material
A. sativa CN 2806 Alger, Algeria Cultivar
A. sativa CN 2807 Alabama, United States Cultivar
A. sativa CN 2897 Morocco Cultivated material
A. sativa CN 5220 Texas, United States Cultivar
A. sativa CN 5224 United States Cultivar
A. sativa CN 53006 Montana, United States Cultivar
A. sativa CN 64264 Heves, Hungary Cultivated material
A. sativa CN 21340 Kirsehir, Turkey Cultivated material
A. sativa CN 63538 Uttar Pradesh, India Landrace
A. sativa CN 64364 Gruzinsk, Georgia Landrace
A. sativa CN 64371 Chernivtsi, Ukraine Landrace
A. sativa CN 64377 Irkutsk, Russian Federation Cultivated material
A. sativa CN 64378 Dzavhan, Mongolia Cultivated material
A. sativa CN 64379 Khevsuretiya, Georgia Landrace
A. sativa CN 64399 Ankara, Turkey Landrace
A. sativa PI 40650 Gansu, China Landrace
A. sativa PI 636013 Heves, Hungary Landrace
A. sativa CN 63917 Gonder, Ethiopia Landrace
A. sativa ssp. nuda CN 53975 Illinois, United States Cultivar
种名a
Speciesa
材料编号b
Accession numberb
来源地
Origin
种质类型
Germplasm type
A. sativa ssp. nuda ZY000674 Deqing, Yunnan, China Landrace
A. sativa ssp. nuda ZY000670 Lijiang, Yunnan, China Landrace
A. sativa ssp. nuda ZY000671 Lijiang, Yunnan, China Landrace
A. sativa ssp. nuda ZY000386 Fanshi, Shanxi, China Landrace
A. sativa ssp. nuda ZY000347 Lanxian, Shanxi, China Landrace
A. sativa ssp. nuda ZY000619 Huangzhong, Shanxi, China Landrace
A. sativa ssp. nuda ZY000383 Shenchi, Shanxi, China Landrace
A. sativa ssp. nuda ZY000290 Youyu, Shanxi, China Landrace
A. sativa ssp. nuda ZY000615 Minhe, Qinghai, China Landrace
A. sativa ssp. nuda ZY000607 Xining, Qinghai, China Landrace
A. sativa ssp. nuda ZY000012 Fengning, Hebei, China Landrace
A. sativa ssp. nuda ZY000021 Kangbao, Hebei, China Landrace
A. sativa ssp. nuda ZY000016 Zhuolu, Hebei, China Landrace
A. sativa ssp. nuda ZY000024 Shangyi, Hebei, China Landrace
A. sativa ssp. nuda ZY000232 Ningcheng, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000100 Huhhot, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000064 Jining, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000236 Keqi, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000083 Fengzhen, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000090 Zhuozi, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000241 Zuoqi, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000245 Shangdu, Inner Mongolia, China Landrace
A. sativa ssp. nuda ZY000632 Pingli, Shaanxi, China Landrace
A. sativa ssp. nuda ZY000625 Xunyang, Shaanxi, China Landrace
A. sativa ssp. nuda ZY000635 Ningshan, Shaanxi, China Landrace
A. sativa ssp. nuda ZY000622 Zhenping, Shaanxi, China Landrace
A. sativa ssp. nuda ZY000630 Zhenping, Shaanxi, China Landrace
A. sterilis CN 19783 Esfahan, Iran Wild species
A. sterilis CN 19991 Mazandaran, Iran Wild species
A. sterilis CN 20234 Iraq Wild species
A. sterilis CN 20235 Iraq Wild species
A. sterilis CN 20239 Iraq Wild species
A. sterilis CN 20242 Iraq Wild species
A. sterilis CN 20280 Iraq Wild species
A. sterilis CN 20349 Lebanon Wild species
A. sterilis CN 20625 Israel Wild species
A. sterilis CN 20982 Elazig, Turkey Wild species
A. sterilis CN 23417 Morocco Wild species
A. sterilis CN 24168 Israel Wild species
A. sterilis CN 24842 Siirt, Turkey Wild species
A. sterilis CN 25974 Morocco Wild species
A. sterilis CN 21178 Algeria Wild species
A. sterilis CN 22266 Ethiopia Wild species
A. sterilis CN 75938 Israel Wild species

图1

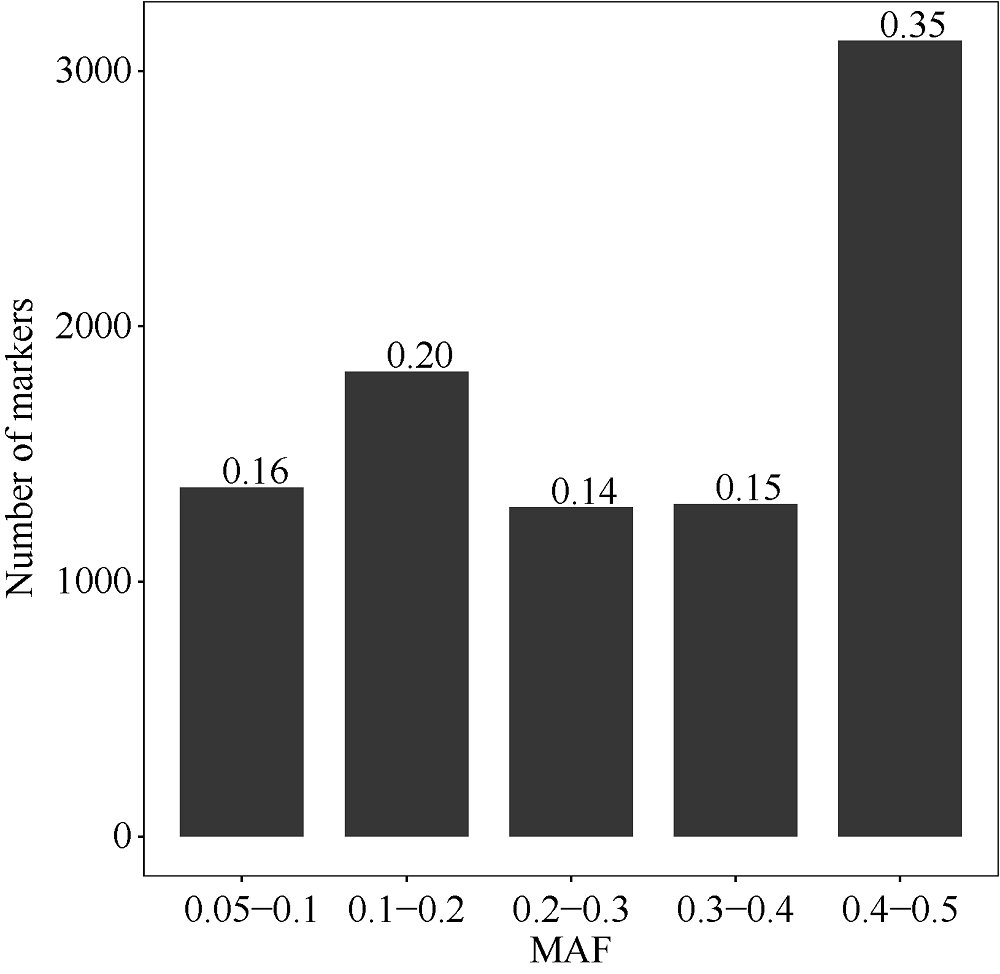
获得的GBS-SNP标记在不同MAF区间的分布 柱状图上面的数字表示占所获的GBS标记的百分比。"

图2

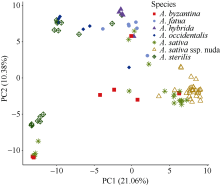
基于8902个GBS标记的89份燕麦材料的PCA分析"

图3

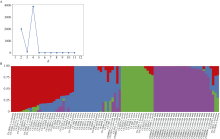
基于8902个GBS标记的STRUCTURE分析 A: Delta K在K=4时达到最大值。B: 最佳K(4)时分组情况。每种颜色代表一个类群(K=4), 每条竖线代表一个燕麦材料。"

图4

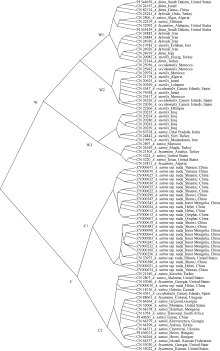
基于UPGMA方法的系统发育树"

[1] Kong L, Huo H, Mao P . Antioxidant response and related gene expression in aged oat seed. Front Plant Sci, 2015,6:158
[2] FAOSTATS. . 2016
[3] Coffman F A . Oat History, Identification and Classification. Washington D. C: US Department of Agriculture, Agricultural Research Service. 1977. pp 3-30
[4] Cox D J, Frey K J . Improving cultivated oats ( Avena sativa L.) with alleles for vegetative growth index from A. sterilis L. Theor Appl Genet, 1984,68:239-245
[5] Branson C V, Frey K J . Recurrent selection for groat oil content in oat. Crop Sci, 1989,29:1382-1387
[6] Zamir D . Improving plant breeding with exotic genetic libraries. Nat Rev Genet, 2001,2:983-989
[7] Loskutov I G, Rines H W. Avena. In: Kole C, ed. Wild Crop Relatives: Genomic and Breeding Resources. Heidelberg: Springer Press, 2011. pp 109-183
[8] Baum B R. Oats: Wild and Cultivated. A Monograph of the Genus Avena L. (Poaceae). Ottawa: Minister of Supply and Services Press, 1977.
[9] Ladizinsky G. Studies in Oat Evolution. A Man’s Life with Avena (Springer Briefs in Agriculture). Heidelberg: Springer Press, 2012. pp 1-18
[10] Coffman F A . Origin of cultivated oats. J Am Soc Agron, 1946,38:983-1002
[11] 郑殿升, 张宗文 . 大粒裸燕麦(莜麦)(Avena nuda L.)起源及分类问题的探讨. 植物遗传资源学报, 2011,5:667-670.
Zheng D S, Zhang Z W . Discussion on the origin and taxonomy of naked oat ( Avena nuda L.). J Plant Genet Resour, 2011,5:667-670 (in Chinese with English abstract)
[12] Zhou X, Jellen E N, Murphy J P . Progenitor germplasm of domisticated hexaploid oat. Crop Sci, 1999,39:1208-1214
[13] Loskutov I G . On evolutionary pathways of Avena species. Genet Resour Crop Evol, 2008,55:211-220
[14] 刘青, 刘欢, 林磊 . 燕麦属系统学研究进展. 热带亚热带植物学报, 2014,5:516-524
Liu Q, Liu H, Lin L . Research advances on systematics of Avena( Pooideae, Poaceae). J Trop Subtrop Bot, 2014,5:516-524 (in Chinese with English abstract)
[15] Ladizinsky G. The domestication and history of oats. In: Mattsson B, Lyhagen R, eds. Proceedings of the 3rd International Oat Conference, Lund, Sweden. Svalof AB, 1988. pp 7-12
[16] Baum B R . Extrapolation of the predomesticated hexaploid cultivated oats. Evolution, 1973,27:518-523
[17] Huang Y F, Poland J A, Wight C P, Tinker N A . Using genotyping-by-sequencing (GBS) for genomic discovery in cultivated oat. PLoS One, 2014,9:e102448
[18] Chew P, Meade K, Hayes A, Harjes C, Bao Y, Beattie A D, Puddephat I, Gusmini G, Tanksley S D . A study on the genetic relationships of Avena taxa and the origins of hexaploid oat. Theor Appl Genet, 2016,129:1405-1415
[19] Yan H, Bekele W A, Wight C P, Peng Y, Langdon T, Latta R G, Fu Y B, Diederichsen A, Howarth C J, Jellen E N, Boyle B, Wei Y, Tinker N A . High-density marker profiling confirms ancestral genomes of Avena species and identifies D-genome chromosomes of hexaploid oat. Theor Appl Genet, 2016,129:2133-2149
[20] Chaffin A S, Huang Y F, Smith S, Bekele W A, Babiker E, Gnanesh B N, Foresman B J, Blanchard S G, Jay J J, Reid R W, Wight C P, Chao S, Islamovic E, Kolb F L, McCartney C, Mitchell F J W, Beattie A D, Bjornstad A, Bonman J M, Langdon T, Howarth C J, Brouwer C R, Jellen E N, Klos K E, Poland J A, Hsieh T F, Brown R, Jackson E, Schlueter J A, Tinker N A . A consensus map in cultivated hexaploid oat reveals conserved grass synteny with substantial subgenome rearrangement. Plant Genome, 2016,9. doi: 10.3835/plantgenome2015.10.0102.
[21] Torkamaneh D, Laroche J, Belzile F . Genome-wide SNP calling from genotyping by sequencing (GBS) data: a comparison of seven pipelines and two sequencing technologies. PLoS One, 2016,11:e0161333
[22] Lu F, Lipka A E, Glaubitz J, Elshire R, Cherney J H, Casler M D, Buckler E S, Costich D E . Switchgrass genomic diversity, ploidy, and evolution: novel insights from a Nnetwork-based SNP discovery protocol. PLoS Genet, 2013,9:139-147
[23] Bradbury P J, Zhang Z, Kroon D E, Casstevens T M, Ramdoss Y, Buckler E S . TASSEL: software for association mapping of complex traits in diverse samples. Bioinformatics, 2007,23:2633-2635
[24] Pritchard J, Stephens M, Donnelly . Inference of population structure using multilocus genotype data. Genetics, 2000,155:945-959
[25] Evanno G, Regnaut S, Goudet J . Detecting the number of clusters of individuals using the software STRUCTURE: a simulation study. Mol Ecol, 2005,14:2611-2620
[26] Earl D A, Vonholdt B M . STRUCTURE HARVESTER: a website and program for visualizing STRUCTURE output and implementing the Evanno method. Conserv Genet Resour, 2012,4:359-361
[27] R Core Team. R: a language and environment for statistical computing. R Foundation for Statistical Computing, Vienna, Austria. . 2016.
[28] Souza E, Sorrells M E . Relationships among 70 north American oat germplasms: I. cluster analysis using quantitative characters. Crop Sci, 1991,31:599-605
[29] Koch. K . Beiträge zu einer flora des orients. Linnaeus, 1948,21:289-443
[30] Baohong G, Zhou X, Murphy J P . Genetic variation within Chinese and Western cultivated oat accessions. Cereal Res Commun, 2003,31:339-346
[31] Malzew A . Wild and cultivated oats: Sectio Eu Avena Griseb. Bull Appl Bot, Genet Plant Breed, 1930,38:473-506 (in Russian with English abstract)
[1] 郭向阳, 涂亮, 王栋, 刘鹏飞, 王安贵, 易强, 任洪, 李刚, 祝云芳, 吴迅, 蒋喻林, 田丰, 陈泽辉. 热带Suwan种质在我国玉米种质改良中的创新与利用[J]. 作物学报, 2026, 52(3): 655-664.
[2] 王琼, 邹丹霞, 陈兴运, 张威, 张红梅, 刘晓庆, 贾倩茹, 魏利斌, 崔晓艳, 陈新, 王学军, 陈华涛. 大豆开花时间和成熟期性状全基因组关联分析与候选基因预测[J]. 作物学报, 2025, 51(6): 1558-1568.
[3] 王亚雯, 戚正阳, 尤佳琦, 聂新辉, 曹娟, 杨细燕, 涂礼莉, 张献龙, 王茂军. 棉花60K功能位点基因芯片的制备及应用[J]. 作物学报, 2025, 51(5): 1178-1188.
[4] 许乃银, 金石桥, 晋芳, 刘丽华, 徐剑文, 刘丰泽, 任雪贞, 孙全, 许栩, 庞斌双. 基于SNP标记的小麦品种遗传相似度及其检测准确度分析[J]. 作物学报, 2024, 50(4): 887-896.
[5] 王琼, 朱宇翔, 周密密, 张威, 张红梅, 陈新, 陈华涛, 崔晓艳. 大豆叶型性状全基因组关联分析与候选基因鉴定[J]. 作物学报, 2024, 50(3): 623-632.
[6] 鲁宗辉, 司二静, 叶霈颖, 汪军成, 姚立蓉, 马小乐, 李葆春, 王化俊, 尚勋武, 孟亚雄. 大麦籽粒β-葡聚糖含量的全基因组关联分析及候选基因预测[J]. 作物学报, 2024, 50(10): 2483-2492.
[7] 杨斌, 乔玲, 赵佳佳, 武棒棒, 温宏伟, 张树伟, 郑兴卫, 郑军. 小麦旗叶叶绿素含量的QTL定位及验证[J]. 作物学报, 2023, 49(3): 744-754.
[8] 温明星, 肖进, 徐涛, 孙丽, 王宗宽, 王海燕, 王秀娥. 利用55K芯片进行小麦生育期相关性状的QTL定位及效应分析[J]. 作物学报, 2023, 49(12): 3188-3203.
[9] 刘丹, 周彩娥, 王晓婷, 吴启蒙, 张旭, 王琪琳, 曾庆东, 康振生, 韩德俊, 吴建辉. 利用集群分离分析结合高密度芯片快速定位小麦成株期抗条锈病基因YrC271[J]. 作物学报, 2022, 48(3): 553-564.
[10] 郑向华, 叶俊华, 程朝平, 魏兴华, 叶新福, 杨窑龙. 利用SNP标记进行水稻品种籼粳鉴定[J]. 作物学报, 2022, 48(2): 342-352.
[11] 张潇文, 李世姣, 张晓军, 李欣, 杨足君, 张树伟, 陈芳, 常利芳, 郭慧娟, 畅志坚, 乔麟轶. 小麦品系CH7034中耐盐QTL定位[J]. 作物学报, 2022, 48(10): 2654-2662.
[12] 张春, 赵小珍, 庞承珂, 彭门路, 王晓东, 陈锋, 张维, 陈松, 彭琦, 易斌, 孙程明, 张洁夫, 傅廷栋. 甘蓝型油菜千粒重全基因组关联分析[J]. 作物学报, 2021, 47(4): 650-659.
[13] 孙程明,陈锋,陈松,彭琦,张维,易斌,张洁夫,傅廷栋. 甘蓝型油菜每角粒数的全基因组关联分析[J]. 作物学报, 2020, 46(01): 147-153.
[14] 孙程明,陈松,彭琦,张维,易斌,张洁夫,傅廷栋. 甘蓝型油菜角果长度性状的全基因组关联分析[J]. 作物学报, 2019, 45(9): 1303-1310.
[15] 杨芳萍,刘金栋,郭莹,贾奥琳,闻伟鄂,巢凯翔,伍玲,岳维云,董亚超,夏先春. 普通小麦‘Holdfast’条锈病成株抗性QTL定位[J]. 作物学报, 2019, 45(12): 1832-1840.
Viewed
Full text


Abstract

Cited

  Shared   
  Discussed   
No Suggested Reading articles found!