欢迎访问作物学报,今天是
作物学报 ›› 2022, Vol. 48 ›› Issue (7): 1645-1657.doi: 10.3724/SP.J.1006.2022.14107
韩尚玲1( ), 霍轶琼1,2, 李辉1, 韩华蕊1, 侯思宇1,2,3, 孙朝霞1,2,3, 韩渊怀1,2,3, 李红英1,2,3,*()
HAN Shang-Ling1(), HUO Yi-Qiong1,2, LI Hui1, HAN Hua-Rui1, HOU Si-Yu1,2,3, SUN Zhao-Xia1,2,3, HAN Yuan-Huai1,2,3, LI Hong-Ying1,2,3,*()
摘要:
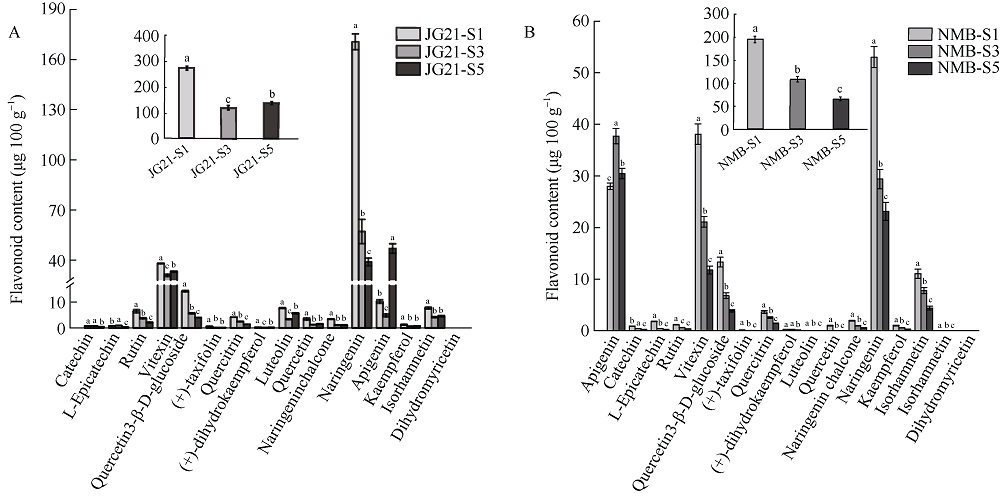
类黄酮是植物重要的次生代谢物质, 在植物生长发育中发挥着重要的作用, 此外, 类黄酮具有抗氧化活性, 对人体十分有益。谷子籽粒营养丰富全面, 是一种保健型杂粮, 深受我国人民喜爱。谷子作为C4模式植物, 正在受到越来越多的关注。目前谷子籽粒类黄酮代谢及调控机制研究较少。本研究利用高类黄酮品种晋谷21 (JG21)及低类黄酮品种牛毛白(NMB)谷穗为材料, 分析JG21与NMB小穗发育不同阶段类黄酮靶向代谢组及JG21小穗发育不同阶段转录组, 结合加权基因共表达网络分析挖掘可能参与调控类黄酮代谢的转录因子, 并在不同水平的类黄酮品种中进行表达分析初步验证。结果发现, 2个品种小穗中主要富集的类黄酮组分为芹菜素、牡荆素及柚皮素, 三者共占总类黄酮含量的79%以上。类黄酮代谢基因共表达网络中包含38,921个基因, 共划分为32个模块, 其中turquoise模块、green模块及magenta模块与类黄酮代谢显著相关。利用类黄酮代谢通路差异表达基因作为关键基因筛选出与类黄酮代谢调控相关的27个转录因子家族, 并通过启动子结合基序分析筛选获得11个转录因子。Pearson相关性分析表明, 11个转录因子中有7个候选转录因子可能参与类黄酮代谢, 分别为WRKY38、MYB4a、PI、WRKY15、WRKY62、MYB46、WRKY23。以上结果为研究谷子类黄酮代谢通路转录调控机制提供了新的候选基因, 为深入揭示类黄酮代谢调控机制奠定基础。
| [1] |
Williams C A, Grayer R J. Anthocyanins and other flavonoids. Nat Prod Rep, 2004, 21: 539-573.
doi: 10.1039/b311404j |
| [2] |
Buer C S, Imin N, Djordjevic M A. Flavonoids: new roles for old molecules. J Integr Plant Biol, 2010, 52: 98-111.
doi: 10.1111/j.1744-7909.2010.00905.x |
| [3] | Kozłowska A, Szostak-Wegierek D. Flavonoids-food sources and health benefits. Rocz Panstw Zakl Hig, 2014, 65: 79-85. |
| [4] |
Nakabayashi R, Yonekura-Sakakibara K, Urano K, Suzuki M, Yamada Y, Nishizawa T, Matsuda F, Kojima M, Sakakibara H, Shinozaki K, Michael A J, Tohge T, Yamazaki M, Saito K. Enhancement of oxidative and drought tolerance in Arabidopsis by overaccumulation of antioxidant flavonoids. Plant J, 2014, 77: 367-379.
doi: 10.1111/tpj.12388 |
| [5] |
Gouot J C, Smith J P, Holzapfel B P, Walker A R, Barril C. Grape berry flavonoids: a review of their biochemical responses to high and extreme high temperatures. J Exp Bot, 2019, 70: 397-423.
doi: 10.1093/jxb/ery392 |
| [6] | Pan J Q, Tong X R, Guo B L. Progress of effects of light on plant flavonoids. China J Chin Mater Med, 2016, 41: 3897-3903. |
| [7] |
Xu W J, Dubos C, Lepiniec L. Transcriptional control of flavonoid biosynthesis by MYB-bHLH-WDR complexes. Trends Plant Sci, 2015, 20: 176-185.
doi: 10.1016/j.tplants.2014.12.001 |
| [8] | 刁现民.谷子种质资源的深度分析和研究利用. 见: 2017年中国作物学会学术年会摘要集, 保定: 中国作物学会, 2017. p 1. |
| Diao X M. In-depth analysis and research utilization of foxtail millet germplasm resources. In: Abstract ppub of the Academic Annual Meeting of Chinese Crop Society in 2017Baoding: The Crop Science Society of China, 2017. p 1. (in Chinese) | |
| [9] | 徐玖亮, 温馨, 刁现民, 张福锁, 李学贤. 我国主要谷类杂粮的营养价值及保健功能. 粮食与饲料工业, 2021, (1): 27-35. |
| Xu J L, Wen X, Diao X M, Zhang F S, Li X X. Nutrition values and health effects of coarse cereals in China. Cereal Feed Ind, 2021, (1): 27-35. (in Chinese with English abstract) | |
| [10] |
Zhang Y K, Gao J H, Qie Q R, Yang Y L, Hou S Y, Wang X C, Li X K, Han Y H. Comparative analysis of flavonoid metabolites in foxtail millet (Setaria italica) with different eating quality. Life (Basel), 2021, 11: 578.
doi: 10.3390/life11060578 |
| [11] | 鲜小华, 王嘉, 徐新福, 曲存民, 卢坤, 李加纳, 刘列钊. 整合GWAS和WGCNA分析挖掘甘蓝型油菜黄籽微效作用位点. 作物学报, 2018, 44: 1105-1113. |
|
Xian X H, Wang J, Xu X F, Qu C M, Lu K, Li J N, Liu L Z. Mining yellow-seeded micro effect loci in B. napus by integrated GWAS and WGCNA analysis. Acta Agron Sin, 2018, 44: 1105-1113. (in Chinese with English abstract)
doi: 10.3724/SP.J.1006.2018.01105 |
|
| [12] | 程旭.基于转录组和共表达网络分析的玫瑰类黄酮和萜类生物合成相关基因研究. 华中农业大学硕士学位论文,湖北武汉, 2016. |
| Cheng X. Research of Flavonoids and Terpenoids Biosynthesis Genes Based on Transcriptome and Co-expression Network Analysis. MS Thesis of Huazhong Agricultural University, Wuhan, Hubei, China, 2016. (in Chinese with English abstract) | |
| [13] |
Yang Z R, Zhang H S, Li X K, Shen H M, Gao J H, Hou S Y, Zhang B, Mayes S, Bennett M, Ma J X, Wu C Y, Sui Y, Han Y H, Wang X C. A mini foxtail millet with an Arabidopsis-like life cycle as a C4 model system. Nat Plants, 2020, 6: 1167-1178.
doi: 10.1038/s41477-020-0747-7 |
| [14] | Andrews S. Babraham bioinformatics-FastQC a quality control tool for high throughput sequence data. Bioinformatics, 2010, 26: 774-798. |
| [15] |
Bolger A M, Lohse M, Usadel B. Trimmomatic: a flexible trimmer for Illumina sequence data. Bioinformatics, 2014, 30: 2114-2120.
doi: 10.1093/bioinformatics/btu170 |
| [16] |
Kim D, Langmead B, Salzberg S L. HISAT: a fast spliced aligner with low memory requirements. Nat Methods, 2015, 12: 357-360.
doi: 10.1038/NMETH.3317 |
| [17] |
Pertea M, Pertea G M, Antonescu C M, Chang T C, Mendell J T, Salzberg S L. StringTie enables improved reconstruction of a transcriptome from RNA-seq reads. Nat Biotechnol, 2015, 33: 290-295.
doi: 10.1038/nbt.3122 |
| [18] |
Love M I, Huber W, Anders S. Moderated estimation of fold change and dispersion for RNA-seq data with DESeq2. Genome Biol, 2014, 15: 550.
doi: 10.1186/s13059-014-0550-8 |
| [19] | Fornes O, Castro-Mondragon J A, Khan A, van der Lee R, Zhang X, Richmond P A, Modi B P, Correard S, Gheorghe M, Baranašić D, Santana-Garcia W, Tan G, Chèneby J, Ballester B, Parcy F, Sandelin A, Lenhard B, Wasserman W W, Mathelier A. JASPAR 2020: update of the open-access database of transcription factor binding profiles. Nucleic Acids Res, 2020, 48: D87-D92. |
| [20] |
Monniaux M, McKim S M, Cartolano M, Thévenon E, Parcy F, Tsiantis M, Hay A. Conservation vs divergence in LEAFY and APETALA1 functions between Arabidopsis thaliana and Cardamine hirsuta. New Phytol, 2017, 216: 549-561.
doi: 10.1111/nph.14419 pmid: 28098947 |
| [21] |
Goslin K, Zheng B B, Serrano-Mislata A, Rae L, Ryan P T, Kwaśniewska K, Thomson B, Ó’Maoiléidigh D S, Madueño F, Wellmer F, Graciet E. Transcription factor interplay between LEAFY and APETALA1/CAULIFLOWER during floral initiation. Plant Physiol, 2017, 174: 1097-1109.
doi: 10.1104/pp.17.00098 pmid: 28385730 |
| [22] |
Han Y Y, Zhang C, Yang H B, Jiao Y L. Cytokinin pathway mediates APETALA1 function in the establishment of determinate floral meristems in Arabidopsis. Proc Natl Acad Sci USA, 2014, 111: 6840-6845.
doi: 10.1073/pnas.1318532111 |
| [23] |
Kim W C, Ko J H, Kim J Y, Kim J, Bae H J, Han K H. MYB 46directly regulates the gene expression of secondary wall- associated cellulose synthases in Arabidopsis. Plant J, 2013, 73: 26-36.
doi: 10.1111/j.1365-313x.2012.05124.x |
| [24] |
Kim W C, Kim J Y, Ko J H, Kim J, Han K H. Transcription factor MYB46 is an obligate component of the transcriptional regulatory complex for functional expression of secondary wall- associated cellulose synthases in Arabidopsis thaliana . J Plant Physiol, 2013, 170: 1374-1378.
doi: 10.1016/j.jplph.2013.04.012 |
| [25] |
Zhong R, Ye Z H. MYB46 and MYB83 bind to the SMRE sites and directly activate a suite of transcription factors and secondary wall biosynthetic genes. Plant Cell Physiol, 2012, 53: 368-380.
doi: 10.1093/pcp/pcr185 |
| [26] |
Wang X C, Wu J, Guan M L, Zhao C H, Geng P, Zhao Q. Arabidopsis MYB4 plays dual roles in flavonoid biosynthesis. Plant J, 2020, 101: 637-652.
doi: 10.1111/tpj.14570 |
| [27] |
Lazakis C M, Coneva V, Colasanti J. ZCN8 encodes a potential orthologue of Arabidopsis FT florigen that integrates both endogenous and photoperiod flowering signals in maize. J Exp Bot, 2011, 62: 4833-4842.
doi: 10.1093/jxb/err129 pmid: 21730358 |
| [28] |
Coneva V, Guevara D, Rothstein S J, Colasanti J. Transcript and metabolite signature of maize source leaves suggests a link between transitory starch to sucrose balance and the autonomous floral transition. J Exp Bot, 2012, 63: 5079-5092.
doi: 10.1093/jxb/ers158 |
| [29] |
Mara C D, Huang T, Irish V F. The Arabidopsis floral homeotic proteins APETALA3 and PISTILLATA negatively regulate the BANQUO genes implicated in light signaling. Plant Cell, 2010, 22: 690-702.
doi: 10.1105/tpc.109.065946 |
| [30] |
Kim K C, Lai Z, Fan B, Chen Z. Arabidopsis WRKY38 and WRKY62 transcription factors interact with histone deacetylase 19 in basal defense. Plant Cell, 2008, 20: 2357-2371.
doi: 10.1105/tpc.107.055566 |
| [31] |
Mao P, Duan M R, Wei C H, Li Y. WRKY62 transcription factor acts downstream of cytosolic NPR1 and negatively regulates jasmonate-responsive gene expression. Plant Cell Physiol, 2007, 48: 833-842.
doi: 10.1093/pcp/pcm058 |
| [32] |
Grunewald W, De Smet I, Lewis D R, Löfke C, Jansen L, Goeminne G, Vanden Bossche R, Karimi M, De Rybel B, Vanholme B, Teichmann T, Boerjan W, Van Montagu M C, Gheysen G, Muday G K, Friml J, Beeckman T. Transcription factor WRKY23 assists auxin distribution patterns during Arabidopsis root development through local control on flavonol biosynthesis. Proc Natl Acad Sci USA, 2012, 109: 1554-1559.
doi: 10.1073/pnas.1121134109 |
| [33] |
Prát T, Hajný J, Grunewald W, Vasileva M, Molnár G, Tejos R, Schmid M, Sauer M, Friml J. WRKY23 is a component of the transcriptional network mediating auxin feedback on PIN polarity. PLoS Genet, 2018, 14: e1007177.
doi: 10.1371/journal.pgen.1007177 |
| [34] |
Guo X Y, Wang Y, Zhao P X, Xu P, Yu G H, Zhang L Y, Xiong Y, Xiang C B. AtEDT1/HDG11 regulates stomatal density and water-use efficiency via ERECTA and E2Fa. New Phytol, 2019, 223: 1478-1488.
doi: 10.1111/nph.15861 |
| [35] |
Cai X T, Xu P, Wang Y, Xiang C B. Activated expression of AtEDT1/HDG11 promotes lateral root formation in Arabidopsis mutant edt1 by upregulating jasmonate biosynthesis. J Integr Plant Biol, 2015, 57: 1017-1730.
doi: 10.1111/jipb.12347 |
| [36] |
Yu L H, Wu S J, Peng Y S, Liu R N, Chen X, Zhao P, Xu P, Zhu J B, Jiao G L, Pei Y, Xiang C B. Arabidopsis EDT1/HDG11 improves drought and salt tolerance in cotton and poplar and increases cotton yield in the field. Plant Biotechnol J, 2016, 14: 72-84.
doi: 10.1111/pbi.12358 |
| [37] |
Vanderauwera S, Vandenbroucke K, Inzé A, van de Cotte B, Mühlenbock P, De Rycke R, Naouar N, Van Gaever T, Van Montagu M C, Van Breusegem F. AtWRKY 15perturbation abolishes the mitochondrial stress response that steers osmotic stress tolerance in Arabidopsis. Proc Natl Acad Sci USA, 2012, 109: 20113-20118.
doi: 10.1073/pnas.1217516109 |
| [38] |
Ge S T, Han X F, Xu X W, Shao Y M, Zhu Q K, Liu Y D, Du J, Xu J, Zhang S Q. WRKY15 suppresses tracheary element differentiation upstream of VND7 during xylem formation. Plant Cell, 2020, 32: 2307-2324.
doi: 10.1105/tpc.19.00689 |
| [39] |
Gu Z Y, Men S Q, Zhu J, Hao Q, Tong N N, Liu Z A, Zhang H C, Shu Q Y, Wang L S. Chalcone synthase is ubiquitinated and degraded via interactions with a RING-H2 protein in petals of Paeonia‘he xie’. J Exp Bot, 2019, 70: 4749-4762.
doi: 10.1093/jxb/erz245 |
| [40] | 张丽玲, 郄倩茹, 罗韶凡, 牛文康, 朱喆标, 高雨柔, 李旭凯, 韩渊怀. 谷子12种黄酮类代谢物合成通路分析. 山西农业大学学报(自然科学版), 2020, 40(4): 10-18. |
| Zhang L L, Qie Q R, Luo S F, Niu W K, Zhu Z B, Gao Y R, Li X K, Han Y H. Analysis of synthesis pathway of twelve flavonoid metabolites in foxtail millet. J Shanxi Agric Univ (Nat Sci Edn), 2020, 40(4): 10-18. (in Chinese with English abstract) | |
| [41] |
Gonzalez A, Zhao M Z, Leavitt J M, Lloyd A M. Regulation of the anthocyanin biosynthetic pathway by the TTG1/bHLH/Myb transcriptional complex in Arabidopsis seedlings. Plant J, 2008, 53: 814-827.
doi: 10.1111/j.1365-313X.2007.03373.x |
| [42] |
Mohamed H I, Latif H H. Improvement of drought tolerance of soybean plants by using methyl jasmonate. Physiol Mol Biol Plants, 2017, 23: 545-556.
doi: 10.1007/s12298-017-0451-x |
| [1] | 陈国欢, 张锐, 李艳迪, 赵佳琪, 任湧涛, 张天赐, 郭华春, 李俊, 杨芳. 外源硒叶面喷施对浅紫色马铃薯块茎花青素合成的影响[J]. 作物学报, 2026, 52(6): 1876-1890. |
| [2] | 马小倩, 秦娜, 代书桃, 秦家范, 李小艳, 王淑婷, 刘忠玲, 李君霞. 175份谷子种质在2种环境下的表型变异分析[J]. 作物学报, 2026, 52(6): 1757-1773. |
| [3] | 王文辕, 燕雪嘉, 刘玉霖, 孙晓彤, 李亚楠, 唐鑫华, 石瑛. 耐弱光马铃薯品种筛选及转录因子编码基因StPIF3的克隆与功能分析[J]. 作物学报, 2026, 52(6): 1631-1645. |
| [4] | 邹仪妹, 徐敏, 汪海洋, 姚辉, 王加峰, 刘浩, 任代胜. 两系不育系水稻幼苗根系响应盐胁迫的转录因子调控网络鉴定[J]. 作物学报, 2026, 52(6): 1728-1742. |
| [5] | 蔡兆琴, 何观咏, 何文, 阮丽霞, 梁振华, 李永珍, 李恒锐, 陈会鲜. 木薯分枝发育过程的动态转录组分析与关键基因发掘[J]. 作物学报, 2026, 52(5): 1430-1441. |
| [6] | 谷春苗, 王润风, 黄璐, 刘浩, 鲁清, 李海芬, 李少雄, 何双呈, 洪彦彬, 陈小平, 谭斌, 余倩霞. 花生WOX基因家族的全基因组分析及不定芽再生候选基因的鉴定[J]. 作物学报, 2026, 52(5): 1326-1340. |
| [7] | 王懿涵, 李富昌, 刘意, 朱国鹏. 甘薯IbOPR2基因启动子克隆及调控因子的筛选[J]. 作物学报, 2026, 52(4): 1268-1276. |
| [8] | 杨影, 郝豫皖, 张学宁, 方佳璐, 马月华, 杨伟龙, 孙文清, 王新超, 王玉春, 黄建燕. 乙烯响应因子CsERF9调控茶树炭疽病抗性的分子机制研究[J]. 作物学报, 2026, 52(4): 1103-1115. |
| [9] | 马娟娥, 姚有华, 姚晓华, 吴昆仑, 崔永梅. 青稞HvERF039基因的克隆及功能研究[J]. 作物学报, 2025, 51(9): 2341-2357. |
| [10] | 杨海洋, 吴林宣, 李博纹, 石翰峰, 袁禧龙, 刘金朝, 蔡海荣, 陈诗怡, 郭涛, 王慧. 基于QTL定位发现的OsWRI3调控水稻种子的落粒性[J]. 作物学报, 2025, 51(7): 1712-1724. |
| [11] | 王若楠, 张颖星, 于筱菡, 刘少雄, 王跃, 薛亚鹏, 辛旭霞, 张莉, 刘敏轩. 基于近红外快速检测技术的谷子淀粉多样性分析及模型构建[J]. 作物学报, 2025, 51(7): 1757-1768. |
| [12] | 沈傲, 刘敏, 倪迪安, 刘炜. 谷子m6A甲基转移酶基因SiMTA1的启动子序列特征和基因表达模式分析[J]. 作物学报, 2025, 51(7): 1969-1978. |
| [13] | 梁红凯, 赵苏蒙, 陆琼, 周鹏, 智慧, 刁现民, 贺强. 谷子微核心种质的构建[J]. 作物学报, 2025, 51(6): 1435-1444. |
| [14] | 方应浩, 周波, 陈茹梅, 杨文竹, 秦慧民. 基于RNA-seq和PER-seq联合分析探究ZmHDZ6表达调控网络[J]. 作物学报, 2025, 51(4): 958-968. |
| [15] | 潘炬忠, 韦萍, 朱德平, 邵胜雪, 陈珊珊, 韦雅倩, 高维维. 水稻转录因子OsERF104的克隆和功能研究[J]. 作物学报, 2025, 51(4): 900-913. |
|
||