欢迎访问作物学报,今天是
作物学报 ›› 2019, Vol. 45 ›› Issue (2): 235-247.doi: 10.3724/SP.J.1006.2019.84063
邹雪1,2,丁凡1,余金龙1,彭洁2,邓孟胜2,王宇2,刘丽芳1,余韩开宗1,陈年伟1,王西瑶2,*( )
Xue ZOU1,2,Fan DING1,Jin-Long YU1,Jie PENG2,Meng-Sheng DENG2,Yu WANG2,Li-Fang LIU1,Kai-Zong YU-HAN1,Nian-Wei CHEN1,Xi-Yao WANG2,*()
摘要:
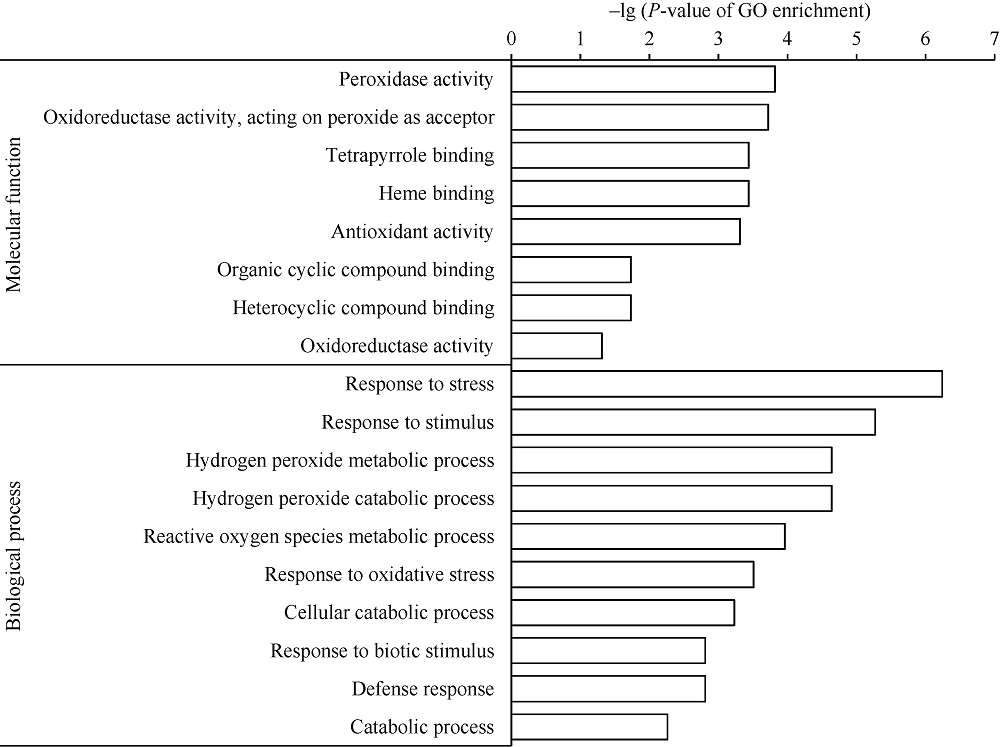
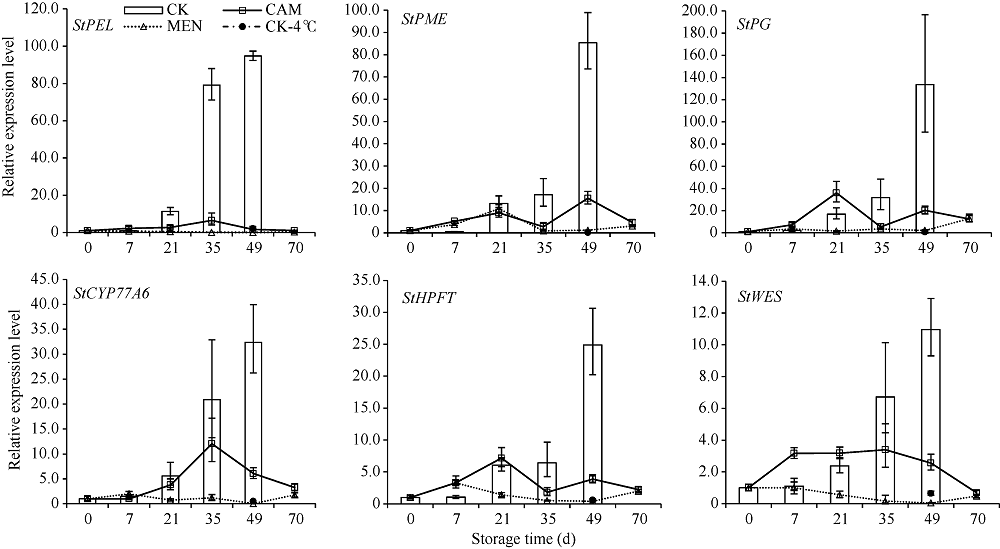
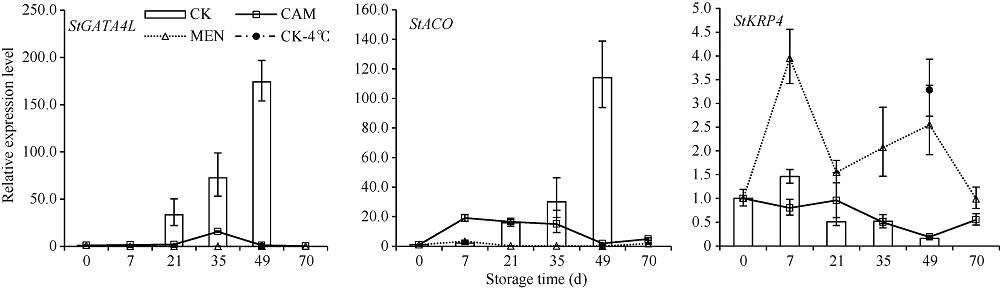
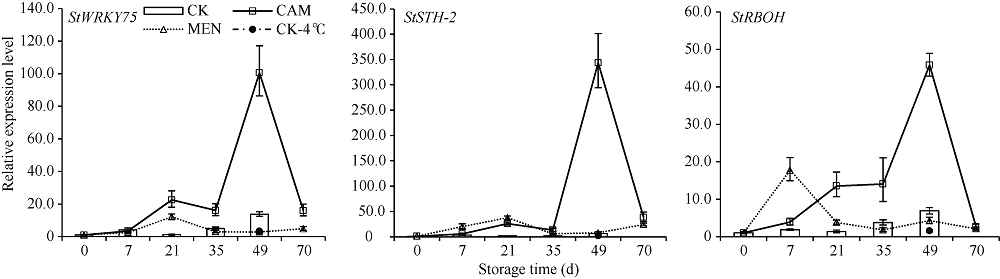
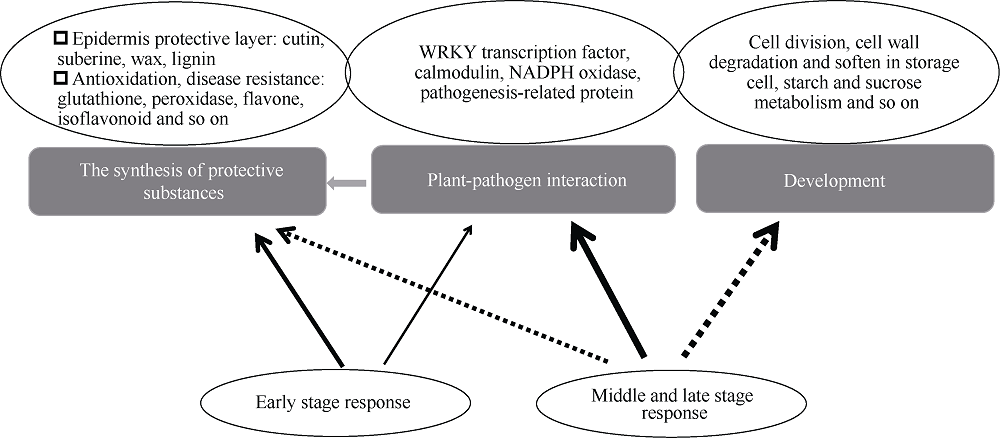
马铃薯块茎过早萌芽会降低商品价值, 本试验比较挥发性物质的抑芽效应, 并从转录和蛋白水平分析其作用机制。结果表明, 抑芽能力薄荷醇?樟脑?萘, 萌芽受抑降低代谢消耗, 薄荷醇处理180 d时的重量损失只有对照损失的36%。樟脑处理萌芽块茎3 d引起表达显著上调(或下调)的基因和蛋白分别有1227 (299)和296 (204)个, 主要参与响应刺激、防御反应。贮藏期间, 果胶代谢基因PEL、PME、PG, 角质合成基因CYP77A6、HPFT、WES, 乙烯合成基因ACO以及转录因子编码基因GATA4L的表达量随时间升高。樟脑早期不同程度地刺激这些基因表达, 中后期则抑制, 49 d时只有对照的0.68%~23.35%。薄荷醇使上述基因表达保持低水平, 但可提高细胞周期负控基因KRP4的表达, 为对照的15.9倍。植物病原菌互作通路中的基因WRKY75、STH-2、RBOH表达受樟脑诱导并在后期高表达。樟脑和薄荷醇均能抑制生长发育基因的表达, 造成芽死亡, 降低贮藏损耗。前者早期能促进合成保护性物质, 萌芽时有更强烈的抗菌反应; 后者则阻碍细胞分裂。
| [1] | 肖关丽, 郭华春 . 不同生理年龄马铃薯种薯芽中的内源激素含量变化及其对马铃薯植株生长发育的影响. 植物生理学报, 2007,43:818-820. |
| Xiao G L, Guo H C . Changes in endogenous hormone contents in bud of seed potato (Solanum tuberosum L.) with different physiological ages and its effect on growth and development. Plant Physiol J, 2007,43:818-820 (in Chinese with English abstract). | |
| [2] |
Daniels-Lake B J, Pruski K, Prange R K . Using ethylene gas and chlorpropham potato sprout inhibitors together. Potato Res, 2011,54:223-236.
doi: 10.1007/s11540-011-9188-z |
| [3] |
Vijay P, Ezekiel R, Pandey R . Use of CIPC as a potato sprout suppressant: health and environmental concerns and future options. Qual Assur Safety Crops Foods, 2018,10:17-24.
doi: 10.3920/QAS2017.1088 |
| [4] |
Gómez-Castillo D . Effects of essential oils on sprout suppression and quality of potato cultivars. Postharvest Biol Technol, 2013,82:15-21.
doi: 10.1016/j.postharvbio.2013.02.017 |
| [5] |
Hartmans K J . The use of carvone in agriculture: sprout suppression of potatoes and antifungal activity against potato tuber and other plant diseases. Ind Crops Prod, 1995,4:3-13.
doi: 10.1016/0926-6690(95)00005-W |
| [6] |
Oosterhaven K, Poolman B, Smid E J . S-carvone as a natural potato sprout inhibiting, fungistatic and bacteristatic compound. Ind Crops Prod, 1995,4:23-31.
doi: 10.1016/0926-6690(95)00007-Y |
| [7] |
Teper-Bamnolker P, Dudai N, Fischer R, Belausov E, Zemach H, Shoseyov O, Eshel D . Mint essential oil can induce or inhibit potato sprouing by differential alteration of apical meristem. Planta, 2010,232:179-186.
doi: 10.1007/s00425-010-1154-5 pmid: 20390295 |
| [8] |
Weerd J W, Thornton M K, Shafii B . Sprout suppressing residue levels of 1,4-dimethylnaphthalene (1,4DMN) in potato cultivars. Am J Potato Res, 2010,87:434-445.
doi: 10.1007/s12230-010-9146-3 |
| [9] |
Campbell M A, Gleichsner A, Alsbury R, Horvath D, Suttle J . The sprout inhibitors chlorpropham and 1,4-dimethylnaphthalene elicit different transcriptional profiles and do not suppress growth through a prolongation of the dormant state. Plant Mol Biol, 2010,73:181-189.
doi: 10.1007/s11103-010-9607-6 pmid: 20135197 |
| [10] |
Campbell M A, Gleichsner A, Hilldorfer L, Horvath D, Suttle J . The sprout inhibitor 1,4-dimethylnaphthalene induces the expression of the cell cycle inhibitors KRP1 and KRP2 in potatoes. Funct Integr Genomics, 2012,12:533-541.
doi: 10.1007/s10142-011-0257-9 pmid: 22113341 |
| [11] |
Li L Q, Zou X, Deng M S, Peng J, Huang X L, Lu X, Fang C C, Wang X Y . Comparative morphology, transcription, and proteomics study revealing the key molecular mechanism of camphor on the potato tuber sprouting effect. Int J Mol Sci, 2017,18:2280.
doi: 10.3390/ijms18112280 pmid: 29084178 |
| [12] |
Liu B L, Zhang N, Wen Y K, Jin X, Yang J W, Si H J, Wang D . Transcriptomic changes during tuber dormancy release process revealed by RNA sequencing in potato. J Biotechnol, 2015,198:17-30.
doi: 10.1016/j.jbiotec.2015.01.019 pmid: 25661840 |
| [13] |
Yang Y, Qiang X, Owsiany K, Zhang S, Thannhauser T W, Li L . Evaluation of different multidimensional LC-MS/MS pipelines for isobaric tags for relative and absolute quantitation (iTRAQ)- based proteomic analysis of potato tubers in response to cold storage. J Proteome Res, 2011,10:4647-4660.
doi: 10.1021/pr200455s pmid: 21842911 |
| [14] |
The Potato Genome Sequencing Consortium. Genome sequence and analysis of the tuber crop potato. Nature, 2011,475:189-195.
doi: 10.1038/nature10158 pmid: 21743474 |
| [15] |
Mortazavi A, Williams B A, McCue K, Schaeffer L, Wold B . Mapping and quantifying mammalian transcriptomes by RNA-Seq. Nat Methods, 2008,5:621-628.
doi: 10.1038/nmeth.1226 |
| [16] |
邹雪, 邓孟胜, 李立芹, 余金龙, 丁凡, 黄雪丽, 彭洁, 帅禹, 蔡诚诚, 王西瑶 . 油菜素内酯合成和信号转导基因在马铃薯块茎贮藏期间的表达变化及对萌芽的影响. 作物学报, 2017,43:811-820.
doi: 10.3724/SP.J.1006.2017.00811 |
|
Zou X, Deng M S, Li L Q, Yu J L, Ding F, Huang X L, Peng J, Shuai Y, Cai C C, Wang X Y . Expression changes of genes related to brassinosteroid biosynthesis and signal transduction during potato storage and its effect on tuber sprouting. Acta Agron Sin, 2017,43:811-820 (in Chinese with English abstract).
doi: 10.3724/SP.J.1006.2017.00811 |
|
| [17] |
Dixon R A . Natural products and plant disease resistance. Nature, 2001,411:843-847.
doi: 10.1038/35081178 |
| [18] |
Kobayashi M, Ohura I, Kawakita K, Yokota N, Fujiwara M, Shimamoto K, Doke N, Yoshioka H . Calcium-dependent protein kinases regulate the production of reactive oxygen species by potato NADPH oxidase. Plant Cell, 2007,19:1065-1080.
doi: 10.1105/tpc.106.048884 pmid: 17400895 |
| [19] |
Baydar H, Karadoğan T . The effects of volatile oils on in vitro potato sprout growth. Potato Res, 2003,46:1-8.
doi: 10.1007/BF02736098 |
| [20] |
马进, 郑钢, 裴翠明, 张振亚 . 基于iTRAQ质谱分析技术筛选南方型紫花苜蓿根部响应盐胁迫差异表达蛋白. 农业生物技术学报, 2016,24:497-509.
doi: 10.3969/j.issn.1674-7968.2016.04.004 |
|
Ma J, Zheng G, Pei C M, Zhang Z Y . Screening differentially expressed proteins in southern type alfalfa (Medicago sativa ‘Millenium’) root upon salt stress by iTRAQ protein mass spectrometry. J Agric Biotechnol, 2016,24:497-509 (in Chinese with English abstract).
doi: 10.3969/j.issn.1674-7968.2016.04.004 |
|
| [21] | Takahashi K, Niwa H, Yokota N, Kubota K, Inoue H . Widespread tissue expression of nepenthesis-like aspartic protease genes in Arabidopsis thaliana. Plant Physiol Biol, 2008,46:724-729. |
| [22] | 李合生 . 现代植物生理学(第3版). 北京: 高等教育出版社, 2012. pp 245-246. |
| Li H S . Modern Plant Physiology, 3rd edn. Beijing: Higher Education Press, 2012. pp 245-246(in Chinese). | |
| [23] |
Coleman W K, Dioxide C . Oxygen and ethylene effects on potato tuber dormancy release and sprout growth. Ann Bot, 1998,82:21-27
doi: 10.1006/anbo.1998.0645 |
| [24] |
Hartmann A, Senning M, Hedden P, Sonnewald U, Sonnewald S . Reactivation of meristem activity and sprout growth in potato tubers require both cytokinin and gibberellin. Plant Physiol, 2011,155:776-796.
doi: 10.1104/pp.110.168252 pmid: 21163959 |
| [25] |
Külen O, Stushnoff C, Davidson R D, Holm D G . Gibberelllic acid and ethephon alter potato minituber bud dormancy and improve seed tuber yield. Am J Potato Res, 2011,88:167-174.
doi: 10.1007/s12230-010-9178-8 |
| [26] |
Amita C, Sane V A, Nath P . Differential expression of pectate lyase during ethylene-induced postharvest softening of mango (Mangifera indica var. Dashehari). Physiol Planta, 2006,128:546-555.
doi: 10.1111/j.1399-3054.2006.00752.x |
| [27] |
Singh A P, Pandey S P, Rajluxmi, Pandey S, Nath P, Sane A P . Transcriptional activation of a pectate lyase gene,RbPel1, during petal abscission in rose. Postharvest Biol Technol, 2011,60:143-148.
doi: 10.1016/j.postharvbio.2010.12.014 |
| [28] |
Ranftl Q L, Bastakis E, Klermund C, Schwechheimer C . LLM- domain containing B-GATA factors control different aspects of cytokinin-regulated development in Arabidopsis thaliana. Plant Physiol, 2016,170:2295-2311.
doi: 10.1104/pp.15.01556 pmid: 26829982 |
| [29] |
Luo X M, Lin W H, Zhu S W, Zhu J Y, Sun Y, Fan X Y, Cheng M L, Hao Y Q, Oh E, Tian M M, Liu L J, Zhang M, Xie Q, Chong K, Wang Z Y . Integration of light- and brassinosteroid-signaling pathways by a GATA transcription factor in Arabidopsis. Dev Cell, 2010,19:872-883.
doi: 10.1016/j.devcel.2010.10.023 pmid: 3022420 |
| [30] |
Shin J M, Chung K M, Sakamoto S, Kojima S, Yeh C M, Ikeda M, Mitsuda N, Ohme-Takagi M . The chimeric repressor for the GATA4 transcription factor improves tolerance to nitrogen deficiency in Arabidopsis. Plant Biotechnol, 2017,34:151-158.
doi: 10.5511/plantbiotechnology.17.0727a |
| [31] | Leene J V, Hollunder J, Eeckhout D, Persiau G, Slijke E V D, Stals H . Targeted interactomics reveals a complex core cell cycle machinery in Arabidopsis thaliana. Mol Sys Biol, 2010,6:397. |
| [32] |
Sang E J, Yoko O, Jaesung N, Masaaki U, Gyung-Tae K . Kip-related protein 3 is required for control of endoreduplication in the shoot apical meristem and leaves of Arabidopsis. Mol Cells, 2013,35:47-53.
doi: 10.1007/s10059-013-2270-4 pmid: 23314608 |
| [33] |
Cheng Y, Cao L, Wang S, Li Y P, Shi X Z . Downregulation of multiple CDK inhibitor ICK/KRP genes upregulates the E2F pathway and increases cell proliferation, and organ and seed sizes in Arabidopsis. Plant J, 2013,75:642-655.
doi: 10.1111/tpj.12228 pmid: 23647236 |
| [34] |
Constabel C P, Brisson N . The defense-related STH-2 gene product of potato shows race-specific accumulation after inoculation with low concentrations of Phytophthora infestans zoospores. Planta, 1992,188:289-295.
doi: 10.1007/BF00192794 pmid: 24178317 |
| [35] |
Constabel C P, Bertrand C, Brisson N . Transgenic potato plants overexpressing the pathogenesis-related STH-2 gene show unaltered susceptibility to Phytophthora infestans and potato virus X. Plant Mol Biol, 1993,22:775-782.
doi: 10.1007/BF00027364 pmid: 8358029 |
| [36] |
El-Banna A, Hajirezaei M R, Wissing J, Ali Z, Vaas L, Heine-Dobbernack E, Jacobsen H J, Schumacher H M, Kiesecker H . Over-expression of PR-10a leads to increased salt and osmotic tolerance in potato cell cultures. J Biotechnol, 2010,150:277-287.
doi: 10.1016/j.jbiotec.2010.09.934 pmid: 20854851 |
| [37] | Park S, Gupta R, Krishna R, Kim S T, Lee D Y, Hwang D J, Bae S C, Ahn I P . Proteome analysis of disease resistance against Ralstonia solanacearum in potato cultivar CT206-10. Plant Pathol J, 2016,32:25-32. |
| [1] | 陈国欢, 张锐, 李艳迪, 赵佳琪, 任湧涛, 张天赐, 郭华春, 李俊, 杨芳. 外源硒叶面喷施对浅紫色马铃薯块茎花青素合成的影响[J]. 作物学报, 2026, 52(6): 1876-1890. |
| [2] | 王亚, 赵宜婷, 王宙, 杨俊芳, 张宏斌, 曹越. 转录组-代谢组联合分析蓖麻蜡质合成相关基因[J]. 作物学报, 2026, 52(6): 1774-1787. |
| [3] | 陈雪燕, 何华川, 李政嘉, 董新盼, 李藕琪, 刘小云, 李丹萍, 陈志伟, 刘国霞, 吕胜源, 吴印莹, 赵振东, 曹新有, 万何平. 水培盐碱复合胁迫下‘济麦60’苗期根系有机酸分泌动态变化及其转录调控机制[J]. 作物学报, 2026, 52(6): 1859-1875. |
| [4] | 王文辕, 燕雪嘉, 刘玉霖, 孙晓彤, 李亚楠, 唐鑫华, 石瑛. 耐弱光马铃薯品种筛选及转录因子编码基因StPIF3的克隆与功能分析[J]. 作物学报, 2026, 52(6): 1631-1645. |
| [5] | 邹仪妹, 徐敏, 汪海洋, 姚辉, 王加峰, 刘浩, 任代胜. 两系不育系水稻幼苗根系响应盐胁迫的转录因子调控网络鉴定[J]. 作物学报, 2026, 52(6): 1728-1742. |
| [6] | 蔡兆琴, 何观咏, 何文, 阮丽霞, 梁振华, 李永珍, 李恒锐, 陈会鲜. 木薯分枝发育过程的动态转录组分析与关键基因发掘[J]. 作物学报, 2026, 52(5): 1430-1441. |
| [7] | 张曦, 王广恩, 李邵琦, 刘祎, 李俊兰, 钱玉源. 基于转录组测序解析陆海杂交姊妹系马克隆值差异的形成机制[J]. 作物学报, 2026, 52(5): 1442-1458. |
| [8] | 韩亚鑫, 何冠华, 张小琼, 张登峰, 李永祥, 刘旭洋, 王天宇, 黎裕, 邹华文, 李春辉. 基于RNA-Seq和BSA-Seq联合分析挖掘玉米侧根密度基因资源[J]. 作物学报, 2026, 52(5): 1341-1352. |
| [9] | 杨亚莉, 徐明睿, 马越飞, 海艺蕊, 刘凯栋, 刘万茂, 孙颖. 玉米根尖及整根响应缺铁的转录组比较研究[J]. 作物学报, 2026, 52(4): 1006-1021. |
| [10] | 田立涛, 丁宁, 王树林, 齐恩芳, 张荣, 王蕊蕊, 马利雯, 李建武, 杨江伟. 马铃薯Argonaute基因家族鉴定及晚疫病诱导表达分析[J]. 作物学报, 2026, 52(4): 1116-1126. |
| [11] | 汪玲, 胡好, 宋家凤, 程洁蓝, 陈颖, 郑婷婷, 吕钊彦, 朱晓彪, 侯华兰. 马铃薯UDP-糖基转移酶基因StUGT52的克隆及功能验证[J]. 作物学报, 2026, 52(3): 665-676. |
| [12] | 马亮, 马璐, 张舒钰, 章慧敏, 王仁明, 宋旭东, 张振良, 冒宇翔, 陆虎华, 陈国清, 郝德荣, 周广飞. 玉米苞叶数目转录组分析及候选基因鉴定[J]. 作物学报, 2026, 52(3): 790-801. |
| [13] | 杨宗桃, 杨婷, 王禹童, 艾静, 李燕烨, 刘家勇, 邓军, 赵勇, 张跃彬. 甘蔗CLC基因家族鉴定与表达分析[J]. 作物学报, 2026, 52(3): 722-734. |
| [14] | 张宇, 刘芳, 蔡诚诚, 杨小华, 吉阿么石扎, 杨元军, 王西瑶. 溴乙烷与赤霉素协同处理破除马铃薯块茎休眠的机理初探[J]. 作物学报, 2026, 52(3): 825-838. |
| [15] | 于永超, 刘明, 靳容, 赵鹏, 张强强, 王静, 朱晓亚, 唐忠厚. 甘薯高氮徒长的生理机制和转录组分析研究[J]. 作物学报, 2026, 52(3): 813-824. |
|
||