欢迎访问作物学报,今天是
作物学报 ›› 2024, Vol. 50 ›› Issue (6): 1451-1466.doi: 10.3724/SP.J.1006.2024.34121
刘震1( ), 陈丽敏2, 李志涛2, 朱金勇2, 王玮璐2, 齐喆颖2, 姚攀锋1, 毕真真2, 孙超2, 白江平3, 刘玉汇1,*()
LIU Zhen1(), CHEN Li-Min2, LI Zhi-Tao2, ZHU Jin-Yong2, WANG Wei-Lu2, QI Zhe-Ying2, YAO Pan-Feng1, BI Zhen-Zhen2, SUN Chao2, BAI Jiang-Ping3, LIU Yu-Hui1,*()
摘要:
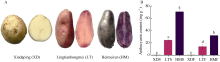
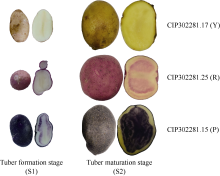
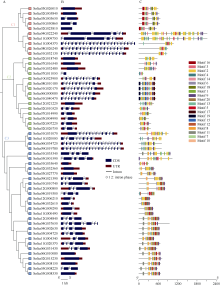
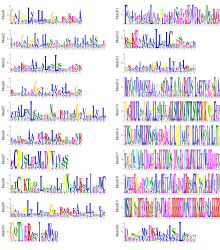
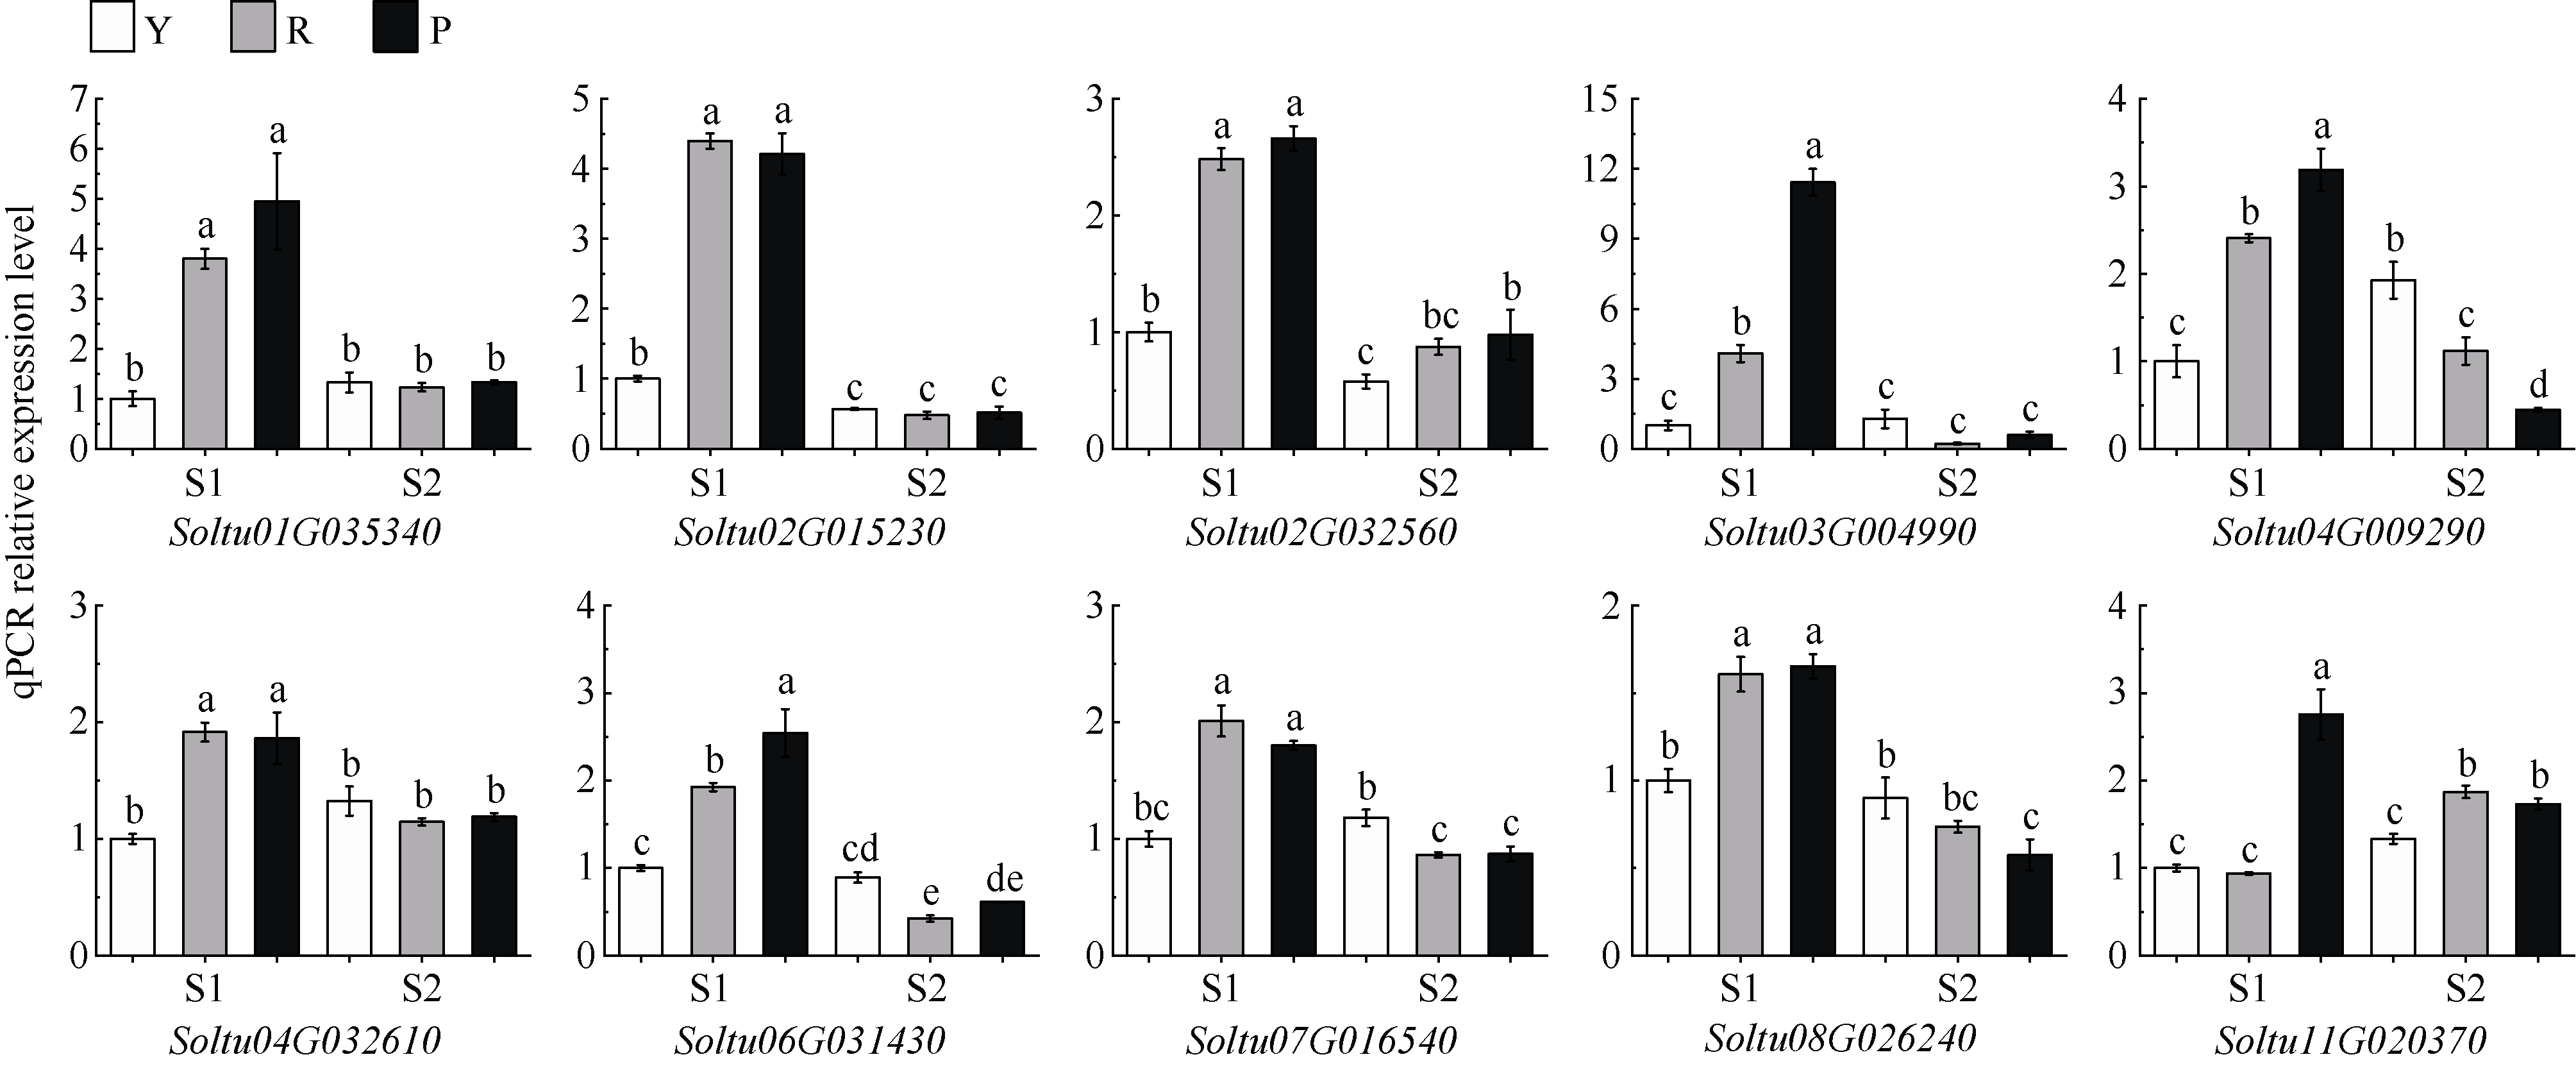
ARM蛋白重复序列(Armadillo repeats)广泛存在于高等植物中, 它们参与多种细胞过程, 如信号转导、核转运以及对多种生物/非生物胁迫的响应。本研究在马铃薯(Solanum tuberosum L.)全基因组水平下鉴定出了54个马铃薯ARM基因家族成员(StARMs), 它们不均匀的分布在12条染色体上。根据其蛋白结构和系统发育特征, 将54个StARMs分为3个亚家族。片段重复事件在马铃薯ARM基因家族的扩展中起主要作用。共线性分析发现, StARMs与番茄(Solanum lycopersicum)、拟南芥(Arabidopsis)、甘蓝(Brassica oleracea)、水稻(Oryza sativa)、玉米(Zea mays)分别有51对、17对、25对、6对和10对直系同源基因, 这些基因均在纯化选择下进化。RNA-seq数据分析发现, 4个StARM基因在匍匐茎中特异表达, 2个StARM基因在根和心皮中特异表达, 1个StARM基因在块茎中特异表, 还有一些StARM基因参与了马铃薯对生物/非生物胁迫的响应。此外, 本研究对3个不同颜色马铃薯块茎组织(薯皮和薯肉)进行了RNA-seq测序, 分析了54个StARMs在不同颜色马铃薯块茎组织中的表达模式, 并利用qPCR分析了StARMs 在3个不同颜色块茎杂交子代薯肉中的相对表达量, 筛选出了4个可能参与马铃薯块茎花色素苷生物合成的候选基因。本研究为进一步了解StARM基因家族的特征, 深入分析StARM基因在马铃薯抵御生物/非生物胁迫和调控块茎花色素苷生物合成中的功能提供了理论依据。
| [1] | Sharma M, Pandey A, Pandey G K. β-catenin in plants and animals: common players but different pathways. Front Plant Sci, 2014, 5: 00143. |
| [2] |
Xu C, Min J. Structure and function of WD40 domain proteins. Protein Cell, 2011, 2: 202-214.
doi: 10.1007/s13238-011-1018-1 pmid: 21468892 |
| [3] | Zhang R, Kennedy M A. Current understanding of the structure and Function of pentapeptide pepeat proteins. Biomolecules, 2021, 11: 638. |
| [4] |
Das A K, Cohen P T W, Barford D. The structure of the tetratricopeptide repeats of protein phosphatase 5: implications for TPR-mediated protein-protein interactions. EMBO J, 1998, 17: 1192-1199.
doi: 10.1093/emboj/17.5.1192 pmid: 9482716 |
| [5] | Sharma M, Pandey G K. Expansion and function of repeat domain proteins during stress and development in plants. Front Plant Sci, 2016, 6: 1218. |
| [6] |
Huber A H, Nelson W J, Weis W I. Three-dimensional structure of the armadillo repeat region of beta-catenin. Cell, 1997, 90: 871-882.
pmid: 9298899 |
| [7] | Hatzfeld M. The armadillo family of structural proteins. Int Rev Cytol, 1998, 186: 179-224. |
| [8] |
Amador V, Monte E, Garcı́a-Martı́nez J L, Prat S. Gibberellins signal nuclear import of PHOR1, a photoperiod-responsive protein with homology to drosophila armadillo. Cell, 2001, 106: 343-354.
pmid: 11509183 |
| [9] | Bergler J, Hoth S. Plant U-box armadillo repeat proteins AtPUB18 and AtPUB19 are involved in salt inhibition of germination in Arabidopsis. Plant Biol, 2011, 13: 725-730. |
| [10] |
Stone S L, Anderson E M, Mullen R T, Goring D R. ARC1 is an E3 ubiquitin ligase and promotes the ubiquitination of proteins during the rejection of self-incompatible Brassica pollen. Plant Cell, 2003, 15: 885-898.
doi: 10.1105/tpc.009845 pmid: 12671085 |
| [11] |
Kirsch C, Logemann E, Lippok B, Schmelzer E, Hahlbrock K. A highly specific pathogen-responsive promoter element from the immediate-early activated CMPG1 gene in Petroselinum crispum. Plant J, 2001, 26: 217-227.
pmid: 11389762 |
| [12] | Sharma M, Pandey G K. OsPUB75, an Armadillo/U-box protein interacts with GSK3 kinase and functions as negative regulator of abiotic stress responses. Environ Exp Bot, 2019, 161: 388-398. |
| [13] | Zhang J X, Wang C, Yang C Y, Wang J Y, Chen L, Bao X M, Zhao Y X, Zhang H, Liu J. The role of Arabidopsis AtFes1A in cytosolic Hsp70 stability and abiotic stress tolerance. Plant J, 2010, 62: 539-548. |
| [14] | Mandal A, Mishra A K, Dulani P, Muthamilarasan M, Shweta S, Prasad M. Identification, characterization, expression profiling, and virus-induced gene silencing of armadillo repeat-containing proteins in tomato suggest their involvement in tomato leaf curl New Delhi virus resistance. Funct Integr Genomic, 2018, 18: 101-111. |
| [15] | Kim S, Choi H, Ryu H J, Park J H, Kim M D, Kim S Y. ARIA, an Arabidopsis ARM repeat protein interacting with a transcriptional regulator of abscisic acid-responsive gene expression, is a novel abscisic acid signaling component. Plant Physiol, 2004, 136: 3639-3648. |
| [16] |
Samuel M A, Salt J N, Shiu S H, Goring D R. Multifunctional ARM repeat domains in plants. Int Rev Cytol, 2006, 253: 1-26.
pmid: 17098053 |
| [17] |
Trujillo M. News from the PUB: plant U-box type E3 ubiquitin ligases. J Exp Bot, 2018, 69: 371-384.
doi: 10.1093/jxb/erx411 pmid: 29237060 |
| [18] | Mudgil Y, Shiu S H, Stone S L, Salt J N, Goring D R. A large complement of the predicted Arabidopsis ARM repeat proteins are members of the U-box E3 ubiquitin ligase family. Plant Physiol, 2004, 134: 59-66. |
| [19] |
Sharma M, Singh A, Shankar A, Pandey A, Baranwal V, Kapoor S, Tyagi A K, Pandey G K. Comprehensive expression analysis of rice armadillo gene family during abiotic stress and development. DNA Res, 2014, 21: 267-283.
doi: 10.1093/dnares/dst056 pmid: 24398598 |
| [20] | Visser R G F, Bachem C W B, Boer J M, Bryan G J, Chakrabati S K, Feingold S, Gromadka R, Ham R C H J, Huang S, Jacobs J M E, Kuznetsov B, Melo P E, Milbourne D, Orjeda G, Sagredo B, and Tang X. Sequencing the potato genome: outline and first results to come from the elucidation of the sequence of the world’s third most important food crop. Am J Potato Res, 2009, 86: 417. |
| [21] | Fossen T, Andersen Ø M. Anthocyanins from tubers and shoots of the purple potato, Solanum tuberosum. J Hortic Sci Biotechnol, 2000, 7: 360-363. |
| [22] |
Igwe E O, Charlton K E, Roodenrys S, Kent K, Fanning K, Netzel M E. Anthocyanin-rich plum juice reduces ambulatory blood pressure but not acute cognitive function in younger and older adults: a pilot crossover dose-timing study. Nutr Res, 2017, 47: 28-43.
doi: S0271-5317(17)30482-7 pmid: 29241576 |
| [23] |
Castellarin S D, Pfeiffer A, Sivilotti P, Degan M, Peterlunger E, Gaspero G. Transcriptional regulation of anthocyanin biosynthesis in ripening fruits of grapevine under seasonal water deficit. Plant Cell Environ, 2007, 30: 1381-1399.
doi: 10.1111/j.1365-3040.2007.01716.x pmid: 17897409 |
| [24] | Liu Z, Li Y, Zhu J, Ma W, Li Z, Bi Z, Sun C, Bai J, Zhang J, Liu Y. Genome-wide identification and analysis of the NF-Y gene family in potato (Solanum tuberosum L.). Front Genet, 2021, 12: 739989. |
| [25] | Gasteiger E, Hoogland C, Gattiker A, Duvaud S, Wilkins M R, Appel R D, Bairoch A. Protein identification and analysis tools on the expasy server. Proteomics Protocols Handbook, 2005, 53: 571-607. |
| [26] | Hu B, Jin J, Guo A Y, Zhang H, Luo J, Gao G. GSDS 2.0: an upgraded gene feature visualization server. Bioinformatics, 2014, 31: 1296-1297. |
| [27] |
Bailey T L, Boden M, Buske F A, Frith M, Grant C E, Clementi L, Ren J, Li W W, Noble W S. MEME SUITE: tools for motif discovery and searching. Nucleic Acids Res, 2009, 37: 202-208.
doi: 10.1093/nar/gkp335 pmid: 19458158 |
| [28] | Wang Y, Tang H, Debarry D, Tan X, Li J, Wang X, Lee T H, Jin H, Marler B, Guo H. MCScanX: a toolkit for detection and evolutionary analysis of gene synteny and collinearity. Nucleic Acids Res, 2012, 40: e49. |
| [29] |
Krzywinski M, Schein J, Birol I, Connors J, Gascoyne R, Horsman D, Jones S J, Marra M A. Circos: an information aesthetic for comparative genomics. Genome Res, 2009, 19: 1639-1645.
doi: 10.1101/gr.092759.109 pmid: 19541911 |
| [30] |
Wang D, Zhang Y, Zhang Z, Zhu J, Yu J. KaKs_Calculator 2.0: a toolkit incorporating gamma-series methods and sliding window strategies. Genom Proteom Bioinf, 2010, 8: 77-80.
doi: 10.1016/S1672-0229(10)60008-3 pmid: 20451164 |
| [31] |
Tang X, Zhang N, Si H, Calderón-Urrea A. Selection and validation of reference genes for RT-qPCR analysis in potato under abiotic stress. Plant Methods, 2017, 13: 85.
doi: 10.1186/s13007-017-0238-7 pmid: 29075311 |
| [32] |
Livak K J, Schmittgen T D. Analysis of relative gene expression data using real-time quantitative PCR and the 2-ΔΔCT method. Methods, 2001, 25: 402-408.
doi: 10.1006/meth.2001.1262 pmid: 11846609 |
| [33] | Chen C, Xia R, Chen H, He Y. TBtools, a toolkit for biologists integrating various HTS-data handling tools with a user-friendly interface. BioRxiv, 2018, 6: 289660. |
| [34] | Cannon S B, Mitra A, Baumgarten A, Young N D, May G. The roles of segmental and tandem gene duplication in the evolution of large gene families in Arabidopsis thaliana. BMC Plant Biol, 2004, 4: 10. |
| [35] | Wang H, Lu Y, Jiang T, Berg H, Li C, Xia Y. The Arabidopsis U-box/ARM repeat E3 ligase AtPUB4 influences growth and degeneration of tapetal cells, and its mutation leads to conditional male sterility. Plant J, 2013, 74: 511-523. |
| [36] | Gebert M, Dresselhaus T, Sprunck S. F-actin organization and pollen tube tip growth in Arabidopsis are dependent on the gametophyte-specific armadillo repeat protein ARO1. Plant Cell, 2008, 20: 2798-2814. |
| [37] | Wang H, Lu Y, Jiang T, Berg H, Li C, Xia Y. The Arabidopsis U-box/ARM repeat E3 ligase AtPUB4 influences growth and degeneration of tapetal cells, and its mutation leads to conditional male sterility. Plant J, 2013, 74: 511-523. |
| [38] | Li W, Ahn I P, Ning Y, Park C H, Zeng L, Whitehill J G A, Lu H, Zhao Q, Ding B, Xie Q, Zhou J, Dai L. The U-Box/ARM E3 ligase PUB13 regulates cell death, defense, and flowering time in Arabidopsis. Plant Physiol, 2012, 15: 239-250. |
| [39] | Zhou J, Lu D, Xu G, Finlayson S A, He P, Shan L. The dominant negative ARM domain uncovers multiple functions of PUB13 in Arabidopsis immunity, flowering, and senescence. J Exp Bot, 2015, 66: 3353-3366. |
| [40] | Dias A P, Braun E L, McMullen M D, Grotewold E. Recently duplicated maize R2R3 Myb genes provide evidence for distinct mechanisms of evolutionary divergence after duplication. Plant Physiol, 2003, 131: 610-620. |
| [41] | Kim E J, Lee S H, Park C H, Kim S H, Hsu C C, Xu S, Wang Z Y, Kim S K, Kim T W. Plant U-Box40 mediates degradation of the brassinosteroid-responsive transcription factor BZR1 in Arabidopsis roots. Plant Cell, 2019, 3: 791-808. |
| [42] | Feng W, Liu Y, Cao Y, Zhao Y, Zhang H, Sun F, Yang Q, Li W, Lu Y, Zhang X, Fu F, and Yu H. Maize ZmBES1/BZR1-3 and -9 transcription factors negatively regulate drought tolerance in transgenic Arabidopsis. Int J Mol Sci, 2022, 23: 6025. |
| [43] | Wang Y, Zhu Y, Jiang H, Mao Z, Zhang J, Fang H, Liu W, Zhang Z, Chen X, Wang N. The regulatory module MdBZR1-MdCOL6 mediates brassinosteroid- and light-regulated anthocyanin synthesis in apple. New Phytol, 2023, 238: 1516-1533. |
| [1] | 陈国欢, 张锐, 李艳迪, 赵佳琪, 任湧涛, 张天赐, 郭华春, 李俊, 杨芳. 外源硒叶面喷施对浅紫色马铃薯块茎花青素合成的影响[J]. 作物学报, 2026, 52(6): 1876-1890. |
| [2] | 左同鸿, 张贺翠, 曾静, 朱利泉. 甘蓝自交不亲和相关基因BoPUB3L的克隆与表达分析[J]. 作物学报, 2026, 52(6): 1698-1710. |
| [3] | 王文辕, 燕雪嘉, 刘玉霖, 孙晓彤, 李亚楠, 唐鑫华, 石瑛. 耐弱光马铃薯品种筛选及转录因子编码基因StPIF3的克隆与功能分析[J]. 作物学报, 2026, 52(6): 1631-1645. |
| [4] | 胡赵, 钱润, 谢丰璞, 应素平. 水稻SPX基因家族鉴定及响应磷处理的表达分析[J]. 作物学报, 2026, 52(6): 1902-1912. |
| [5] | 田立涛, 丁宁, 王树林, 齐恩芳, 张荣, 王蕊蕊, 马利雯, 李建武, 杨江伟. 马铃薯Argonaute基因家族鉴定及晚疫病诱导表达分析[J]. 作物学报, 2026, 52(4): 1116-1126. |
| [6] | 汪玲, 胡好, 宋家凤, 程洁蓝, 陈颖, 郑婷婷, 吕钊彦, 朱晓彪, 侯华兰. 马铃薯UDP-糖基转移酶基因StUGT52的克隆及功能验证[J]. 作物学报, 2026, 52(3): 665-676. |
| [7] | 杨宗桃, 杨婷, 王禹童, 艾静, 李燕烨, 刘家勇, 邓军, 赵勇, 张跃彬. 甘蔗CLC基因家族鉴定与表达分析[J]. 作物学报, 2026, 52(3): 722-734. |
| [8] | 孟成, 王哲. 玉米ZmPFK基因家族全基因组鉴定及响应胁迫表达分析[J]. 作物学报, 2026, 52(3): 764-779. |
| [9] | 张宇, 刘芳, 蔡诚诚, 杨小华, 吉阿么石扎, 杨元军, 王西瑶. 溴乙烷与赤霉素协同处理破除马铃薯块茎休眠的机理初探[J]. 作物学报, 2026, 52(3): 825-838. |
| [10] | 徐强, 谢奎忠, 胡新元, 岳云, 董博, 罗爱花. 连作对马铃薯根际土壤线虫群落结构与功能的影响[J]. 作物学报, 2026, 52(2): 527-538. |
| [11] | 张力岚, 杨军, 王让剑. 基于WGCNA发掘茶树糖苷类香气前体含量性状相关的候选基因[J]. 作物学报, 2026, 52(2): 494-513. |
| [12] | 杨飚, 杜帅康, 张继旺, 石瑛, 张丽莉. 马铃薯III类POD基因家族的全基因组鉴定及其表达谱分析[J]. 作物学报, 2026, 52(2): 405-420. |
| [13] | 王雅致, 杨飚, 季香林, 石瑛, 张丽莉. 二倍体马铃薯抗旱资源鉴定及抗旱基因初步筛选[J]. 作物学报, 2026, 52(1): 72-84. |
| [14] | 田甲春, 葛霞, 李守强, 李梅, 田世龙, 张亚倩, 程建新, 李玉梅. 低O2高CO2贮藏环境延缓马铃薯块茎衰老的作用机制[J]. 作物学报, 2026, 52(1): 262-278. |
| [15] | 姬炫彤, 卞春松, 金黎平, 李森, 秦军红, 李广存. 不同耐旱型马铃薯根际微生物对干旱的响应[J]. 作物学报, 2026, 52(1): 165-177. |
|
||