欢迎访问作物学报,今天是
作物学报 ›› 2018, Vol. 44 ›› Issue (03): 397-404.doi: 10.3724/SP.J.1006.2018.00397
梁云飞1,*, 张林成1,*, 蒲全明2, 雷镇泽1, 施松梅1, 姜宇鹏1, 任雪松1, 高启国1,*( )
Yun-Fei LIANG1,**, Lin-Cheng ZHANG1,**, Quan-Ming PU2, Zhen-Ze LEI1, Song-Mei SHI1, Yu-Peng JIANG1, Xue-Song REN1, Qi-Guo GAO1,*()
摘要:
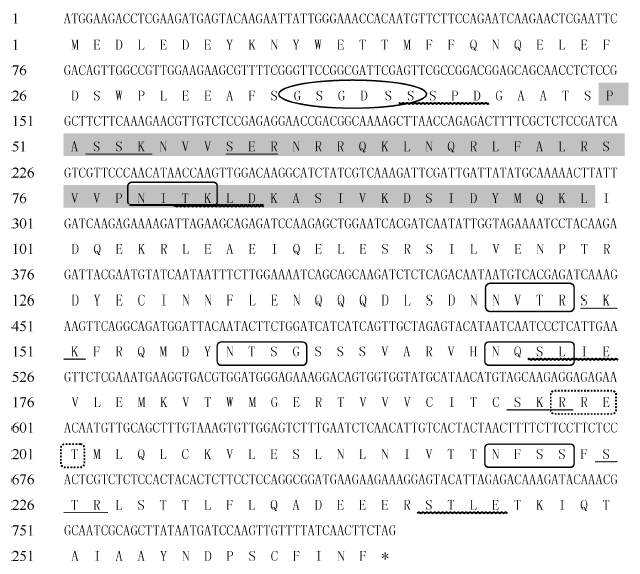
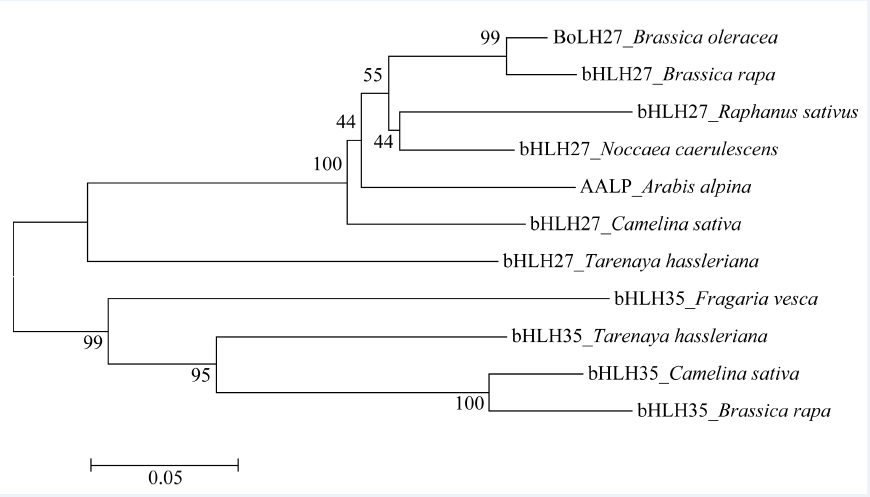
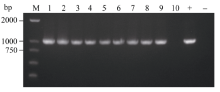
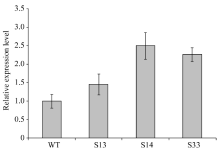
bHLH转录因子对植物生长发育、形态调控有重要作用, 为了研究BoLH27基因在甘蓝叶片发育及形态建成中的调控功能, 本文以甘蓝品种519为材料, 克隆出转录因子BoLH27基因。序列分析表明, 该基因含有一个795 bp的开放阅读框, 编码264个氨基酸, 具有一个保守的典型bHLH结构域。以农杆菌介导的遗传转化方法将正义BoLH27基因导入甘蓝品种519中以增强表达, 通过PCR筛选出9株T0代转基因单株, 结合T2代单株的qRT-PCR分析表明, 筛选的转基因植株内BoLH27基因的表达积累量明显高于野生型。试验基地隔离网内种植的转基因甘蓝表型明显, 主要表现为莲座期茎叶间距拉长、叶柄伸长以及植株茎和叶柄显示紫色, 植株叶片平展, 无向上向内卷曲趋势, 表明BoLH27基因可能对甘蓝叶片发育有重要的调控作用。
| [1] | Ludwig S R, Habera L F, Dellaporta S L, Wessler S R.Lc, a member of the maize R gene family responsible for tissue- specific anthocyanin production, encodes a protein similar to transcriptional activators and contains the myc-homology region. Proc Natl Acad Sci USA, 1989, 86: 7092-7096 |
| [2] | Ling H Q, Bauer P, Bereczky Z, Keller B, Ganal M.The tomato FER gene encoding a bHLH protein controls iron-uptake responses in roots.Proc Natl Acad Sci USA, 2002, 99: 13938-13943 |
| [3] | Kiribuchi K, Jikumaru Y, Kaku H, Minami E, Hasegawa M, Kodama O.Involvement of the basic helix-loop-helix transcription factor RERJ1 in wounding and drought stress responses in rice plants.Biosci Biotechnol Biochem, 2005, 69: 1042-1044 |
| [4] | Carreteropaulet L, Galstyan A, Roigvillanova I, Martínezgarcía J F, Bilbaocastro J R, Robertson D L.Genome-wide classification and evolutionary analysis of the bHLH family of transcription factors in Arabidopsis, poplar, rice, moss, and algae.Plant Physiol, 2010, 153: 1398-1412 |
| [5] | Pires N, Dolan L.Origin and diversification of basic-helix- loop-helix proteins in plants.Mol Biol Evol, 2010, 27: 862-874 |
| [6] | Grove C A, De M F, Barrasa M I, Newburger D E, Alkema M J, Bulyk M L.A multiparameter network reveals extensive divergence between C. elegans bHLH transcription factors. Cell, 2009, 138: 314-327 |
| [7] | Toledo-Ortiz G, Huq E, Quail P H.The Arabidopsis basic-helix-loop-helix transcription factor family. Plant Cell, 2003, 15: 1749-1770 |
| [8] | Li X, Duan X, Jiang H, Sun Y, Tang Y, Yuan Z.Genome-wide analysis of basic-helix-loop-helix transcription factor family in rice and Arabidopsis. Plant Physiol, 2006, 141: 1167-1184 |
| [9] | Atchley W R, Terhalle W, Dress A.Positional dependence, cliques, and predictive motifs in the bHLH protein domain.J Mol Evol, 1999, 48: 501-516 |
| [10] | Heim M A, Jakoby M, Werber M, Martin C, Weisshaar B, Bailey P C.The basic helix-loop-helix transcription factor family in plants: a genome-wide study of protein structure and functional diversity.Mol Biol Evol, 2003, 20: 735-747 |
| [11] | Yin J, Chang X, Kasuga T, Mai B, Reid M S, Jiang C Z.A basic helix-loop-helix transcription factor, PhFBH4, regulates flower senescence by modulating ethylene biosynthesis pathway in petunia.Hortic Res, 2015, 2: 15059-15068 |
| [12] | Ko S S, Li M J, Sun-Ben K M, Ho Y C, Lin Y J, Chuang M H. The bHLH142 transcription factor coordinates with TDR1 to modulate the expression of EAT1 and regulate pollen development in rice.Plant Cell, 2014, 26: 2486-2504 |
| [13] | Takahashi Y, Ebisu Y, Kinoshita T, Doi M, Okuma E, Murata Y. bHLH transcription factors that facilitate K+ uptake during stomatal opening are repressed by abscisic acid through phosphorylation. Sci Signal, 2013, 6: ra48 |
| [14] | Shen Q, Lu X, Yan T, Fu X, Lv Z, Zhang F.The jasmonate-responsive AaMYC2 transcription factor positively regulates artemisinin biosynthesis in Artemisia annua. New Phytol, 2016, 210: 1269-1281 |
| [15] | Kurbidaeva A, Ezhova T, Novokreshchenova M.Arabidopsis thaliana ICE2 gene: phylogeny, structural evolution and functional diversification from ICE1. Plant Sci, 2014, 229: 10-22 |
| [16] | Makkena S, Lamb R S.The bHLH transcription factor SPATULA is a key regulator of organ size in Arabidopsis thaliana. Plant Signal Behav, 2013, 8: e24140 |
| [17] | An R, Liu X, Wang R, Wu H, Liang S, Shao J, Qi Y, An L, Yu F.The over-expression of two transcription factors, ABS5/bHLH30 and ABS7/MYB101, leads to upwardly curly leaves.PLoS One, 2014, 9: e107637 |
| [18] | Nath U, Crawford B C, Carpenter R, Coen E.Genetic control of surface curvature.Science, 2003, 299: 1404-1407 |
| [19] | Qin G, Gu H, Zhao Y, Ma Z, Shi G, Yang Y.An indole-3-acetic acid carboxyl methyltransferase regulates Arabidopsis leaf development.Plant Cell, 2005, 17: 2693-2704 |
| [20] | Sarvepalli K, Nath U.Hyper-activation of the TCP4 transcription factor in Arabidopsis thaliana accelerates multiple aspects of plant maturation. Plant J, 2011, 67: 595-607 |
| [21] | Efroni I, Blum E, Goldshmidt A, Eshed Y.A protracted and dynamic maturation schedule underlies Arabidopsis leaf development. Plant Cell, 2008, 20: 2293-2306 |
| [22] | 莫晓婷. 玉米逆境相关转录因子的克隆与初步分析. 中国农业科学院硕士学位论文. 北京, 2013 |
| Mo X T.Cloning and Functional Characterization of Stress-related Transcription Factors in Maize. MS Thesis of Chinese Academy of Agricultural Sciences, Beijing,China, 2013 (in Chinese with English abstract) | |
| [23] | 何绍敏, 李春雨, 兰彩耘, 邹敏, 任雪松, 司军, 李成琼, 宋洪元. 转MLPK反义基因对甘蓝自交不亲和性的影响. 园艺学报, 2015, 42: 252-262 |
| He S M, Li C Y, Lan C Y, Zou M, Ren X S, Si J, Li C Q, Song H Y.Effect of antisense RNA of the MLPK gene on self-incompatibility in cabbage.Acta Hortic Sin, 2015, 42: 252-262 (in Chinese with English abstract) | |
| [24] | Heim M A, Jakoby M, Werber M, Martin C, Weisshaar B, Bailey P C.The basic helix-loop-helix transcription factor family in plants: a genome-wide study of protein structure and functional diversity.Mol Biol Evol, 2003, 20: 735-747 |
| [25] | Grotewold E, Sainz M B, Tagliani L, Hernandez J M, Bowen B, Chandler V L.Identification of the residues in the Myb domain of maize C1 that specify the interaction with the bHLH cofactor R.Proc Natl Acad Sci USA, 2000, 97: 13579-13584 |
| [26] | Bernhardt C, Lee M M, Gonzalez A, Zhang F, Lloyd A, Schiefelbein J.The bHLH genes GLABRA3 (GL3) and ENHANCER OF GLABRA3 (EGL3) specify epidermal cell fate in the Arabidopsis root. Development, 2003, 130: 6431-6439 |
| [27] | Zhang L Y, Bai M Y, Wu J, Zhu J Y, Wang H, Zhang Z.Antagonistic HLH/bHLH transcription factors mediate brassinosteroid regulation of cell elongation and plant development in rice and Arabidopsis. Plant Cell, 2009, 21: 3767-3780 |
| [28] | Meng Y, Li H, Wang Q, Liu B, Lin C.Blue light-dependent interaction between cryptochrome 2 and CIB1 regulates transcription and leaf senescence in soybean.Plant Cell, 2013, 25: 4405-4420 |
| [29] | Husbands A, Bell E M, Shuai B, Smith H M S, Springer P S. LATERAL ORGAN BOUNDARIES defines a new family of DNA-binding transcription factors and can interact with specific bHLH proteins.Nucl Acids Res, 2007, 35: 6663-6671 |
| [30] | Shuai B, Reynagapeña C G, Springer P S.The lateral organ boundaries gene defines a novel, plant-specific gene family.Plant Physiol, 2002, 129: 747-761 |
| [31] | Aguilar-Martínez J A, Sinha N. Analysis of the role of Arabidopsis class I TCP genes AtTCP7, AtTCP8, AtTCP22, and AtTCP23 in leaf development. Front Plant Sci, 2013, 8:e24140 |
| [32] | Guo Z, Fujioka S, Blancaflor E B, Miao S, Gou X, Li J.TCP1 modulates brassinosteroid biosynthesis by regulating the expression of the key biosynthetic gene DWARF4 in Arabidopsis thaliana. Plant Cell, 2010, 22: 1161-1173 |
| [33] | Palatnik J F, Allen E, Wu X, Schommer C, Schwab R, Carrington J C.Control of leaf morphogenesis by microRNAs.Nature, 2003, 425: 257-263 |
| [34] | Chandler V L, Radicella J P, Robbins T P, Chen J, Turks D.Two regulatory genes of the maize anthocyanin pathway are homologous: isolation of B utilizing R genomic sequences.Plant Cell, 1989, 1: 1175-1183 |
| [35] | de Vetten N, Quattrocchio F, Mol J, Koes R. The an11 locus controlling flower pigmentation in petunia encodes a novel WD-repeat protein conserved in yeast, plants, and animals.Genes Dev, 1997, 11: 1422-1434 |
| [36] | Baudry A, Caboche M, Lepiniec L.TT8 controls its own expression in a feedback regulation involving TTG1 and homologous MYB and bHLH factors, allowing a strong and cell-specific accumulation of flavonoids in Arabidopsis thaliana. Plant Mol Biol, 2006, 46: 768-779 |
| [37] | Zhang F, Gonzalez A, Zhao M, Payne C T, Lloyd A.A network of redundant bHLH proteins functions in all TTG1-dependent pathways of Arabidopsis. Development, 2003, 130: 4859-4869 |
| [38] | Liu X F, Yin X R, Allan A C, Wang K L, Shi Y N, Huang Y J.The role of MrbHLH1, and MrMYB1, in regulating anthocyanin biosynthetic genes in tobacco and Chinese bayberry (Myrica rubra) during anthocyanin biosynthesis. Plant Cell Tissue Org, 2013, 115: 285-298 |
| [39] | Chiu L W, Zhou X, Burke S, Wu X, Prior R L, Li L.The purple cauliflower arises from activation of a MYB transcription factor.Plant Physiol, 2010, 154: 1470-1480 |
| [1] | 马小倩, 秦娜, 代书桃, 秦家范, 李小艳, 王淑婷, 刘忠玲, 李君霞. 175份谷子种质在2种环境下的表型变异分析[J]. 作物学报, 2026, 52(6): 1757-1773. |
| [2] | 左同鸿, 张贺翠, 曾静, 朱利泉. 甘蓝自交不亲和相关基因BoPUB3L的克隆与表达分析[J]. 作物学报, 2026, 52(6): 1698-1710. |
| [3] | 杨扬, 常诗惠, 田红丽, 易红梅, 王璐, 任洁, 范亚明, 刘亚维, 王凤格, 赵久然. 不同生态区国审玉米品种的遗传多样性分析[J]. 作物学报, 2026, 52(5): 1352-1364. |
| [4] | 徐建霞, 丁延庆, 曹宁, 程斌, 高旭, 李文贞, 王若若, 王磊, 张立异. 397份高粱种质资源在贵州表型多样性分析及综合评价[J]. 作物学报, 2026, 52(4): 1073-1087. |
| [5] | 王楚锐, 李开祥, 赵志, 肖麓, 唐国永, 赵志刚, 徐亮, 杜德志, 柳海东. 甘蓝型春油菜早花基因BnCRY2功能位点KASP标记的开发及应用[J]. 作物学报, 2026, 52(3): 708-721. |
| [6] | 张超, 郭欢, 李忠玲, 岳淑宁, 赵娜. 基于BSA-seq技术定位玉米籽粒花青素关联基因[J]. 作物学报, 2026, 52(3): 780-789. |
| [7] | 马毅娜, 吴晓明玉, 李藕琪, 王圆, 陈丽, 张盈川, 赵伦, 文静, 傅廷栋, 沈金雄. Bna-miR1040-EIF3A模块调控油菜开花时间的功能研究[J]. 作物学报, 2026, 52(2): 349-362. |
| [8] | 余开航, 周洪斌, 罗亮扎, 王玫郦, 姜瑞梅, 董陈文华, 李仕金, 毛孝强, 陈升位. 大麦亮氨酸富集重复型类受体激酶基因HvLRR-RLK-510的克隆和表达分析[J]. 作物学报, 2026, 52(2): 421-432. |
| [9] | 刘迪, 黎瑞源, 石茂竹, 李洪有, 陈庆富, 石桃雄. 苦荞半矮秆突变体sd3的表型鉴定及转录组分析[J]. 作物学报, 2026, 52(1): 316-328. |
| [10] | 薛晓菲, 戴云静, 李熙林, 丁艳艳, 王翔, 雷长英, 韩焕勇, 贺道华. 陆地棉杜松烯合酶基因GhCDN10的特征及其在棉酚合成中功能分析[J]. 作物学报, 2025, 51(8): 2060-2076. |
| [11] | 许忆葳, 张莹莹, 李瑞, 燕永亮, 刘允军, 孔照胜, 郑军, 王逸茹. 戈壁异常球菌csp2基因提高玉米的抗旱性[J]. 作物学报, 2025, 51(8): 1981-1990. |
| [12] | 王彬, 蒙姜宇, 邱浩良, 贺亚军, 钱伟. 甘蓝型油菜BnaDUF579基因家族的鉴定与表达模式分析[J]. 作物学报, 2025, 51(8): 2100-2110. |
| [13] | 旺姆, 卓嘎, 扎桑, 西若曲宗, 达瓦顿珠, 郭刚刚, 张京, 卓嘎, 伦珠朗杰. 基于6个表型性状的青稞种质遗传多样性分析及综合评价[J]. 作物学报, 2025, 51(6): 1526-1537. |
| [14] | 夏琦, 郭滢, 王坤美, 王思忆, 巨建业, 彭雅雯, 刘忠松, 夏石头. 甘蓝型油菜种子和种皮中水杨酸含量与原花色素积累的关系研究[J]. 作物学报, 2025, 51(5): 1189-1197. |
| [15] | 王晓琳, 刘忠松, 康雷, 杨柳. 甘蓝型油菜角果长度和每角粒数基因定位以及角果皮转录组动态分析[J]. 作物学报, 2025, 51(4): 888-899. |
|
||