欢迎访问作物学报,今天是
作物学报 ›› 2020, Vol. 46 ›› Issue (12): 1831-1838.doi: 10.3724/SP.J.1006.2020.03017
宋欣冉1( ), 胡书婷2(), 张凯2, 崔则瑾2, 李建生2, 杨小红2, 白光红1,*()
Xin-Ran SONG1(), Shu-Ting HU2(), Kai ZHANG2, Ze-Jin CUI2, Jian-Sheng LI2, Xiao-Hong YANG2, Guang-Hong BAI1,*()
摘要:
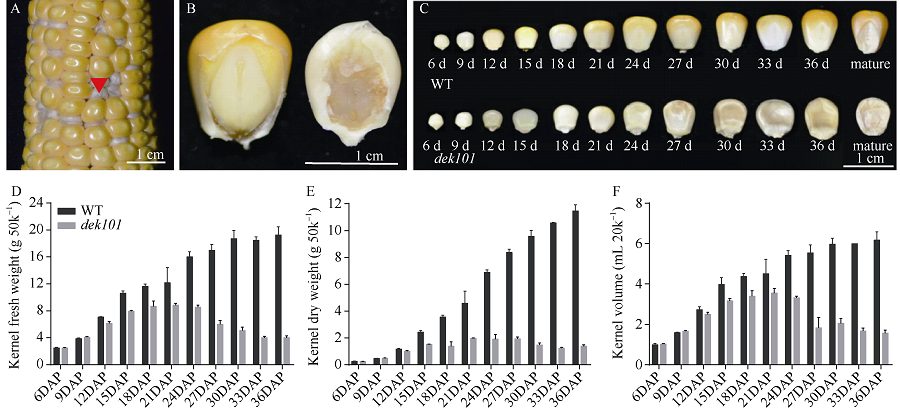
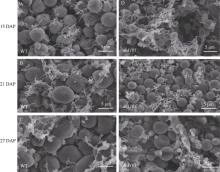
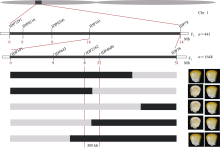
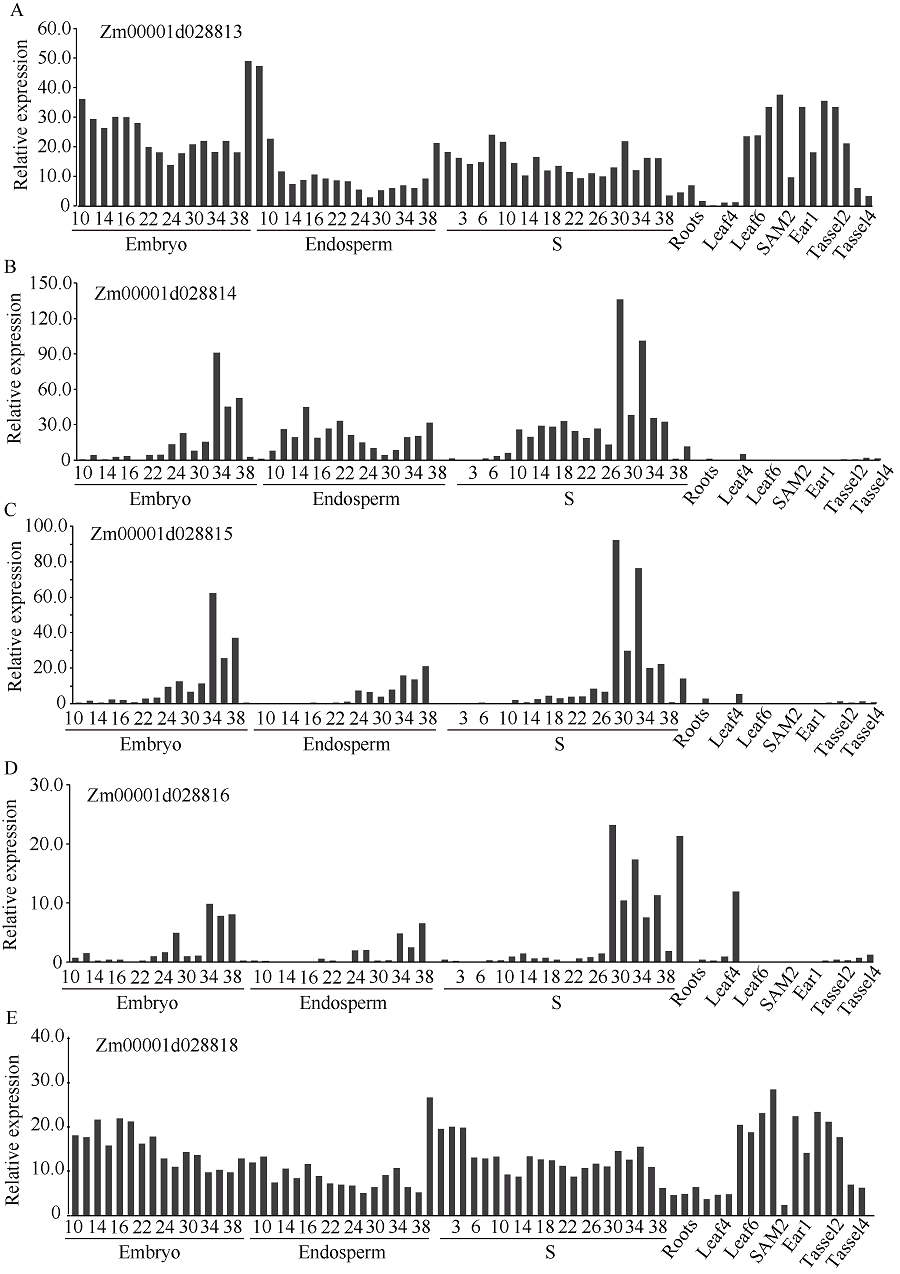
籽粒作为玉米储藏器官, 其发育程度和物质储存直接影响玉米的产量和品质。本研究在玉米双单倍体系选育过程中发现可稳定遗传的籽粒缺陷突变体, 命名为defective kernel 101 (dek101)。该突变体籽粒皱缩, 粒重显著降低, 胚致死, 胚乳发育缺陷, 不能成苗。在授粉后12 d, dek101开始出现明显的发育异常, 授粉后21 d籽粒鲜重、干重、体积不再增加。扫描电镜观察发现, 与野生型相比, dek101淀粉粒显著变小。遗传分析证实该突变性状受隐性单基因控制。利用441个F2单株和1648个F3单株, 将该基因定位在1号染色体的标记IDP2182和IDP4600之间, 物理区间约300 kb, 共有5个预测基因。这些结果为挖掘与玉米籽粒发育有关的功能基因, 解析籽粒发育机制奠定了基础。
| [1] | Rossi V, Hartings H, Thompson R, Mario M . Genetic and molecular approaches for upgrading starch and protein fractions in maize kernels. Maydica, 2001,46:147-158. |
| [2] |
Shannon J C, Pien F M, Cao H, Liu K C . Brittle-1, an adenylate translocator, facilitates transfer of extraplastidial synthesized ADP-Glucose into amyloplasts of maize endosperms. Plant Physiol, 1998,117:1235-1252.
doi: 10.1104/pp.117.4.1235 pmid: 9701580 |
| [3] |
Dickinson D B, Preiss J . Presence of ADP-Glucose pyrophosphorylase in shrunken-2 and brittle-2 mutants of maize endosperm. Plant Physiol, 1969,44:1058-1062.
doi: 10.1104/pp.44.7.1058 pmid: 16657157 |
| [4] |
Zhang X L, Colleoni C, Ratushna V, Colleoni M S, Martha J, Myers A . Molecular characterization demonstrates that the Zea mays gene sugary2 codes for the starch synthase isoform SSIIa. Plant Mol Biol, 2004,54:865-879.
doi: 10.1007/s11103-004-0312-1 |
| [5] | Wang Y J, White P, Pollak L, Jane J L . Characterization of starch structure of 17 maize endosperm mutant genotypes with Oh43 inbred line background. Cereal Chem, 1993,70:171-179. |
| [6] |
Shure M, Wessler S, Fedoroff N . Molecular identification and isolation of the waxy locus in maize. Cell, 1983,35:225-233.
doi: 10.1016/0092-8674(83)90225-8 pmid: 6313224 |
| [7] |
Fu S N, Meeley R, Scanlon M J . Empty pericarp2 encodes a negative regulator of the heat shock response and is required for maize embryogenesis. Plant Cell, 2002,14:3119-3132.
doi: 10.1105/tpc.006726 pmid: 12468731 |
| [8] |
Jose F, Gutierrez M, Mauro D P . Empty pericarp4 encodes a mitochondrion-targeted Pentatricopeptide repeat protein necessary for seed development and plant growth in maize. Plant Cell, 2007,19:196-210.
doi: 10.1105/tpc.105.039594 pmid: 17259266 |
| [9] |
He Y H, Wang J G, Qi W W, Song R T . Maize dek15 encodes the cohesin-loading complex subunit SCC4 and is essential for chromosome segregation and kernel development. Plant Cell, 2019,31:465-485.
doi: 10.1105/tpc.18.00921 pmid: 30705131 |
| [10] |
Garcia N, Li Y B, Dooner H K, Messing J . Maize defective kernel mutant generated by insertion of a Ds element in a gene encoding a highly conserved TTI2 cochaperone. Proc Natl Acad Sci USA, 2017,114:5165-5170.
doi: 10.1073/pnas.1703498114 pmid: 28461460 |
| [11] |
Qi W W, Lu L, Huang S C, Song R T . Maize dek44 encodes mitochondrial ribosomal protein L9 and is required for seed development. Plant Physiol, 2019,180:2106-2119.
doi: 10.1104/pp.19.00546 pmid: 31182559 |
| [12] |
Shen Y, Li C L, McCarty D R, Meeley R, Bao C T . Embryo defective 12 encodes the plastid initiation factor 3 and is essential for embryogenesis in maize. Plant J, 2013,74:792-804.
doi: 10.1111/tpj.12161 |
| [13] |
Li C, Shen Y, Meeley R, McCarty D R, Bao C T . Embryo defective 14 encodes a plastid-targeted cGTPase essential for embryogenesis in maize. Plant J, 2015,84:785-799.
doi: 10.1111/tpj.13045 pmid: 26771182 |
| [14] |
Mertz ET, Bates L S, Nelson O E . Mutant gene that changes protein composition and increases lysine content of maize endosperm. Science, 1964,145:279-280.
doi: 10.1126/science.145.3629.279 pmid: 14171571 |
| [15] |
Ueda T, Waverczak W, Ward K, Sher K, Ketuda M, Schmidt R J, Messing J . Mutations of the 22- and 27-kD zein promoters affect transactivation by the Opaque-2 protein. Plant Cell, 1992,4:701-709.
doi: 10.1105/tpc.4.6.701 pmid: 1392591 |
| [16] | Coleman C E, Larkins B A . The Prolamins of Maize. Seed Proteins. Springer Netherlands, 1999. pp 109-139. |
| [17] | Nelson O E, Mertz E T, Bates L S . Second mutant gene affecting the amino acid pattern of maize. Endosperm Proteins, 1966,150:1469-1470. |
| [18] |
Huang Y C, Wang H H, Huang X, Wang Q, Wang C J, An D, Li J Q, Wang W Q, Wu Y R . Maize VKS1 regulates mitosis and cytokinesis during early endosperm development. Plant Cell, 2019,31:1238-1256.
doi: 10.1105/tpc.18.00966 pmid: 30962394 |
| [19] |
Zheng X X, Li Q, Li C S, An D, Xiao Q, Wang W Q, Wu Y R . Intra-kernel reallocation of proteins in maize depends on VP1-mediated scutellum development and nutrient assimilation. Plant Cell, 2019,31:2613-2635.
doi: 10.1105/tpc.19.00444 pmid: 31530735 |
| [20] |
Chen J, Zeng B, Zhang M, Xie S J, Wang G K, Hauck A, Lai J S . Dynamic transcriptome landscape of maize embryo and endosperm development. Plant Physiol, 2014,166:252-264.
doi: 10.1104/pp.114.240689 |
| [21] |
Chourey P S, Nelson O E . The enzymatic deficiency conditioned by the shrunken-1, mutations in maize. Biochem Genet, 1976,14:1041-1055.
doi: 10.1007/BF00485135 pmid: 1016220 |
| [22] |
Hannah L C, Jr O E N . Characterization of ADP-glucose pyrophosphorylase from shrunken-2, and brittle-2, mutants of maize. Biochemical Genet, 1976,14:547-560.
doi: 10.1007/BF00485834 |
| [23] |
Gao M, Wanat J, Stinard P S, James M G, Myers A M . Characterization of dull1, a maize gene coding for a novel starch synthase. Plant Cell, 1998,10:399-412.
doi: 10.1105/tpc.10.3.399 pmid: 9501113 |
| [24] |
Magnard J L, Heckel T, Massonneau A, Wisniewski J P, Cordelier S, Lassagne H, Perez P, Dumas C, Rogowsky P M . Morphogenesis of maize embryos requires ZmPRPL35-1 encoding a plastid ribosomal protein. Plant Physiol, 2004,134:649-663.
doi: 10.1104/pp.103.030767 pmid: 14730079 |
| [25] |
Qi W, Tian Z, Lu L, Chen X, Chen X, Zhang W, Song R T . Editing of mitochondrial transcripts nad3 and cox2 by dek10 is essential for mitochondrial function and maize plant development. Genetics, 2017,205:1489-1501.
doi: 10.1534/genetics.116.199331 pmid: 28213476 |
| [26] |
Chen X, Feng F, Qi W, Xu L, Yao D, Wang Q, Song R T . Dek35 encodes a PPR protein that affects cis-splicing of mitochondrial nad4 intron 1 and seed development in maize. Mol Plant, 2017,10:427-441.
doi: 10.1016/j.molp.2016.08.008 pmid: 27596292 |
| [27] |
Wang G, Zhong M, Shuai B, Song J, Zhang J, Han L, Ling H, Tang Y, Wang G, Song R T . E+ subgroup PPR protein defective kernel 36 is required for multiple mitochondrial transcripts editing and seed development in maize and Arabidopsis. New Phytol, 2017,214:1563-1578.
doi: 10.1111/nph.14507 pmid: 28277611 |
| [28] |
Dai D, Luan S, Chen X, Wang Q, Feng Y, Zhu C, Qi W, Song R T . Maize dek37 encodes a P-type PPR protein that affects cis-splicing of mitochondrial nad2 intron 1 and seed development. Genetics, 2018,208:1069-1082.
doi: 10.1534/genetics.117.300602 pmid: 29301905 |
| [29] |
Li X, Gu W, Sun S, Chen Z, Chen J, Song W, Zhao H, Lai J . Defective kernel 39 encodes a PPR protein required for seed development in maize. J Integr Plant Biol, 2018,60:45-64.
doi: 10.1111/jipb.12602 |
| [30] |
Ren R C, Lu X, Zhao Y J, Wei Y M, Wang L L, Zhang L, Zhang W T, Zhang C, Zhang X S, Zhao X Y . Pentatricopeptide repeat protein DEK40 is required for mitochondrial function and kernel development in maize. J Exp Bot, 2019,70:6163-6179.
doi: 10.1093/jxb/erz391 pmid: 31598687 |
| [31] |
Zuo Y, Feng F, Qi W W, Song R T . Dek42 encodes an RNA-binding protein that affects alternative pre-mRNA splicing and maize kernel development. J Integr Plant Biol, 2019,61:728-748.
doi: 10.1111/jipb.12798 |
| [32] |
Stein E L, Darren G, Rudolf J, Jennifer A L, Evgueni A, Mark C, Niu X M, Meeley R, Nichols S, Olsen O A . The defective kernel 1 (dek 1) gene required for aleurone cell development in the endosperm of maize grains encodes a membrane protein of the calpain gene superfamily. Proc Natl Acad Sci USA, 2002,99:5460-5465.
doi: 10.1073/pnas.042098799 pmid: 11929961 |
| [33] |
Zhu C, Jin G, Fang P, Zhang Y, Feng X, Tang Y, Qi W W, Song R T . Maize Pentatricopeptide repeat protein DEK41 affects cis-splicing of mitochondrial nad4 intron 3 and is required for normal seed development. J Exp Bot, 2019,70:3795-3808.
doi: 10.1093/jxb/erz193 pmid: 31020318 |
| [34] |
Yi G, Lauter A M, Scott P, Becraft P W . The thick aleurone1 mutant defines a negative regulation of maize aleurone cell fate that functions downstream of defective kernel 1. Plant Physiol, 2011,156:1826-1836.
doi: 10.1104/pp.111.177725 |
| [35] |
Xu C, Min J R . Structure and function of WD40 domain proteins. Protein Cell, 2011,2:202-214.
doi: 10.1007/s13238-011-1018-1 |
| [36] |
Xie Y R, Chen Z Y, Brown R L, Bhatnagar D . Expression and functional characterization of two pathogenesis-related protein 10 genes from Zea mays. J Plant Physiol, 2010,167:121-130.
doi: 10.1016/j.jplph.2009.07.004 pmid: 19682768 |
| [1] | 刘恩波, 陈静, 李红星, 于宁宁, 任佰朝, 赵斌, 刘鹏, 张吉旺. 遮阴改变源-库平衡和调节碳水化合物代谢进而抑制夏玉米幼穗发育[J]. 作物学报, 2026, 52(6): 1891-1901. |
| [2] | 梁进宇, 尹嘉德, 王红丽, 张国平, 侯慧芝, 董博, 马明生. 基于无人机高光谱和机器学习的旱地饲用玉米叶片氮含量估测[J]. 作物学报, 2026, 52(6): 1788-1801. |
| [3] | 孙淑凤, 许振南, 黄嘉鑫, 翁建峰, 李新海. 玉米MAPK家族全基因组鉴定及其对拟轮枝镰孢菌感染的响应[J]. 作物学报, 2026, 52(5): 1291-1308. |
| [4] | 张宁宁, 滕雨菲, 任娜娜, 魏兴卓, 闫书豪, 樊可心, 王永宏, 陈文康, 张兴华, 朱万超, 徐淑兔, 薛吉全. 201份玉米自交系抗旱表型评价及可塑性分析[J]. 作物学报, 2026, 52(5): 1309-1325. |
| [5] | 张鸿蓉, 王菲儿, 李盼, 仇海龙, 朱静, 赵连豪, 南运有, 何蔚, 樊志龙, 胡发龙, 柴强, 殷文. 减量20%灌水与25%有机肥替代化肥提高青贮玉米产量的光合特性[J]. 作物学报, 2026, 52(5): 1487-1500. |
| [6] | 杨欣雨, 崔文涛, 迪力尼格尔·阿力木, 汪凯翔, 吴鹏昊, 任姣姣. 玉米穗上叶片数全基因组关联分析和全基因组选择[J]. 作物学报, 2026, 52(5): 1573-1590. |
| [7] | 韩亚鑫, 何冠华, 张小琼, 张登峰, 李永祥, 刘旭洋, 王天宇, 黎裕, 邹华文, 李春辉. 基于RNA-Seq和BSA-Seq联合分析挖掘玉米侧根密度基因资源[J]. 作物学报, 2026, 52(5): 1341-1352. |
| [8] | 杨扬, 常诗惠, 田红丽, 易红梅, 王璐, 任洁, 范亚明, 刘亚维, 王凤格, 赵久然. 不同生态区国审玉米品种的遗传多样性分析[J]. 作物学报, 2026, 52(5): 1352-1364. |
| [9] | 蔡宏玮, 于爱忠, 姜科强, 王鹏飞, 王玉珑, 霍建喆, 庞小能, 尹波, 尚永盼. 干旱灌区有机肥替代部分化肥促进甜玉米产量提升的关键机制[J]. 作物学报, 2026, 52(4): 1166-1180. |
| [10] | 田红丽, 杨扬, 范亚明, 易红梅, 郭丹丹, 王凤格, 赵久然. 适于玉米品种鉴定的一套三等位变异SNP新型标记组合[J]. 作物学报, 2026, 52(4): 993-1005. |
| [11] | 杨亚莉, 徐明睿, 马越飞, 海艺蕊, 刘凯栋, 刘万茂, 孙颖. 玉米根尖及整根响应缺铁的转录组比较研究[J]. 作物学报, 2026, 52(4): 1006-1021. |
| [12] | 马亮, 马璐, 张舒钰, 章慧敏, 王仁明, 宋旭东, 张振良, 冒宇翔, 陆虎华, 陈国清, 郝德荣, 周广飞. 玉米苞叶数目转录组分析及候选基因鉴定[J]. 作物学报, 2026, 52(3): 790-801. |
| [13] | 孟成, 王哲. 玉米ZmPFK基因家族全基因组鉴定及响应胁迫表达分析[J]. 作物学报, 2026, 52(3): 764-779. |
| [14] | 李新浩, 邢梦柯, 周梓惠, 李思烨, 任昊, 王洪章, 赖华江. 外源褪黑素通过协调光反应与暗反应增强玉米苗期的耐热性[J]. 作物学报, 2026, 52(3): 839-856. |
| [15] | 张超, 郭欢, 李忠玲, 岳淑宁, 赵娜. 基于BSA-seq技术定位玉米籽粒花青素关联基因[J]. 作物学报, 2026, 52(3): 780-789. |
|
||