欢迎访问作物学报,今天是
作物学报 ›› 2024, Vol. 50 ›› Issue (11): 2908-2916.doi: 10.3724/SP.J.1006.2024.42013
• 研究简报 • 上一篇
徐飞( ), 刘杨, 许健成, 余璐璐()
XU Fei(), LIU Yang, XU Jian-Cheng, YU Lu-Lu()
摘要:
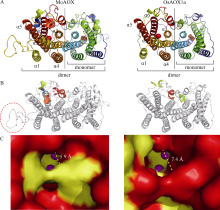
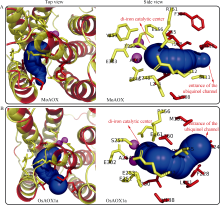
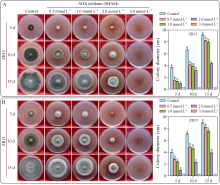
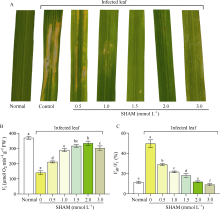
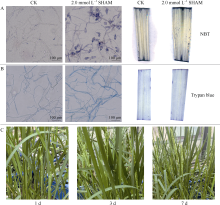
水稻(Oryza sativa L.)是世界主要粮食作物之一。中国作为世界上最大的稻米生产国, 每年因稻瘟菌(Magnaporthe oryzae)引起的稻瘟病受到广泛关注。稻瘟病在水稻整个生育期中均可发生, 从而引起水稻大幅度减产, 甚至颗粒无收。值得注意的是, 交替氧化酶(alternative oxidase, AOX)广泛存在于植物和真菌中, 是线粒体呼吸电子传递链中的末端氧化酶, 被证实参与了胁迫条件下植物的生长发育调节以及真菌胁迫响应等。本文比较分析了水稻AOX和稻瘟菌AOX蛋白结构差异, 并利用AOX抑制剂开展稻瘟菌防治试验。结果表明,水稻AOX和稻瘟菌AOX蛋白的双铁催化活性中心的氨基酸残基相对保守, 但其在泛醌通道大小、氨基酸组成以及形成的疏水口袋等方面有较大差异。通过AOX抑制剂处理可明显减缓稻瘟菌菌丝的生长, 并减轻水稻叶片稻瘟菌病害症状。本研究表明, AOX可作为有效靶标用于抑制稻瘟菌, 在水稻稻瘟菌病害防治方面具有潜在应用价值。
| [1] |
韩艺娟, 鲁国东. 水稻与稻瘟病菌相互作用研究进展. 生物技术通报, 2018, 34(2): 25-37.
doi: 10.13560/j.cnki.biotech.bull.1985.2017-0623 |
| [2] | Han Y J, Lu G D. Recent understanding on the interactions between rice and Magnaporthe oryzae. Biotechnol Bull 2018, 34(2): 25-37 (in Chinese with English abstract). |
| [3] |
Yin J, Zou L, Zhu X, Cao Y, He M, Chen X. Fighting the enemy: How rice survives the blast pathogen’s attack. Crop J, 2021, 9: 543-552.
doi: 10.1016/j.cj.2021.03.009 |
| [4] | Jo L, Pelletier J M, Hsu S W, Baden R, Goldberg R B, Harada J J. Combinatorial interactions of the LEC1 transcription factor specify diverse developmental programs during soybean seed development. Proc Natl Acad Sci USA, 2020, 117: 1223-1232. |
| [5] | Kumar S, Kashyap P L, Mahapatra S, Jasrotia P, Singh G P. New and emerging technologies for detecting Magnaporthe oryzae causing blast disease in crop plants. Crop Prot, 2021, 143: 105473. |
| [6] | Galhano R, Talbot N J. The biology of blast: understanding how Magnaporthe oryzae invades rice plants. Fungal Biol Rev, 2011, 25: 61-67. |
| [7] | Xu F, Copsey A C, Young L, Barsottini M R O, Albury M S, Moore A L. Comparison of the kinetic parameters of alternative oxidases from Trypanosoma brucei and Arabidopsis thaliana: a tale of two cavities. Front Plant Sci, 2021, 12: 744218. |
| [8] |
DelSaz N F, Ribas-Carbo M, McDonald A E, Lambers H, Fernie A R, Florez-Sarasa I. An in vivo perspective of the role(s) of the alternative oxidase pathway. Trends Plant Sci, 2018, 23: 206-219.
doi: S1360-1385(17)30259-5 pmid: 29269217 |
| [9] | Xu F, Peng Y, He Z Q, Yu L L. The role of cyanoalanine synthase and alternative oxidase in promoting salt stress tolerance in Arabidopsis thaliana. BMC Plant Biol 2023, 23: 163. |
| [10] |
Xu F, Yuan S, Zhang D W, Lv X, Lin H H. The role of alternative oxidase in tomato fruit ripening and its regulatory interaction with ethylene. J Exp Bot, 2012, 63: 5705-5716.
doi: 10.1093/jxb/ers226 pmid: 22915749 |
| [11] |
Selinski J, Scheibe R, Day D A, Whelan J. Alternative oxidase is positive for plant performance. Trends Plant Sci, 2018, 23: 588-597.
doi: S1360-1385(18)30080-3 pmid: 29665989 |
| [12] | Moore A L, Albury M S, Crichton P G, Affourtit C. Function of the alternative oxidase: is it still a scavenger. Trends Plant Sci, 2002, 7: 478-481. |
| [13] | Li G B, He J X, Wu J L, Wang H, Zhang X, Liu J, Hu X H, Zhu Y, Shen S, Bai Y F, Yao Z L, Liu X X, Zhao J H, Li D Q, Li Y, Huang F, Huang Y Y, Zhao Z X, Zhang J W, Zhou S X, Ji Y P, Pu M, Qin P, Li S G, Chen X W, Wang J, He M, Li W T, Wu X J, Xu Z J, Wang W M, Fan J. Overproduction of OsRACK1A, an effector-targeted scaffold protein promoting OsRBOHB- mediated ROS production, confers rice floral resistance to false smut disease without yield penalty. Mol Plant, 2022, 15: 1790-1806. |
| [14] |
Li Y, Cao X L, Zhu Y, Yang X M, Zhang K N, Xiao Z Y, Wang H, Zhao J H, Zhang L L, Li G B. Osa-miR398b boosts H2O2 production and rice blast disease-resistance via multiple superoxide dismutases. New Phytol, 2019, 222: 1507-1522.
doi: 10.1111/nph.15678 pmid: 30632163 |
| [15] |
Hu J, Liu M, Zhang A, Dai Y, Chen W, Chen F, Wang W, Shen D, Telebanco-Yanoria M J, Ren B. Co-evolved plant and blast fungus ascorbate oxidases orchestrate the redox state of host apoplast to modulate rice immunity. Mol Plant, 2022, 15: 1347-1366.
doi: 10.1016/j.molp.2022.07.001 pmid: 35799449 |
| [16] | Kido Y, Shiba T, Inaoka D K, Sakamoto K, Nara T, Aoki T, Honma T, Tanaka A, Inoue M, Matsuoka S. Crystallization and preliminary crystallographic analysis of cyanide-insensitive alternative oxidase from Trypanosoma brucei brucei. Acta Crystallogr Sect F Struct Biol Cryst Commun 2010, 66: 275-278. |
| [17] | May B, Young L, Moore A L. Structural insights into the alternative oxidases: are all oxidases made equal. Biochem Soc Trans, 2017, 45: 731-740. |
| [18] |
Kawano Y. Fine-tuning ROS homeostasis by ROD1 is a battleground between rice and Magnaporthe oryzae. Mol Plant 2021, 14: 1979-1981.
doi: 10.1016/j.molp.2021.11.005 pmid: 34785317 |
| [19] | Liu X, Zhang Z. A double-edged sword: reactive oxygen species (ROS) during the rice blast fungus and host interaction. FEBS J, 2022, 289: 5505-5515. |
| [20] | Liu Y, Yu L L, Peng Y, Geng X X, Xu F. Alternative oxidase inhibition impairs tobacco root development and root hair formation. Front Plant Sci, 2021, 12: 664792. |
| [21] | Manbir S P, Kumari A, Gupta K J. Alternative oxidase plays a role in minimizing ROS and RNS produced under salinity stress in Arabidopsis thaliana. Physiol Plant 2022, 174: e13649. |
| [1] | 胡赵, 钱润, 谢丰璞, 应素平. 水稻SPX基因家族鉴定及响应磷处理的表达分析[J]. 作物学报, 2026, 52(6): 1902-1912. |
| [2] | 邹仪妹, 徐敏, 汪海洋, 姚辉, 王加峰, 刘浩, 任代胜. 两系不育系水稻幼苗根系响应盐胁迫的转录因子调控网络鉴定[J]. 作物学报, 2026, 52(6): 1728-1742. |
| [3] | 闫安, 蒋昆炜, 王蓉圆, 田林, 张璐, 王韵, 徐建龙. 水稻剑叶小维管束数基因SVN7的鉴定与克隆[J]. 作物学报, 2026, 52(5): 1364-1372. |
| [4] | 陈伟, 卫万娟, 赵其兵, 常东伟, 余凌波, 翟鹏飞, 冯志明, 陈宗祥, 任仰涛, 杨鹏, 刘海浪, 李珍富, 杨永乐, 金彦刚, 左示敏. 利用CRISPR/Cas9编辑Hd6基因创制优质早熟水稻新种质[J]. 作物学报, 2026, 52(4): 1046-1056. |
| [5] | 石少阶, 刘凯, 陈姿夷, 王卉颖, 李三和, 周雷, 游艾青. 水稻矮化多分蘖基因DMT1的克隆与功能分析[J]. 作物学报, 2026, 52(4): 1022-1034. |
| [6] | 覃奕琰, 付瑶, 苏畅, 李娜, 徐静茹, 程笑然, 张琪, 赵明辉. OsST41调控水稻苗期耐盐性的功能分析[J]. 作物学报, 2026, 52(3): 802-812. |
| [7] | 叶凡, 李帅, 李思宇, 陈云, 窦超银, 刘立军. 不同节水灌溉方式对东北稻区水稻产量和群体质量的影响[J]. 作物学报, 2026, 52(3): 895-907. |
| [8] | 王婵, 吴莹莹, 李文奇, 李霞, 王芳权, 周彤, 杨杰. 基于HRM技术开发水稻抗条纹叶枯病基因STV11功能标记[J]. 作物学报, 2025, 51(9): 2547-2556. |
| [9] | 陈惠莹, 何嘉欣, 朱斌, 黄士轩, 周星佑, 伍君权, 杨美艳. 水稻黄单胞菌噬菌体vB_XaS_HDB2的全基因组分析和生物学特性研究[J]. 作物学报, 2025, 51(8): 2087-2099. |
| [10] | 杨海洋, 吴林宣, 李博纹, 石翰峰, 袁禧龙, 刘金朝, 蔡海荣, 陈诗怡, 郭涛, 王慧. 基于QTL定位发现的OsWRI3调控水稻种子的落粒性[J]. 作物学报, 2025, 51(7): 1712-1724. |
| [11] | 雷松翰, 范骏扬, 车艳奕, 代永东, 郑雨萌, 田维江, 桑贤春, 王晓雯. 水稻内卷叶突变体acl3的鉴定及调控基因的功能分析[J]. 作物学报, 2025, 51(6): 1467-1479. |
| [12] | 李福媛, 杨奕, 马继琼, 许明辉, 林良斌, 孙一丁. 水稻OsPUB4基因克隆、激素诱导表达分析与互作蛋白筛选[J]. 作物学报, 2025, 51(6): 1690-1700. |
| [13] | 王梦宁, 谢可冉, 高逖, 王飞, 任孝俭, 熊栋梁, 黄见良, 彭少兵, 崔克辉. 水稻幼穗分化期至抽穗期高温对籽粒形态和充实的影响及其与粒重的关系[J]. 作物学报, 2025, 51(5): 1347-1362. |
| [14] | 盛倩男, 方娅婷, 赵剑, 杜思垚, 胡行珍, 余秋华, 朱俊, 任涛, 鲁剑巍. 不同养分管理措施对稻田和旱地油菜产量的影响及其对冻害的响应[J]. 作物学报, 2025, 51(5): 1286-1298. |
| [15] | 翁文安, 邢志鹏, 胡群, 魏海燕, 廖萍, 朱海滨, 瞿济伟, 李秀丽, 刘桂云, 高辉, 张洪程. 无人化旱直播水稻产量形成特征及其能量与经济效益研究[J]. 作物学报, 2025, 51(5): 1363-1377. |
|
||