欢迎访问作物学报,今天是
作物学报 ›› 2020, Vol. 46 ›› Issue (8): 1146-1156.doi: 10.3724/SP.J.1006.2020.94198
冯韬1,2,谭晖1,2,官梅2,官春云2,*( )
FENG Tao1,2,TAN Hui1,2,GUAN Mei2,GUAN Chun-Yun2,*()
摘要:
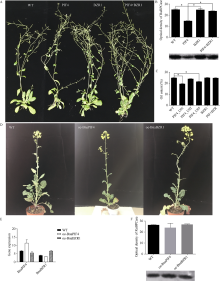
甘蓝型油菜品系XY881和XY883是湘油15辐照诱变后连续自交筛选的2个种子含油量、光合效率和弱光敏感性等有明显差别的子代品系。分别从XY881和XY883中克隆了芸薹素唑抗性因子1 (brassinazole-resistant 1, BnaBZR1) 和光敏色素互作因子4 (phytochrome interacting factor 4, BnaPIF4)基因并进行了序列结构、表达和功能分析。结果表明, XY883的BnaBZR1和BnaPIF4基因存在结构变异, 引起表达和调控模式的差异。XY883中BnaBZR1的启动子具有124 bp的富含A/T的插入序列, 且XY883具有比XY881高的BnaBZR1表达, 并且在弱光和2,4-表油菜素内酯(2,4-BL)诱导下具有较少的表达变化。XY883中BnaPIF4的5'-UTR区域存在可变剪接, 形成长度分别为424 bp (U01)、239 bp (U02)和332 bp (U03)的3种5'-UTR, 在弱光和2,4-BL诱导下, XY883中3种可变剪接的BnaPIF4转录产物的变化不一致。将BnaPIF4的3个5'-UTR与CDS分别组合转化拟南芥后其表达在转录水平无明显差异, 但蛋白翻译存在明显差异, 表明BnaPIF4的5'-UTR变异影响其翻译过程。转BnaPIF4基因拟南芥出现株高增加、叶片狭长且光合作用下降的表型, 共转化BnaBZR1能减弱BnaPIF4造成的光合作用下降; 转BnaPIF4和BnaBZR1基因对油菜的影响与拟南芥相似, 但表型不如拟南芥明显, 表明BnaPIF4是油菜光合作用的负调控因子, 而BnaBZR1可对BnaPIF4的光合负调控产生拮抗; 这与XY881和XY883中两基因表达调控模式及其光合表型相吻合。
| [1] |
Oh E, Zhu J Y, Wang Z Y. Interaction between BZR1 and PIF4 integrates brassinosteroid and environmental responses. Nat Cell Biol, 2012,14:802-809.
doi: 10.1038/ncb2545 pmid: 22820378 |
| [2] |
Bai M Y, Shang J X, Oh E, Fan M, Bai Y, Zentella R, Sun T P, Wang Z Y. Brassinosteroid, gibberellin and phytochrome impinge on a common transcription module in Arabidopsis. Nat Cell Biol, 2012,14:810-817.
doi: 10.1038/ncb2546 pmid: 22820377 |
| [3] |
Gudesblat G E, Russinova E. Plants grow on brassinosteroids. Curr Opin Plant Biol, 2011,14:530-537.
pmid: 21802346 |
| [4] | Ryu H, Hwang I. Brassinosteroids in plant developmental signaling networks. J Plant Biol, 2013,56:267-273. |
| [5] | Wang W, Bai M Y, Wang Z Y. The brassinosteroid signaling network—a paradigm of signal integration. Curr Opin Plant Biol, 2014,21:147-153. |
| [6] | USDA FAS (Foreign Agricultural Service), 2016. Oilseeds: World Markets and Trade. https://www.fas.usda.gov/data/oilseeds-world-markets-and-trade. |
| [7] |
Chalhoub B, Denoeud F, Liu S, Parkin I A, Tang H, Wang X, Corréa M. Early allopolyploid evolution in the post-Neolithic Brassica napus oilseed genome. Science, 2014,345:950-953.
doi: 10.1126/science.1253435 pmid: 25146293 |
| [8] |
Mølmann J A, Hagen S F, Bengtsson G B, Johansen T J. Influence of high latitude light conditions on sensory quality and contents of health and sensory-related compounds in swede roots (Brassica napus L. ssp. rapifera Metzg.). J Sci Food Agric, 2018,98:1117-1123.
doi: 10.1002/jsfa.8562 pmid: 28732144 |
| [9] | 冯韬, 官春云. 甘蓝型油菜光敏色素互作因子4 (BnaPIF4)基因克隆和功能分析. 作物学报, 2019,45:204-213. |
| Feng T, Guan C Y. Cloning and characterization of phytochrome interacting factor 4 (BnaPIF4) gene from Brassica napus L. Acta Agron Sin, 2019,45:204-213 (in Chinese with English abstract). | |
| [10] |
Wei F, Gao G Z, Wang X F, Dong X Y, Li P P, Hua W, Wang X, Wu X M, Chen H. Quantitative determination of oil content in small quantity of oilseed rape by ultrasound-assisted extraction combined with gas chromatography. Ultrason Sonochem, 2008,15:938-942.
pmid: 18504157 |
| [11] | 冯韬, 谭晖, 徐江林, 官春云. 油菜素内酯在不同生育期对两品系甘蓝型油菜的生长调控. 中国油料作物学报, 2019,41:904-913. |
| Feng T, Tan H, Xu J L, Guan C Y. Epibrassinolide regulation on oilseed rape (Brassica napus L.) in different period. Chin J Oil Crop Sci, 2019,41:904-913 (in Chinese with English abstract). | |
| [12] |
Wang Z Y, Nakano T, Gendron J, He J X, Chen M, Vafeados D, Yang Y L, Fujioka S, Yoshida S, Asami T, Chory J. Nuclear-localized BZR1 m llklediates brassinosteroid-induced growth and feedback suppression of brassinosteroid biosynthesis. Dev Cell, 2002,2:505-513.
doi: 10.1016/s1534-5807(02)00153-3 pmid: 11970900 |
| [13] |
Casson S A, Franklin K A, Gray J E, Grierson C S, Whitelam G C, Hetherington A M. Phytochrome B and PIF4 regulate stomatal development in response to light quantity. Curr Biol, 2009,19:229-234.
doi: 10.1016/j.cub.2008.12.046 pmid: 19185498 |
| [14] |
Kumar S V, Lucyshyn D, Jaeger K E, Alós E, Alvey E, Harberd N P, Wigge P A. Transcription factor PIF4 controls the thermosensory activation of flowering. Nature, 2012,484:242-245.
doi: 10.1038/nature10928 pmid: 22437497 |
| [15] |
Lucas M D, Davière J M, Mariana R F, Pontin M, Manuel J I P, Lorrain S, Fankhauser C, Blázquez M A, Titarenko E, Prat S. A molecular framework for light and gibberellin control of cell elongation. Nature, 2008,451:480-484.
doi: 10.1038/nature06520 pmid: 18216857 |
| [16] |
Stella B G, Miguel D L, Cristina M, Ana E R, Davière J M, Prat S. BR-dependent phosphorylation modulates PIF4 transcriptional activity and shapes diurnal hypocotyl growth. Genes Dev, 2014,28:1681-1694.
doi: 10.1101/gad.243675.114 pmid: 25085420 |
| [17] |
Franklin K A, Lee S H, Patel D, Kumar S V, Spartz A K, Gu C, Ye S Q, Yu P, Breen G, Cohen J D, Wigge P A, Gray W M. PHYTOCHROME-NTERACTING FACTOR 4 (PIF4) regulates auxin biosynthesis at high temperature. Proc Natl Acad Sci USA, 2011,108:20231-20235.
doi: 10.1073/pnas.1110682108 pmid: 22123947 |
| [18] | 冯韬, 官春云. 甘蓝型油菜芸薹素唑耐受因子(BnaBZR1/ BnaBES1)全长CDS克隆与生物信息学分析. 作物学报, 2018,44:1793-1801. |
| Feng T, Guan C Y. Cloning and characterization of brassinazole-resistant (BnaBZR1 and BnaBES1) CDS from Brassica napus L. Acta Agron Sin, 2018,44:1793-1801 (in Chinese with English abstract). |
| [1] | 马毅娜, 吴晓明玉, 李藕琪, 王圆, 陈丽, 张盈川, 赵伦, 文静, 傅廷栋, 沈金雄. Bna-miR1040-EIF3A模块调控油菜开花时间的功能研究[J]. 作物学报, 2026, 52(2): 349-362. |
| [2] | 王彬, 蒙姜宇, 邱浩良, 贺亚军, 钱伟. 甘蓝型油菜BnaDUF579基因家族的鉴定与表达模式分析[J]. 作物学报, 2025, 51(8): 2100-2110. |
| [3] | 夏琦, 郭滢, 王坤美, 王思忆, 巨建业, 彭雅雯, 刘忠松, 夏石头. 甘蓝型油菜种子和种皮中水杨酸含量与原花色素积累的关系研究[J]. 作物学报, 2025, 51(5): 1189-1197. |
| [4] | 王晓琳, 刘忠松, 康雷, 杨柳. 甘蓝型油菜角果长度和每角粒数基因定位以及角果皮转录组动态分析[J]. 作物学报, 2025, 51(4): 888-899. |
| [5] | 张琴, 戴成, 马朝芝. 生长素响应报告基因转化甘蓝型油菜及各组织GUS动态信号分析[J]. 作物学报, 2025, 51(3): 667-675. |
| [6] | 孙程明, 周晓婴, 陈锋, 张维, 王晓东, 彭琦, 郭月, 高建芹, 胡茂龙, 付三雄, 张洁夫. 长链非编码RNA (lncRNA)在甘蓝型油菜分枝角度调控中的功能分析与预测[J]. 作物学报, 2025, 51(3): 559-567. |
| [7] | 黄绒, 周渠晨, 陈楚铭, 罗倩, 易东, 杜常欢, 黄祥宇, 盛锋, 杜雪竹. 过表达BnNRT2.3-like对油菜氮素吸收利用及产量的影响[J]. 作物学报, 2025, 51(12): 3184-3197. |
| [8] | 巨建业, 杨柳, 陈浩, 康雷, 夏石头, 刘忠松. 单细胞核转录组分析揭示油菜种皮分化过程和种子颜色差异原因[J]. 作物学报, 2025, 51(11): 2860-2874. |
| [9] | 张雯, 李玉, 王创, 石磊, 丁广大. 甘蓝型油菜磷转运蛋白BnaPT48的功能研究[J]. 作物学报, 2025, 51(11): 2983-2995. |
| [10] | 胡志康, 舒雨, 王会, 杨莹莹, 廖俊宇, 刘佳, 成洪涛, 郭晨, 张园园, 刘胜毅, 胡琼, 梅德圣, 李超. 甘蓝型油菜苗期耐碱性种质综合鉴定与评价[J]. 作物学报, 2025, 51(10): 2681-2692. |
| [11] | 王晨, 贺丹, 姚敏, 邱萍, 何昕, 熊兴华, 康雷, 刘忠松, 钱论文. 基于转录组分析鉴定甘蓝型油菜开花候选基因以及BnaCOR27功能验证[J]. 作物学报, 2025, 51(10): 2693-2704. |
| [12] | 徐林珊, 郜耿东, 王宇, 王家星, 杨吉招, 武亚瑞, 张宵寒, 常影, 李真, 谢雄泽, 龚德平, 王晶, 葛贤宏. 甘蓝型油菜漆酶基因家族成员表达模式及与茎秆抗折力的关联分析[J]. 作物学报, 2025, 51(1): 134-148. |
| [13] | 李嘉欣, 黄莹, 吴潞梅, 赵伦, 易斌, 马朝芝, 涂金星, 沈金雄, 傅廷栋, 文静. 甘蓝型油菜BnaSLY1基因进化分析及功能研究[J]. 作物学报, 2025, 51(1): 44-57. |
| [14] | 钟元, 朱天宇, 戴成, 马朝芝. 耐亚磷酸盐除草剂转基因油菜的创建和抗性评价[J]. 作物学报, 2024, 50(5): 1158-1171. |
| [15] | 曹松, 姚敏, 任睿, 贾元, 向星汝, 李文, 何昕, 刘忠松, 官春云, 钱论文, 熊兴华. 转录组结合区域关联分析挖掘油菜含油量积累的候选基因[J]. 作物学报, 2024, 50(5): 1136-1146. |
|
||