欢迎访问作物学报,今天是
作物学报 ›› 2023, Vol. 49 ›› Issue (8): 2077-2087.doi: 10.3724/SP.J.1006.2023.23062
所属专题: 玉米:遗传育种·种质资源·分子遗传学
王兴荣1( ), 张彦军1, 涂奇奇2, 龚佃明2,*(), 邱法展2,*()
WANG Xing-Rong1(), ZHANG Yan-Jun1, TU Qi-Qi2, GONG Dian-Ming2,*(), QIU Fa-Zhan2,*()
摘要:
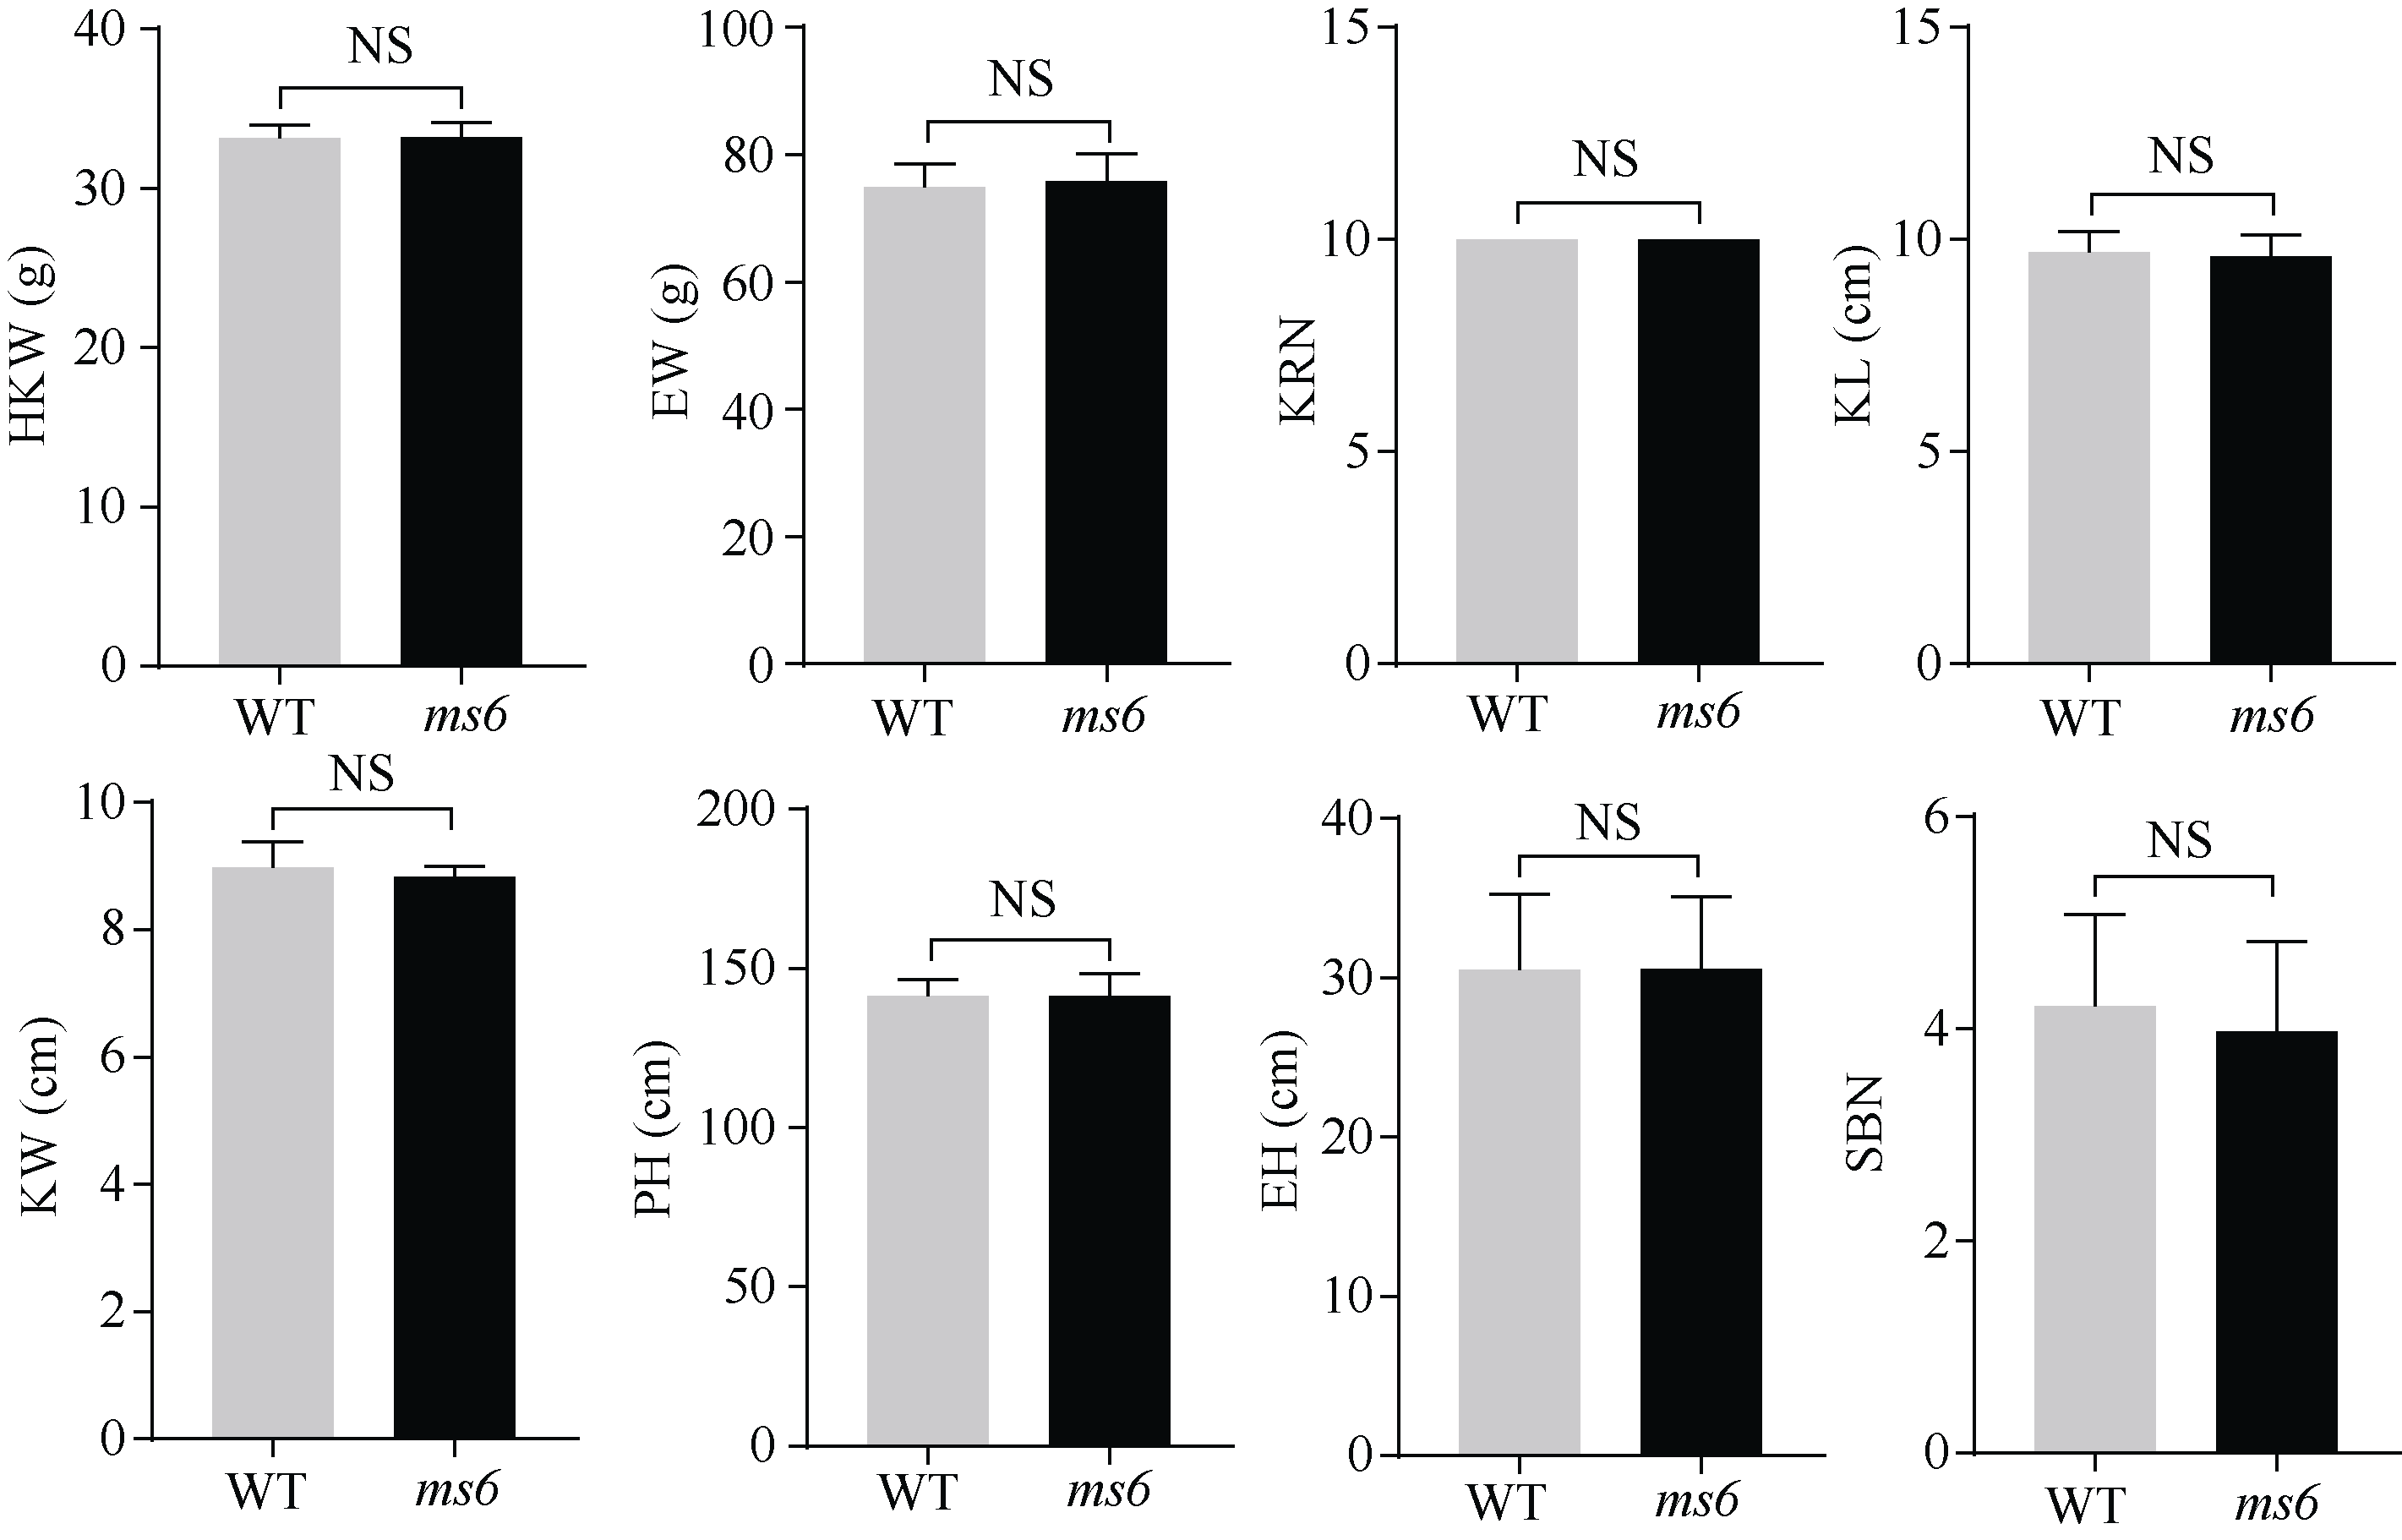
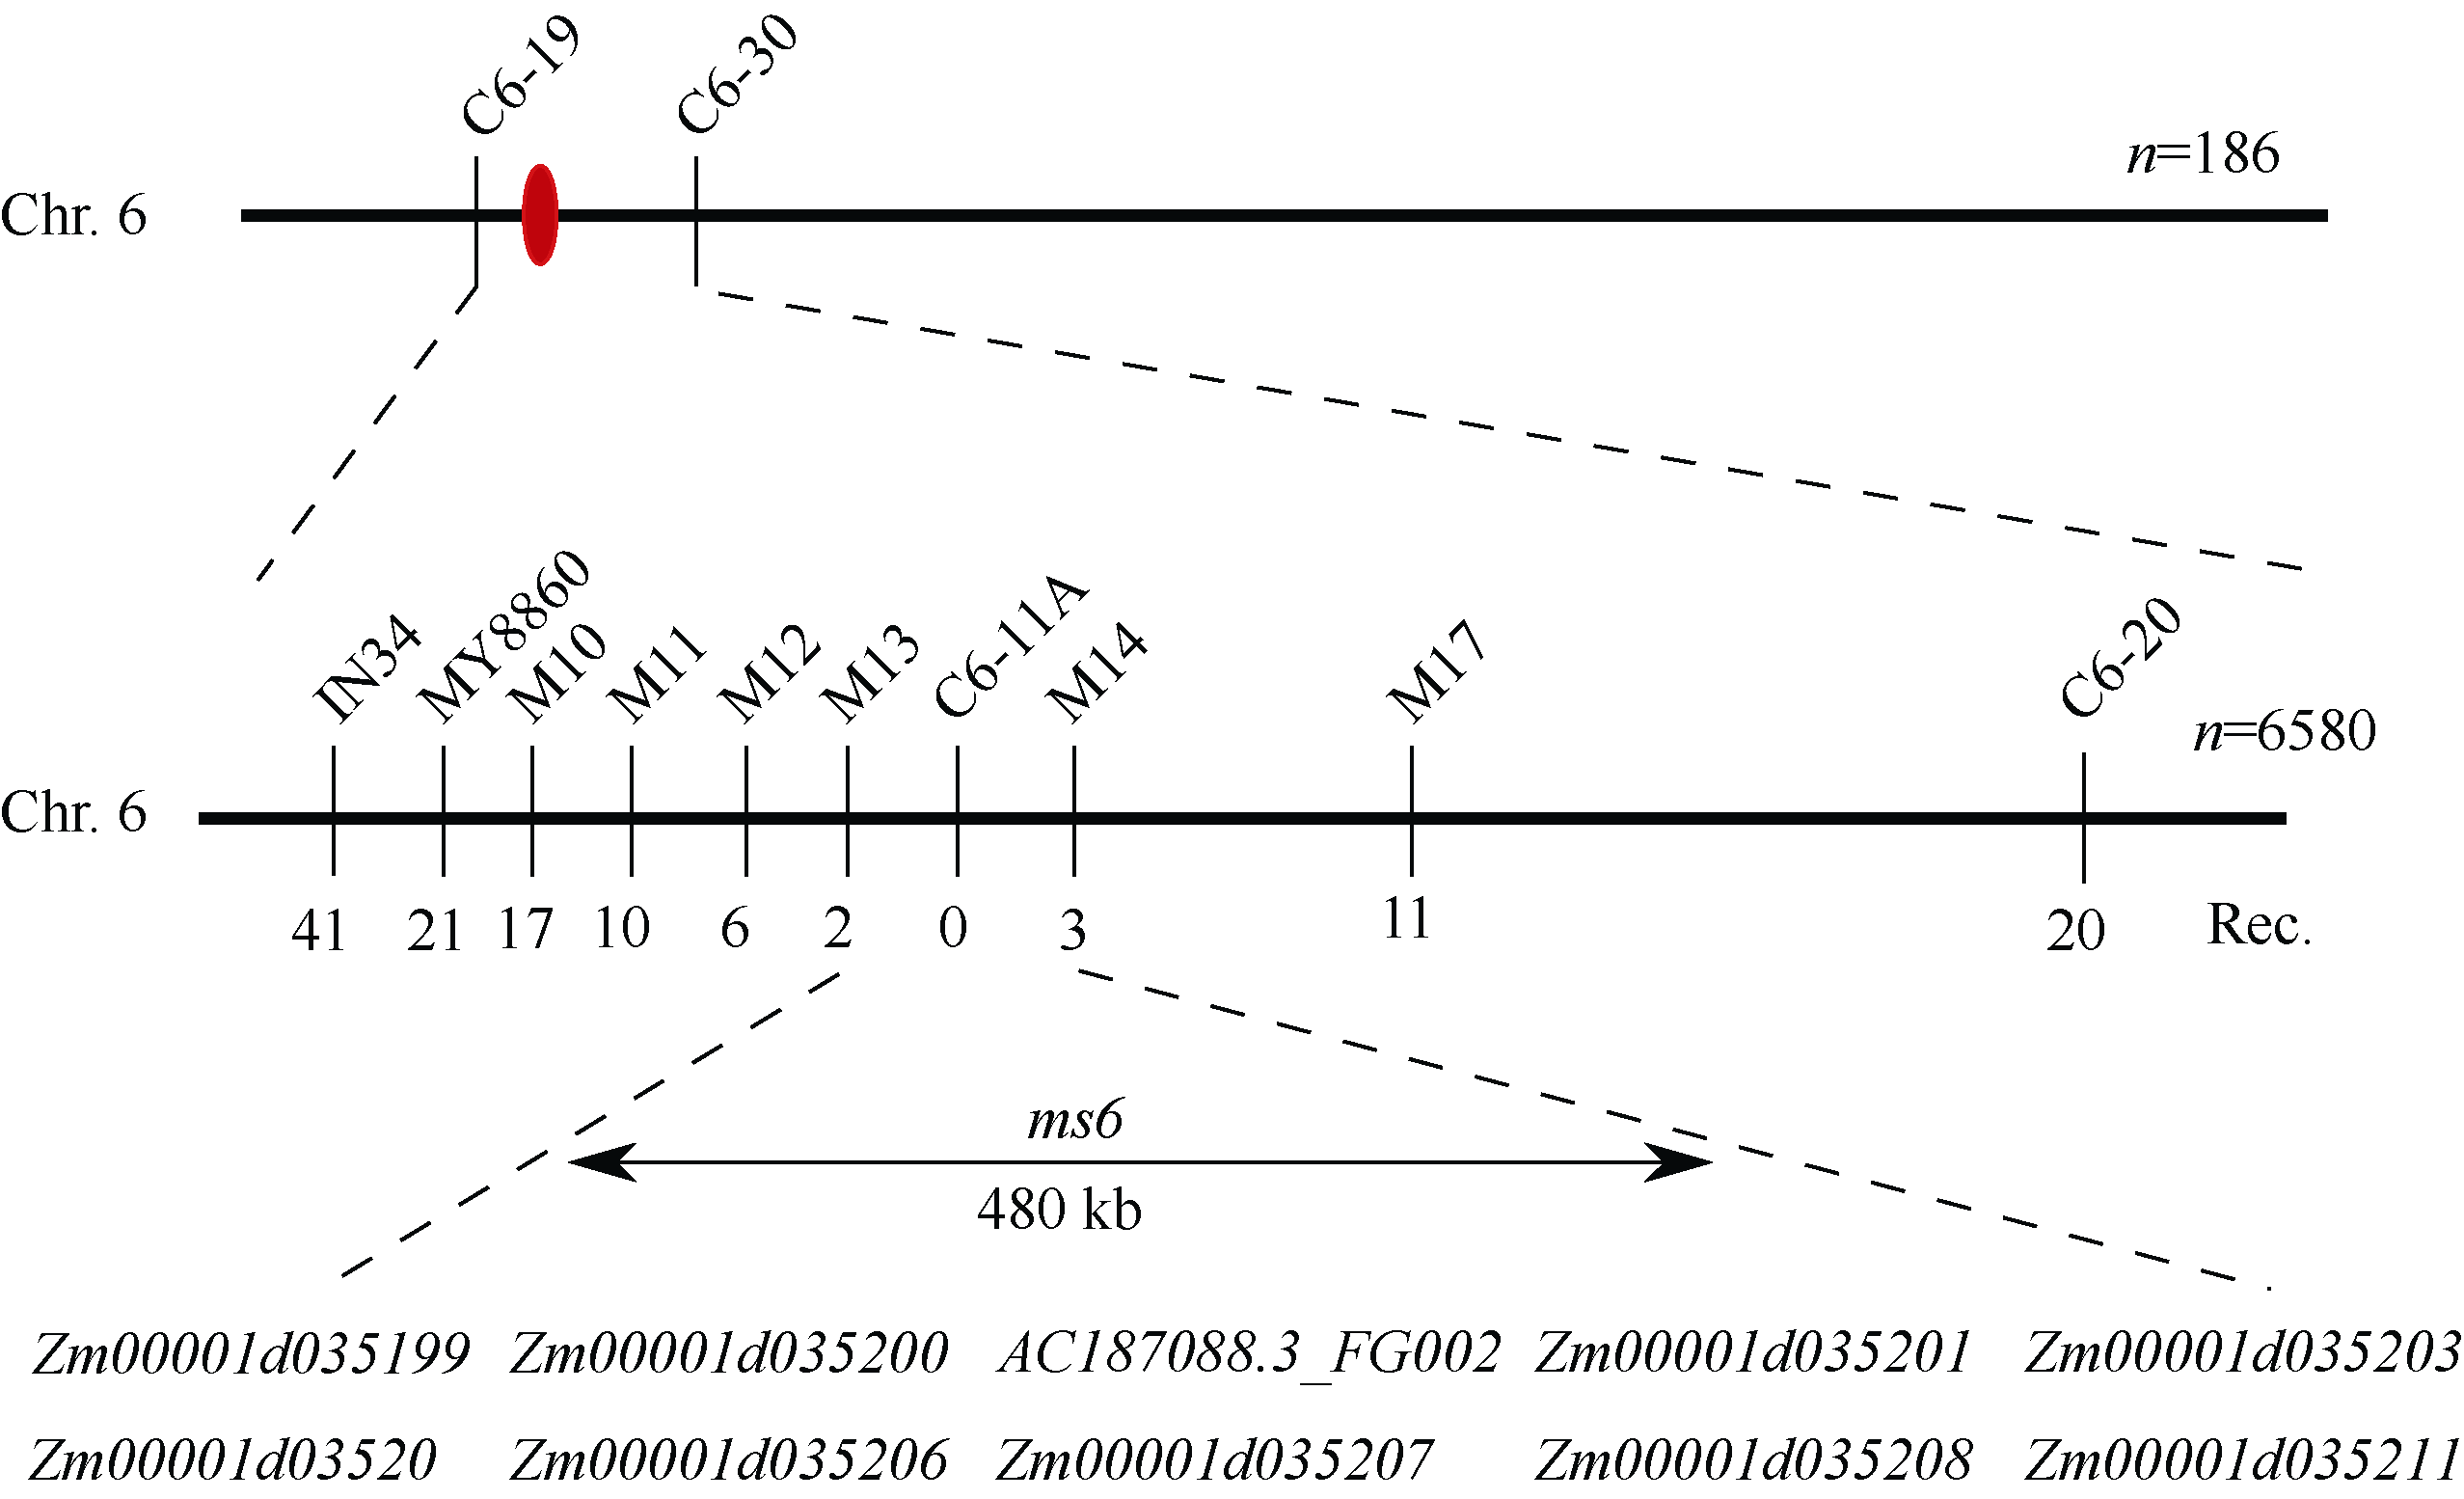
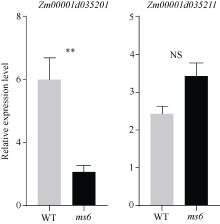
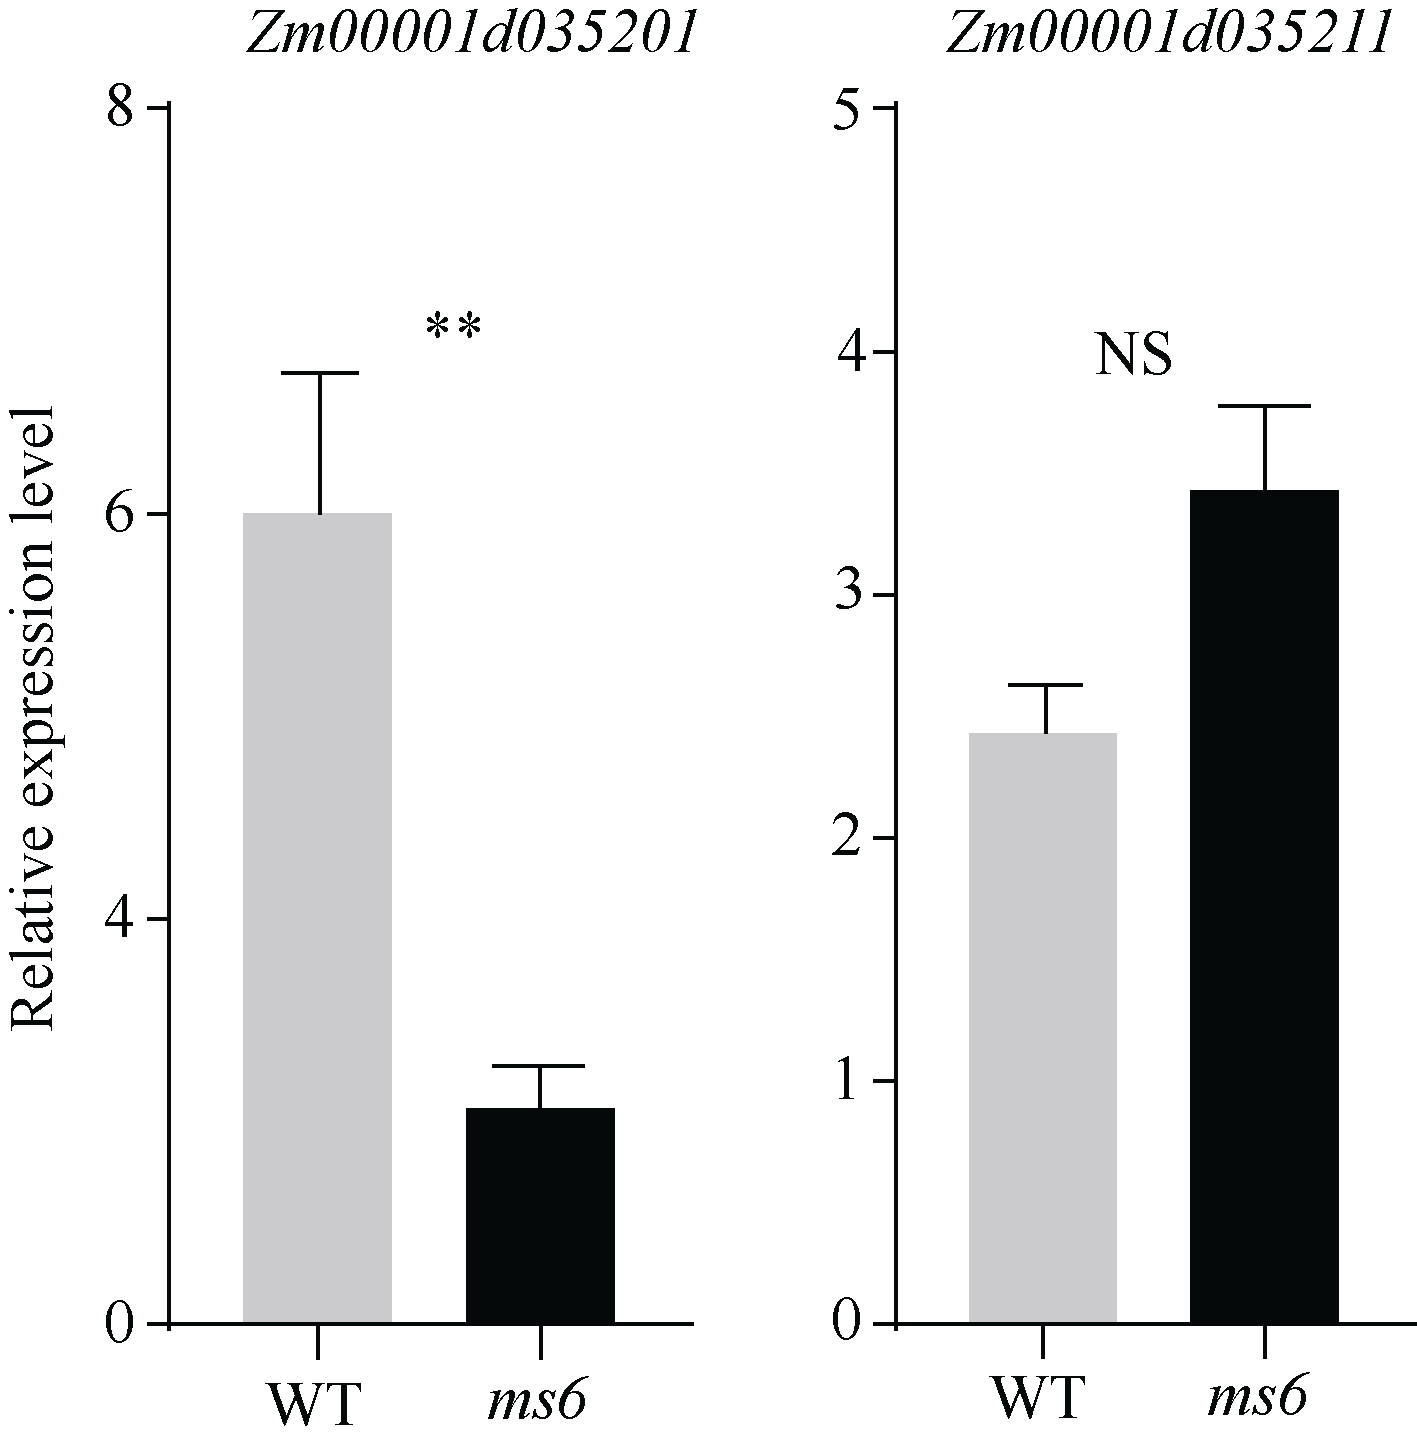
玉米雄性不育基因的定位、克隆和功能机理研究, 不仅能够加深我们对玉米雄花生长发育的分子调控机理的认识, 而且能够有效推动雄性不育技术体系的发展及在玉米育种和种子生产中的运用。本研究以玉米自交系Mo17为野生型背景材料, 经EMS诱变获得了一个玉米雄性不育突变体, 命名为ms6 (male sterile 6)。表型鉴定结果表明, ms6突变体植株能够正常抽雄, 但雄花颖壳不能正常开裂和散粉, 花粉粒干瘪, 表现为无花粉型不育。同时, ms6与Mo17野生型(wild type, WT)在株型、穗部性状以及籽粒粒形等相关性状上无显著差异, 说明该基因突变后, 仅影响植株的育性, 而不影响其他农艺性状。细胞学观察显示, ms6不育突变体的小孢子发育晚期出现异常, 表现为绒毡层细胞提前降解, 小孢子不能进行有丝分裂并逐渐裂解。扫描电镜观察表明, ms6花药外壁皱缩, 内壁无完整的花粉粒, 无乌氏小体的存在。遗传学分析表明, ms6突变性状受1对隐性核基因控制。以ms6 × B73 F2遗传定位群体, 利用全基因组约200对多态性SSR分子标记, 结合表型与基因型连锁分析, 将ms6初定位于玉米6号染色体C6-19与C6-30两个标记之间, 进一步利用区间内10对新开发的多态性标记, 最终将ms6定位在分子标记M13~M14之间约480 kb的区间范围内。转录组测序结合qRT-PCR试验验证结果, 初步将Zm00001d035201确定为ms6的关键候选基因。Zm00001d035201基因编码一个酸性核糖体蛋白。本研究结果为ms6后续基因功能的研究打下了坚实的基础。同时ms6作为一个新的核不育突变体也为将来玉米新型核不育基因的生产应用提供了重要材料支持。
| [1] | 吴锁伟, 张丹凤, 方才臣, 邓联武, 万向元. 玉米高效农杆菌转化体系的研究进展及其影响因素分析. 玉米科学, 2012, 20(5): 59-64. |
| Wu S W, Zhang D F, Fang C C, Deng L W, Wan X Y. Advances and major influencing factors of high-efficient agrobacterium- mediated genetic transformation in maize. J Maize Sci, 2012, 20(5): 59-64. (in Chinese with English abstract) | |
| [2] | 王保明, 陈永忠, 李红波, 莫华, 黄露波. 植物雄性不育的机制及应用研究进展. 河南农业科学, 2019, 48(5): 1-9. |
| Wang B M, Chen Y Z, Li H B, Mo H, Huang L B. Progress of mechanism of male sterility of plants and its application. J Henan Agric Sci, 2019, 48(5):1-9. (in Chinese with English abstract) | |
| [3] |
Wasiak M, Niedziela A, Woś H, Pojmaj M, Bednarek P T. Genetic mapping of male sterility and pollen fertility QTLs in triticale with sterilizing Triticum timopheevii cytoplasm. J Appl Genet, 2021, 62: 59-71.
doi: 10.1007/s13353-020-00595-z |
| [4] | 孙小媛, 王一帆, 王韫慧, 蔺佳雨, 李金红, 丘远涛, 方小龙, 孔凡江, 李美娜. 大豆细胞核雄性不育基因研究进展. 遗传, 2021, 43: 52-65. |
| Sun X Y, Wang Y F, Wang Y H, Lin J Y, Li J H, Qiu Y T, Fang X L, Kong F J, Li M N. Progress on genic male sterility gene in soybean. Hereditas, 2021, 43: 52-65. (in Chinese with English abstract) | |
| [5] |
Goldberg R B, Beals T P, Sanders P M. Anther development: basic principles and practical applications. Plant Cell, 1993, 5: 1217-1229.
doi: 10.1105/tpc.5.10.1217 pmid: 8281038 |
| [6] |
Chen X Y, Zhang H, Sun H Y, Luo H B, Zhao L, Dong Z B, Yan S S, Zhao C, Liu R Y, Xu C Y, Li S, Chen H B, Jin W W. IRREGULAR POLLEN EXINE1 is a novel factor in anther cuticle and pollen exine formation. Plant Physiol, 2017, 173: 307-325.
doi: 10.1104/pp.16.00629 |
| [7] |
Zhang D B, Wilson Z A. Stamen specification and anther development in rice. Chin Sci Bull, 2009, 54: 2342-2353.
doi: 10.1007/s11434-009-0348-3 |
| [8] | 田有辉, 万向元. 玉米花药发育的细胞生物学与分子遗传学的研究方法. 中国生物工程杂志, 2018, 38(1): 88-89. |
| Tian Y H, Wang X Y. The methods of cell biology and molecular genetics of maize anther development. Chin J Biotechnol, 2018, 38(1): 88-89. (in Chinese with English abstract) | |
| [9] |
Wan X Y, Wu S W, Li Z W, Dong Z Y, An X L, Ma B, Tian Y H, Li J P. Maize genic male-sterility genes and their applications in hybrid breeding: progress and perspectives. Mol Plant, 2019, 12: 321-342.
doi: S1674-2052(19)30020-6 pmid: 30690174 |
| [10] |
Zhang D F, Wu S W, An X L, Xie K, Dong Z Y, Zhou Y, Xu L W, Fang W, Liu S S, Liu S S, Zhu T T, Li J P, Rao L Q, Zhao J R, Wan X Y. Construction of a multicontrol sterility system for a maize male-sterile line and hybrid seed production based on the ZmMs7 gene encoding a PHD-finger transcription factor. Plant Biotechnol J, 2018, 16: 459-471.
doi: 10.1111/pbi.2018.16.issue-2 |
| [11] | Nan G L, Zhai J, Arikit S, Morrow D, Fernandes J, Mai L, Nguyen N, Meyers B C, Walbot V. MS23, a master basic helix-loop-helix factor, regulates the specification and development of the tapetum in maize. Development, 2017, 144: 163-172. |
| [12] |
Moon J, Skibbe D, Timofejeva L, Wang C J, Kelliher T, Kremling K, Walbot V, Cande W Z. Regulation of cell divisions and differentiation by MALE STERILITY32 is required for anther development in maize. Plant J, 2013, 76: 592-602.
doi: 10.1111/tpj.2013.76.issue-4 |
| [13] |
Vernoud V, Laigle G, Rozier F, Meeley R B, Perez P, Rogowsky P M. The HD-ZIP IV transcription factor OCL4 is necessary for trichome patterning and anther development in maize. Plant J, 2009, 59: 883-894.
doi: 10.1111/tpj.2009.59.issue-6 |
| [14] |
Wang D, Adams C M, Fernandes J F, Egger R L, Walbot V.A low molecular weight proteome comparison of fertile and male sterile 8 anthers of Zea mays. Plant Biotechnol J, 2012, 10: 925-935.
doi: 10.1111/j.1467-7652.2012.00721.x pmid: 22748129 |
| [15] |
Wang Y B, Liu D C, Tian Y H, Wu S W, An X L, Dong Z Y, Zhang S M, Bao J X, Li Z W, Li J P, Wan X Y. Map-based cloning, phylogenetic, and microsynteny analyses of ZmMs20 gene regulating male fertility in maize. Int J Mol Sci, 2019, 20: 1411.
doi: 10.3390/ijms20061411 |
| [16] |
Djukanovic V, Smith J, Lowe K, Yang M Z, Gao H R, Jones S, Nicholson M G, West A, Lape J, Bidney D, Carl Falco S, Jantz D, Alexander Lyznik L. Male-sterile maize plants produced by targeted mutagenesis of the cytochrome P450-like gene (MS26) using a re-designed I-CreI homing endonuclease. Plant J, 2013, 76: 888-899.
doi: 10.1111/tpj.12335 |
| [17] |
An X L, Dong Z Y, Tian Y H, Xie K, Wu S W, Zhu T T, Zhang D F, Zhou Y, Niu C F, Ma B, Hou Q C, Bao J X, Zhang S M, Li Z W, Wang Y B, Yan T W, Sun X J, Zhang Y W, Li J P, Wan X Y. ZmMs30 encoding a novel GDSL lipase is essential for male fertility and valuable for hybrid breeding in maize. Mol Plant, 2019, 12: 343-359.
doi: 10.1016/j.molp.2019.01.011 |
| [18] |
Xie K, Wu S W, Li Z W, Zhou Y, Zhang D F, Dong Z Y, An X L, Zhu T T, Zhang S M, Liu S S, Li J P, Wan X Y. Map-based cloning and characterization of Zea mays male sterility 33 (ZmMs33) gene, encoding a glycerol-3-phosphate acyltransferase. Theor Appl Genet, 2018, 131: 1363-1378.
doi: 10.1007/s00122-018-3083-9 pmid: 29546443 |
| [19] |
Fox T, DeBruin J, Haug Collet K, Trimnell M, Clapp J, Leonard A, Li B, Scolaro E, Collinson S, Glassman K, Miller M, Schussler J, Dolan D, Liu L, Gho C, Albertsen M, Loussaert D, Shen B. A single point mutation in Ms44 results in dominant male sterility and improves nitrogen use efficiency in maize. Plant Biotechnol J, 2017, 15: 942-952.
doi: 10.1111/pbi.2017.15.issue-8 |
| [20] |
Cigan A M, Unger E, Xu R J. Phenotypic complementation of ms45 maize requires tapetal expression of MS45. Sex Plant Reprod, 2001, 14: 135-142.
doi: 10.1007/s004970100099 |
| [21] |
Tian Y H, Xiao S L, Liu J, Somaratne Y, Zhang H, Wang M M, Zhang H R, Zhao L, Chen H B. MALE STERILE6021 (MS6021) is required for the development of anther cuticle and pollen exine in maize. Sci Rep, 2017, 7: 16736.
doi: 10.1038/s41598-017-16930-0 |
| [22] |
Somaratne Y, Tian Y H, Zhang H, Wang M M, Huo Y Q, Cao F G, Zhao L, Chen H B. ABNORMAL POLLEN VACUOLATION1 (APV1) is required for male fertility by contributing to anther cuticle and pollen exine formation in maize. Plant J, 2017, 90: 96-110.
doi: 10.1111/tpj.2017.90.issue-1 |
| [23] |
Wang C J, Nan G L, Kelliher T, Timofejeva L, Vernoud V, Golubovskaya I N, Harper L, Egger R, Walbot V, Cande W Z. Maize multiple archesporial cells 1 (mac1), an ortholog of rice TDL1A, modulates cell proliferation and identity in early anther development. Development, 2012, 139: 2594-2603.
doi: 10.1242/dev.077891 |
| [24] | 曹双河, 张相岐, 张爱民. 光(温)敏雄性不育的调控机理和分子遗传学研究进展. 植物学通报, 2005, 22: 19-26. |
| Cao S H, Zhang X Q, Zhang A M. Review of the molecular regulation mechanism and genetics of photoperiod- and/or thermosensitive male sterility. Chin Bull Bot, 2005, 22: 19-26. (in Chinese with English abstract) | |
| [25] | 谢潮添, 杨延红, 葛丽丽, 王瑞, 田惠桥. 白菜核雄性不育花药超微结构的研究. 实验生物学报, 2005, 38: 501-512. |
| Xie C T, Yang Y H, Ge L L, Wang R, Tian H Q. The study on ultrastructure of anther of male sterility in Chinese cabbage. Acta Biol Exp Sin, 2005, 38: 501-512. (in Chinese with English abstract) | |
| [26] |
Vidakovic M B, Vancetovic J, Vidakovic M. A new search for restorer cytoplasm: the restorer cytoplasm for the gene ms10 most probably does not exist in maize. J Hered, 2002, 93: 444-447.
pmid: 12642646 |
| [27] | 王超, 安学丽, 张增为, 杨青, 饶力群, 陈信波, 方才臣, 万向元. 植物隐性核雄性不育基因育种技术体系的研究进展与展望. 植物生物工程杂志, 2013, 33(10): 124-130. |
| Wang C, An X L, Zhang Z W, Yang Q, Rao L Q, Chen X B, Fang C C, Wan X Y. Research progress and prospect of plant recessive nuclear male sterile gene breeding technology system. Chin J Biotechnol, 2013, 33(10): 124-130. (in Chinese with English abstract) | |
| [28] |
An X L, Ma B, Duan M J, Dong Z Y, Liu R G, Yuan D Y, Hou Q C, Wu S W, Zhang D F, Liu D C, Yu D, Zhang Y W, Xie K, Zhu T T, Li Z W, Zhang S M, Tian Y H, Liu C, Li J P, Yuan L P, Wan X Y. Molecular regulation of ZmMs7 required for maize male fertility and development of a dominant male-sterility system in multiple species. Proc Natl Acad Sci USA, 2020, 117: 23499-23509.
doi: 10.1073/pnas.2010255117 |
| [1] | 刘恩波, 陈静, 李红星, 于宁宁, 任佰朝, 赵斌, 刘鹏, 张吉旺. 遮阴改变源-库平衡和调节碳水化合物代谢进而抑制夏玉米幼穗发育[J]. 作物学报, 2026, 52(6): 1891-1901. |
| [2] | 梁进宇, 尹嘉德, 王红丽, 张国平, 侯慧芝, 董博, 马明生. 基于无人机高光谱和机器学习的旱地饲用玉米叶片氮含量估测[J]. 作物学报, 2026, 52(6): 1788-1801. |
| [3] | 孙淑凤, 许振南, 黄嘉鑫, 翁建峰, 李新海. 玉米MAPK家族全基因组鉴定及其对拟轮枝镰孢菌感染的响应[J]. 作物学报, 2026, 52(5): 1291-1308. |
| [4] | 张宁宁, 滕雨菲, 任娜娜, 魏兴卓, 闫书豪, 樊可心, 王永宏, 陈文康, 张兴华, 朱万超, 徐淑兔, 薛吉全. 201份玉米自交系抗旱表型评价及可塑性分析[J]. 作物学报, 2026, 52(5): 1309-1325. |
| [5] | 杨欣雨, 崔文涛, 迪力尼格尔·阿力木, 汪凯翔, 吴鹏昊, 任姣姣. 玉米穗上叶片数全基因组关联分析和全基因组选择[J]. 作物学报, 2026, 52(5): 1573-1590. |
| [6] | 韩亚鑫, 何冠华, 张小琼, 张登峰, 李永祥, 刘旭洋, 王天宇, 黎裕, 邹华文, 李春辉. 基于RNA-Seq和BSA-Seq联合分析挖掘玉米侧根密度基因资源[J]. 作物学报, 2026, 52(5): 1341-1352. |
| [7] | 杨扬, 常诗惠, 田红丽, 易红梅, 王璐, 任洁, 范亚明, 刘亚维, 王凤格, 赵久然. 不同生态区国审玉米品种的遗传多样性分析[J]. 作物学报, 2026, 52(5): 1352-1364. |
| [8] | 张鸿蓉, 王菲儿, 李盼, 仇海龙, 朱静, 赵连豪, 南运有, 何蔚, 樊志龙, 胡发龙, 柴强, 殷文. 减量20%灌水与25%有机肥替代化肥提高青贮玉米产量的光合特性[J]. 作物学报, 2026, 52(5): 1487-1500. |
| [9] | 蔡宏玮, 于爱忠, 姜科强, 王鹏飞, 王玉珑, 霍建喆, 庞小能, 尹波, 尚永盼. 干旱灌区有机肥替代部分化肥促进甜玉米产量提升的关键机制[J]. 作物学报, 2026, 52(4): 1166-1180. |
| [10] | 田红丽, 杨扬, 范亚明, 易红梅, 郭丹丹, 王凤格, 赵久然. 适于玉米品种鉴定的一套三等位变异SNP新型标记组合[J]. 作物学报, 2026, 52(4): 993-1005. |
| [11] | 杨亚莉, 徐明睿, 马越飞, 海艺蕊, 刘凯栋, 刘万茂, 孙颖. 玉米根尖及整根响应缺铁的转录组比较研究[J]. 作物学报, 2026, 52(4): 1006-1021. |
| [12] | 张超, 郭欢, 李忠玲, 岳淑宁, 赵娜. 基于BSA-seq技术定位玉米籽粒花青素关联基因[J]. 作物学报, 2026, 52(3): 780-789. |
| [13] | 郭向阳, 涂亮, 王栋, 刘鹏飞, 王安贵, 易强, 任洪, 李刚, 祝云芳, 吴迅, 蒋喻林, 田丰, 陈泽辉. 热带Suwan种质在我国玉米种质改良中的创新与利用[J]. 作物学报, 2026, 52(3): 655-664. |
| [14] | 孟成, 王哲. 玉米ZmPFK基因家族全基因组鉴定及响应胁迫表达分析[J]. 作物学报, 2026, 52(3): 764-779. |
| [15] | 李新浩, 邢梦柯, 周梓惠, 李思烨, 任昊, 王洪章, 赖华江. 外源褪黑素通过协调光反应与暗反应增强玉米苗期的耐热性[J]. 作物学报, 2026, 52(3): 839-856. |
|
||