欢迎访问作物学报,今天是

作物学报 ›› 2024, Vol. 50 ›› Issue (11): 2731-2741.doi: 10.3724/SP.J.1006.2024.44024

• 作物遗传育种·种质资源·分子遗传学 • 上一篇    下一篇

大豆GmRSM1通过调节PIN基因表达促进顶端弯钩消失

付佳祺1,2(), 李世宽1,2, 谭萌慧1,2, 罗方3, 张传玲3, 刘祾悦3, 卢倩1,*(), 谷勇哲1,2,*()   

  1. 1哈尔滨师范大学生命科学与技术学院, 黑龙江哈尔滨 150025
    2中国农业科学院作物科学研究所, 北京 100081
    3阿荣旗农业事业发展中心, 内蒙古阿荣旗 162750
  • 收稿日期:2024-02-05 接受日期:2024-06-20 出版日期:2024-11-12 网络出版日期:2024-07-10
  • 通讯作者: *卢倩, E-mail: luqian@hrbnu.edu.cn; 谷勇哲, E-mail: guyongzhe@caas.cn
  • 作者简介:E-mail: 1440170828@qq.com
  • 基金资助:
    国家自然科学基金项目(32372190)

Soybean GmRSM1 promotes apical hook disappearance by regulating PIN gene expression

FU Jia-Qi1,2(), LI Shi-Kuan1,2, TAN Meng-Hui1,2, LUO Fang3, ZHANG Chuan-Ling3, LIU Ling-Yue3, LU Qian1,*(), GU Yong-Zhe1,2,*()   

  1. 1College of Life Sciences and Technology, Harbin Normal University, Harbin 150025, Heilongjiang, China
    2Institute of Crop Sciences, Chinese Academy of Agricultural Sciences, Beijing 100081, China
    3Arong Banner Agricultural Development Center, Arong Banner 162750, Inner Mongolia, China
  • Received:2024-02-05 Accepted:2024-06-20 Published:2024-11-12 Published online:2024-07-10
  • Contact: *E-mail: luqian@hrbnu.edu.cn;E-mail: guyongzhe@caas.cn
  • Supported by:
    National Natural Science Foundation of China(32372190)

摘要:

顶端弯钩是双子叶植物黄化幼苗短暂出现的独有结构, 尽管当前拟南芥顶端弯钩的模型网络已经相对透彻, 但在大豆中的研究却非常少。本试验构建pBAR-GmRSM1过表达载体, 通过遗传转化和阳性植株筛选, 得到3个拟南芥过表达纯合株系(OE-GmRSM1#64、#69和#70)和3个大豆纯合株系(OE-GmRSM1#103、#78和#95), 转化体的表达量均显著高于野生型。暗培养拟南芥和大豆, 过表达转化体的顶端弯钩消失或消失速度快于野生型。在扫描电镜下观察拟南芥野生型和转化体植株顶端弯钩部位细胞长度发现, 野生型在弯钩维持阶段弯钩内侧细胞长度小于外侧, 而转化体植株两侧细胞长度相同。分离大豆顶端弯钩内外两侧, 并通过检测PIN基因在大豆野生型与3个过表达转化体顶端弯钩的表达情况, 发现PIN1ePIN3dPIN6a三个基因在子叶出土时的顶端弯钩部位表达量显著高于顶端弯钩展开后的表达量, 而转化体中弯钩处这3个基因在弯钩维持阶段的表达量显著高于野生型, 但在展开后的表达量并无显著性差异。经过烟草瞬时表达, 确定GmRSM1蛋白定位在细胞核和细胞膜。因此, 顶端弯钩出现的原因是弯钩内外两侧细胞差异伸长, 因而导致下胚轴弯曲。GmRSM1可以通过正向调控生长素运输载体PIN1e、PIN3d和PIN6a缩短弯钩维持和展开时间, 验证了该基因对生长素转运的调控作用。本试验通过验证GmRSM1基因在顶端弯钩消失表型中的作用, 进一步完善了顶端弯钩的基因通路, 为后续研究奠定基础。

关键词: 顶端弯钩, 大豆, 拟南芥, PIN家族, 生长素

Abstract:

The apical hook is a transient structure found in etiolated dicot seedlings, and while the current model for the apical hook in Arabidopsis thaliana is relatively well-established, there is limited research on soybean. In this study, the pBAR- GmRSM1 overexpression vector was constructed, and three homozygous lines each of Arabidopsis thaliana (OE-GmRSM1#64, #69, and #70) and soybean (OE-GmRSM1#103, #78, and #95) were generated through genetic transformation and positive plant selection. The expression levels of the transgenic lines were significantly higher than the wild type. Both Arabidopsis thaliana and soybean cultures were grown in darkness, and the apical hooks in the overexpressed transformants disappeared or exhibited faster disappearance than the wild type. Scanning electron microscopy observations of cell length in the apical hook of Arabidopsis thaliana wild-type and transformants revealed that the inner hook cells were shorter than the outer hook cells during the hook maintenance stage, while the cell lengths were same on both sides in the transformant plants. The inner and outer sides of the soybean apical hook were separated, and the expression of the PIN gene in the wild type and three overexpressed transformants of soybean was analyzed. The results demonstrated that the expression levels of the PIN1e, PIN3d, and PIN6a genes were significantly higher in the apical hook after cotyledon unfolding, and during the hook maintenance stage, these three genes exhibited significantly higher expression levels in the transformants than the wild type, but there was no significant difference in expression levels after unfolding. Transient expression in tobacco confirmed than the GmRSM1 protein were localized in the nucleus and cell membrane. Thus, the apical hook formation is attributed to differential cell elongation between the inner and outer sides of the hook, leading to hypocotyl curvature. GmRSM1 regulates the expression of auxin transporters PIN1e, PIN3d, and PIN6a, thereby shortening the duration of hook maintenance and unfolding. These genes are positively regulated by GmRSM1 during the hook stage, and the study confirmed the regulatory effect of this gene on auxin transport. Overall, this study verified the role of GmRSM1 in the disappearance of the apical hook phenotype and further elucidated the gene pathway involved in apical curvature, laying a foundation for future research.

Key words: apical hook, soybean, Arabidopsis, PIN family, auxin

表1

生物信息学预测及分析所用网址"

网站或软件名
Website or software
网址
Uniform resource locator
用途
Purpose
ExPASy ProtParam http://us.expasy.org/tools 氨基酸组成及理化性质预测
Prediction of amino acid composition and physicochemical properties
Cell-PLoc 2.0 http://www.csbio.sjtu.edu.cn/bioinf/Cell-PLoc-2/ 蛋白亚细胞定位预测
Predict protein subcellular localization
SPOMA https://npsa.lyon.inserm.fr/cgi-bin/
secpred_sopma.pl
蛋白二级结构预测
Protein secondary structure prediction
TMHMM-2.0 https://services.healthtech.dtu.dk/
services/TMHMM-2.0/
蛋白跨膜分析
Protein transmembrane analysis
Phytozome 13 https://phytozome-next.jgi.doe.gov/ 获得GmRSM1的启动子序列、CDS序列、编码序列和蛋白序列, 并进行基因结构分析
The promoter sequence, CDS sequence, coding sequence and protein sequence of GmRSM1 were obtained, and the gene structure was analyzed
PlantCARE https://bioinformatics.psb.ugent.be/webtools/plantcare/html/ 启动子区顺式作用元件分析
Analysis of cis-acting elements in the promoter region

图3

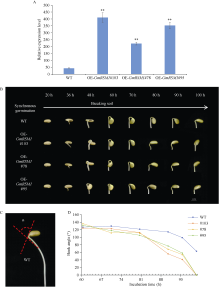
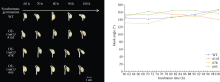
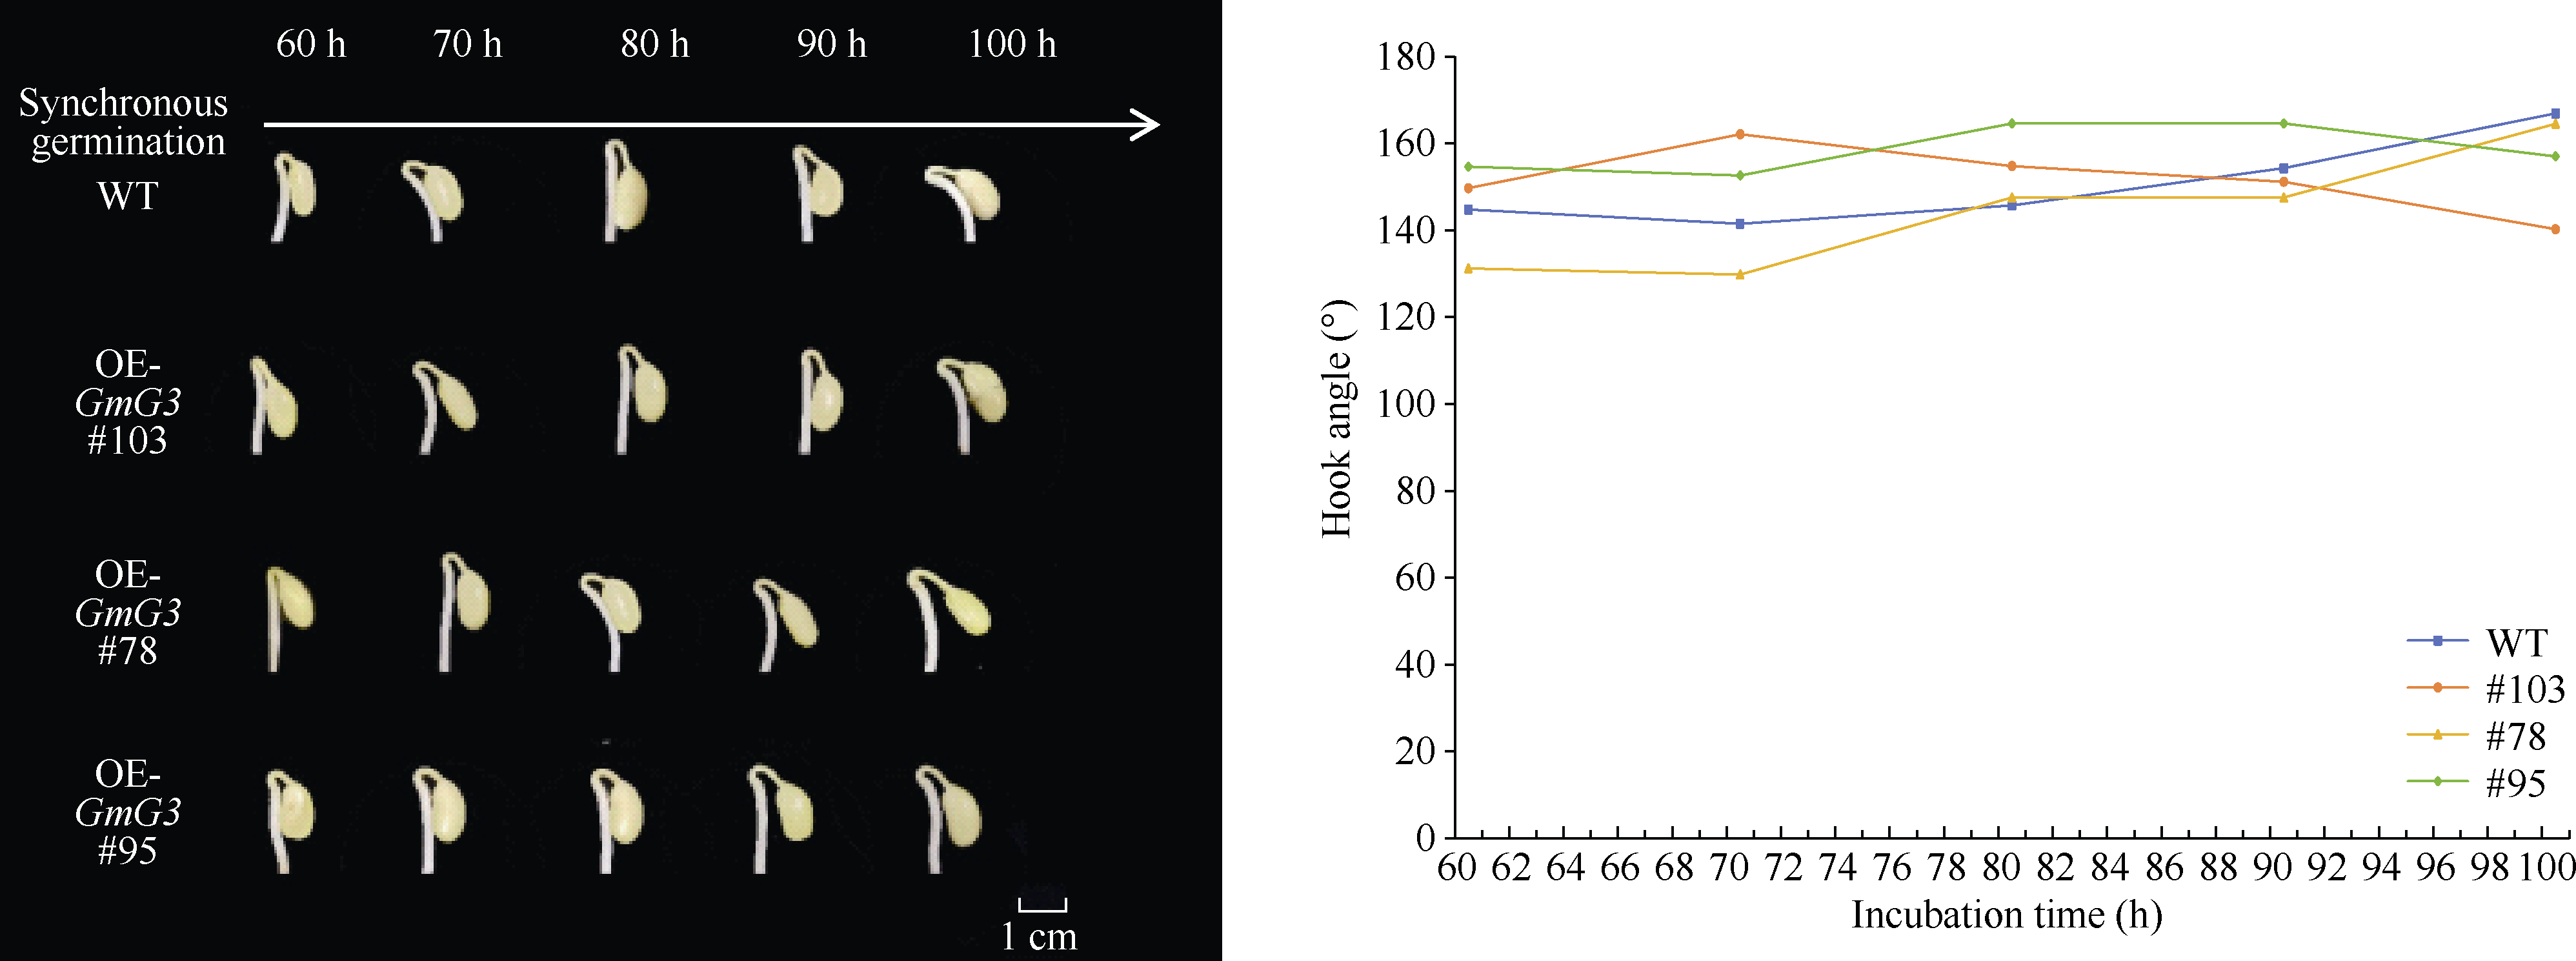
大豆GmRSM1过表达株系与野生型顶端弯钩表型差异 A: qRT-PCR对过表达大豆性株系进行相对表达量测定。图中**代表与野生型WT相比差异极显著(P < 0.01)。B: 大豆表型: 从上到下分别是野生型大豆、转化体OE-GmRSM1#103、#78和#95按培养时间进行表型观测的黄化幼苗的顶端弯钩。C: 大豆的顶端弯钩角度测量示意图。D: 按时间顺序检测并测量的顶端弯钩角度变化折线图。"

附表1

本试验所用引物及用途"

引物名称
Primer name
上游引物
Forward primer (5°-3°)
上游引物
Reverse primer (5°-3°)
引物用途
Primer function
pBAR-GmRSM1 CTCGGTACCCGGGGATCCATGGCCT-CAAGCTCAGCTT GATGAAGGTTCTAAGCCTCCACTGA-TCTAGAGTCCGCAAATCACCAGTCT 基因克隆和构建过表达载体
Gene cloning and overexpression vector construction
qPCR-GmRSM1 GTAAGACTGTGGAGGAAGTGAA AGCATTTCTGTAATTGGGCAAG 荧光定量Real-time PCR
qPCR-GmActin GGTGGTTCTATCTTGGCATC CTTTCGCTTCAATAACCCTA 内参引物Reference primer
qPCR-AtUBQ1 TTCCTTGATGATGCTTGCTC TTGACAGCTCTTGGGTGAAG 内参引物Reference primer
qPCR-PIN1a GCAACCGAGGATCATAGCAT AGAGAACGCCTTTGAGTCCA 荧光定量Real-time PCR
qPCR-PIN1b TGTTGATTGCTTTGCCCATA TGTCTGATGCTCAACAAGCC 荧光定量Real-time PCR
qPCR-PIN1c ATGCAAAGCTTGGTTGAGGT GATCCTGGGGTTCTTCTTCC 荧光定量Real-time PCR
qPCR-PIN1d GCATAAAAAGTGGGACCGAA ATGACAACCTGTGCCATTCA 荧光定量Real-time PCR
qPCR-PIN1e GGGATGCTAATTGCTCTTCCTA GGTAGTTTGATCCACACTGCAA 荧光定量Real-time PCR
qPCR-PIN3a CCCCAACACTTACTCCAGTCTC ATAGCTATACGCAAGAGGGTGC 荧光定量Real-time PCR
qPCR-PIN3b AGAATTCGCAGACACAGCCT GTTGGCTTTGTTCCCACTGT 荧光定量Real-time PCR
qPCR-PIN3c GTGACGGTAGCTTCTCCTCG GAATTCTGGCTCTGGCTCTG 荧光定量Real-time PCR
qPCR-PIN3d ACACTTGCAAAATGGGGAAG GCCCAACTTGTTGAGTCCAT 荧光定量Real-time PCR
qPCR-PIN6a TGCAACTCGTGGTTCTTCAG CGTCGAATTTCGCTATGGAT 荧光定量Real-time PCR
qPCR-PIN6b AGTTCTTGACATGCCCTGCT TTCCCACAAGCTTTTCCAAC 荧光定量Real-time PCR

图1

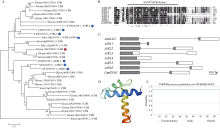
GmRSM1的生物信息学分析 A: 进化树分析。图中红色圆形标注为GmRSM1的蛋白序列, 蓝色圆形标注为拟南芥ATRL1~ATRL6的蛋白序列和金鱼草中AmRAD蛋白序列。B: 蛋白序列保守性比对。图中数字表示每种肽中的氨基酸数, 标有星号的位置表示整个序列的100%一致, 三角形表示RAD-Like特有的残基。C: 基因结构分析; D: 蛋白的三级结构预测; E: 跨膜结构预测。"

表2

GmRSM1基因上游2000 bp的启动子元件分析"

元件
Motif
数量
Number
功能
Function
CAAT-box 47 启动子和增强子区域中常见的顺式作用元件
Common cis-acting element in promoter and enhancer regions
TATA-box 38 转录起始点−30左右的核心启动子元件 Core promoter element around −30 of transcription start
G-box 7 参与光响应的顺式作用调节元件 Cis-acting regulatory element involved in light responsiveness
ABRE 6 参与脱落酸反应的顺式作用元件 Cis-acting element involved in the abscisic acid responsiveness
MYC 5 MYC结合位点元件 MYC binding site element
ABRE3a 3 ABA (脱落酸)应答元件ABA (abscisic acid) transponder
ABRE4 3 ABA (脱落酸)应答元件ABA (abscisic acid) transponder
AT~TATA-box 3 核心启动子元件 Core promoter element
Box 4 3 参与光响应的保守DNA模块的一部分
Part of a conserved DNA module involved in light responsiveness
ACE 2 参与光响应的顺式作用元件 Cis-acting element involved in light responsiveness
ERE 2 乙烯诱导顺式作用元件 Ethylene-induced cis-acting element
TCCC-motif 2 光响应元件的一部分 Part of a light responsive element
TCT-motif 2 光响应元件的一部分 Part of a light responsive element
ATCT-motif 1 参与光响应的保守DNA模块的一部分
Part of a conserved DNA module involved in light responsiveness
Box II 1 光响应元件的一部分 Part of a light responsive element
Box III 1 蛋白结合位点 Protein binding site
CCAAT-box 1 MYB Hv1结合位点 MYB Hv1 binding site
GATA-motif 1 光响应元件的一部分 Part of a light responsive element
GT1-motif 1 光响应元件 Light responsive element
I-box 1 光响应元件的一部分 Part of a light responsive element
MBS 1 MYB结合位点参与干旱诱导 MYB binding site involved in drought-inducibility
MBSI 1 MYB结合位点参与类黄酮生物合成基因调控
MYB binding site involved in flavonoid biosynthetic genes regulation
MYB 2 MYB结合位点元件 MYB binding site element
MYB recognition site 1 MYB识别位点元件 MYB recognizes site-based elements
MYB-like sequence 1 MYB-like序列 MYB-like sequence
STRE 1 应激响应的顺式作用元件 Cis-acting element of stress response
TATC-box 1 参与赤霉素反应的顺式作用元件 Cis-acting element involved in gibberellin-responsiveness
TCA-element 1 参与水杨酸反应性的顺式作用元件 Cis-acting element involved in salicylic acid responsiveness

图2

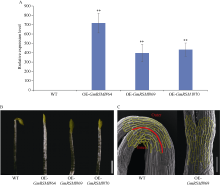
拟南芥过表达GmRSM1株系与野生型顶端弯钩表型差异 A: qRT-PCR对过表达拟南芥阳性株系进行相对表达量测定: 图中**代表与野生型WT相比差异极显著(P < 0.01)。B: 拟南芥表型: 从左到右分别是野生型拟南芥、转化体OE-GmRSM1#64、#69和#70的黄化幼苗顶端弯钩。C: 拟南芥的过表达株系#69及野生型的顶端弯钩电子显微镜扫描图。"

图4

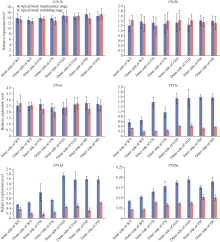
维持阶段和展开阶段PIN基因在顶端弯钩内外的相对表达量"

图5

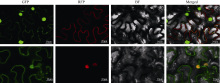
GmRSM1蛋白的亚细胞定位 在绿色荧光、红色荧光、明场和叠加场4个视野下拍摄的照片。标尺为10 μm。"

图6

深播条件下大豆GmRSM1过表达株系与野生型顶端弯钩表型差异"

[1] Veloccia A, Fattorini L, Della Rovere F, Sofo A, D’ Angeli S, Betti C, Falasca G, Altamura M M. Ethylene and auxin interaction in the control of adventitious rooting in Arabidopsis thaliana. J Exp Bot 2016, 67: 6445-6458.
doi: 10.1093/jxb/erw415 pmid: 27831474
[2] Shen X, Li Y, Pan Y, Zhong S. Activation of HLS1 by mechanical stress via ethylene-stabilized EIN3 is crucial for seedling soil emergence. Front Plant Sci, 2016, 7: 1571.
[3] Peng Y, Zhang D, Qiu Y, Xiao Z, Ji Y, Li W, Xia Y, Wang Y, Guo H. Growth asymmetry precedes differential auxin response during apical hook initiation in Arabidopsis. J Integr Plant Biol 2022, 64: 5-22.
[4] Shi H, Liu R, Xue C, Shen X, Wei N, Deng X W, Zhong S. Seedlings transduce the depth and mechanical pressure of covering soil using COP1 and ethylene to regulate EBF1/EBF2 for soil emergence. Curr Biol, 2016, 26: 139-149.
doi: S0960-9822(15)01497-9 pmid: 26748855
[5] Silk W, Erickson R. Kinematics of hypocotyl curvature. Am J Bot, 1978, 65: 310-319.
[6] Weijers D, Nemhauser J, Yang Z. Auxin: small molecule, big impact. J Exp Bot, 2018, 69: 133-136.
doi: 10.1093/jxb/erx463 pmid: 29309681
[7] Schwark A, Schierle J. Interaction of ethylene and auxin in the regulation of hook growth: I. The role for ethylene in different growing regions of the hypocotyl hook of phaseolus vulgaris. J. Plant Physiol, 1992, 140: 562-570.
[8] Žádníková P, Wabnik K, Abuzeineh A, Gallemi M, Van Der Straeten D, Smith R S, Inzé D, Friml J, Prusinkiewicz P, Benková E. A model of differential growth-guided apical hook formation in plants. Plant Cell, 2016, 28: 2464-2477.
[9] Hamaguchi A, Yamashino T, Koizumi N, Kiba T, Kojima M, Sakakibara H, Mizuno T. A small subfamily of Arabidopsis RADIALIS-LIKE SANT/MYB genes: a link to HOOKLESS1- mediated signal transduction during early morphogenesis. Biosci Biotechnol Biochem, 2008, 72: 2687-2696.
[10] Béziat C, Kleine-Vehn J. The road to auxin-dependent growth repression and promotion in apical hooks. Curr Biol, 2018, 28: R519-R525.
[11] Krecek P, Skupa P, Libus J, Naramoto S, Tejos R, Friml J, Zazímalová E. The PIN-FORMED (PIN) protein family of auxin transporters. Genome Biol, 2009, 10: 249.
doi: 10.1186/gb-2009-10-12-249 pmid: 20053306
[12] Zádníková P, Petrásek J, Marhavy P, Raz V, Vandenbussche F, Ding Z, Schwarzerová K, Morita M T, Tasaka M, Hejátko J, Van Der Straeten D, Friml J, Benková E. Role of PIN-mediated auxin efflux in apical hook development of Arabidopsis thaliana. Development 2010, 137: 607-617.
doi: 10.1242/dev.041277 pmid: 20110326
[13] Wang Y, Chai C, Valliyodan B, Maupin C, Annen B, Nguyen H T. Genome-wide analysis and expression profiling of the PIN auxin transporter gene family in soybean (Glycine max). BMC Genomics, 2015, 16: 951.
doi: 10.1186/s12864-015-2149-1 pmid: 26572792
[14] Clough S J, Bent A F. Floral dip: a simplified method for Agrobacterium-mediated transformation of Arabidopsis thaliana. Plant J, 1998, 16: 735-743.
doi: 10.1046/j.1365-313x.1998.00343.x pmid: 10069079
[15] Wang Y, Li Z, Chen X, Gu Y, Zhang L, Qiu L. An efficient soybean transformation protocol for use with elite lines. Plant Cell Tissue Organ Cult, 2022, 151: 457-466.
[16] Cheng G, Dong M, Xu Q, Peng L, Yang Z, Wei T, Xu J. Dissecting the molecular mechanism of the subcellular localization and cell-to-cell movement of the Sugarcane mosaic virus P3N-PIPO. Sci Rep, 2017, 7: 9868.
[17] Wu Q, Li Y, Lyu M, Luo Y, Shi H, Zhong S. Touch-induced seedling morphological changes are determined by ethylene-regulated pectin degradation. Sci Adv, 2020, 6: eabc9294.
[18] Wang Y, Guo H. On hormonal regulation of the dynamic apical hook development. New Phytol, 2019, 222: 1230-1234.
doi: 10.1111/nph.15626 pmid: 30537131
[19] Li H, Johnson P, Stepanova A, Alonso J M, Ecker J R. Convergence of signaling pathways in the control of differential cell growth in Arabidopsis. Dev Cell 2004, 7: 193-204.
[20] Chai C, Wang Y, Valliyodan B, Nguyen H T. Comprehensive analysis of the soybean (Glycine max) GmLAX auxin transporter gene family. Front Plant Sci, 2016, 7: 282.
doi: 10.3389/fpls.2016.00282 pmid: 27014306
[21] Baxter C E, Costa M M, Coen E S. Diversification and co-option of RAD-like genes in the evolution of floral asymmetry. Plant J, 2007, 52: 105-113.
pmid: 17672842
[22] Costa M M, Fox S, Hanna A I, Baxter C, Coen E. Evolution of regulatory interactions controlling floral asymmetry. Development, 2005, 132: 5093-5101.
pmid: 16236768
[23] Corley S B, Carpenter R, Copsey L, Coen E. Floral asymmetry involves an interplay between TCP and MYB transcription factors in Antirrhinum. Proc Natl Acad Sci USA, 2005, 102: 5068-5073.
pmid: 15790677
[1] 金昱何, 王雪菲, 徐张一娃, 缪怡宁, 蒋云杰, 伊莹, 缪德麟, 朱静仪, 钟一帆, 陈铭亨, 方芳, 刘鹏. 外源激素对低温胁迫下大豆叶片叶绿素荧光参数及抗氧化酶系统的影响[J]. 作物学报, 2026, 52(6): 1817-1829.
[2] 唐宽强, 李公允, 宋美毅, 赵雪, 常春玲. 大豆株高性状全基因组关联分析及预测模型构建[J]. 作物学报, 2026, 52(6): 1743-1756.
[3] 张曦, 王广恩, 李邵琦, 刘祎, 李俊兰, 钱玉源. 基于转录组测序解析陆海杂交姊妹系马克隆值差异的形成机制[J]. 作物学报, 2026, 52(5): 1442-1458.
[4] 姚术, 郭凯悦, 翟慧慧, 姚佳慧, 邓文琪, 闫玲, 黄驰, 高阳, 俞嫣然, 赵振邦, 李英慧, 王晓波, 李佳佳. 大豆苗期耐低铁综合评价及优异种质筛选[J]. 作物学报, 2026, 52(5): 1373-1387.
[5] 石少阶, 刘凯, 陈姿夷, 王卉颖, 李三和, 周雷, 游艾青. 水稻矮化多分蘖基因DMT1的克隆与功能分析[J]. 作物学报, 2026, 52(4): 1022-1034.
[6] 张晴, 杨昱, 郭茜, 岳霈尧, 殷丛丛, 牛景萍, 赵晋忠, 杜维俊, 岳爱琴. 大豆GmARA6a的克隆及响应盐胁迫的功能分析[J]. 作物学报, 2026, 52(2): 480-493.
[7] 王克晶, 李向华. 我国珍稀的大豆属多年生烟豆和短绒野大豆物种遗传资源濒危性评估分析[J]. 作物学报, 2025, 51(8): 2009-2019.
[8] 孟然, 李赵嘉, 冯薇, 陈悦, 刘路平, 杨春燕, 鲁雪林, 王秀萍. 大豆不同生育时期耐盐性综合评价及耐盐种质筛选[J]. 作物学报, 2025, 51(8): 1991-2008.
[9] 贺红利, 张雨涵, 杨静, 程云清, 赵杨, 李星诺, 司洪亮, 张兴政, 杨向东. 大豆e1-as基因突变体的创制及生理分析[J]. 作物学报, 2025, 51(8): 2228-2239.
[10] 胡蒙, 沙丹, 张晟瑞, 谷勇哲, 张世碧, 李静, 孙君明, 邱丽娟, 李斌. 大豆分枝数QTL定位及候选基因筛选[J]. 作物学报, 2025, 51(7): 1747-1756.
[11] 雷松翰, 范骏扬, 车艳奕, 代永东, 郑雨萌, 田维江, 桑贤春, 王晓雯. 水稻内卷叶突变体acl3的鉴定及调控基因的功能分析[J]. 作物学报, 2025, 51(6): 1467-1479.
[12] 王琼, 邹丹霞, 陈兴运, 张威, 张红梅, 刘晓庆, 贾倩茹, 魏利斌, 崔晓艳, 陈新, 王学军, 陈华涛. 大豆开花时间和成熟期性状全基因组关联分析与候选基因预测[J]. 作物学报, 2025, 51(6): 1558-1568.
[13] 殷丛丛, 李睿琦, 岳霈尧, 李晨, 牛景萍, 赵晋忠, 杜维俊, 岳爱琴. 基于闭合哑铃介导等温扩增可视化检测大豆花叶病毒SC15方法的建立及应用[J]. 作物学报, 2025, 51(5): 1248-1260.
[14] 张琴, 戴成, 马朝芝. 生长素响应报告基因转化甘蓝型油菜及各组织GUS动态信号分析[J]. 作物学报, 2025, 51(3): 667-675.
[15] 许静, 毕竞男, 殷祥贞, 赵健鑫, 赵旭红, 潘丽娟, 陈娜, 姜骁, 马俊卿, 殷冬梅, 迟晓元. 花生ω-3脂肪酸脱氢酶基因在拟南芥中异源表达及转录组分析[J]. 作物学报, 2025, 51(12): 3251-3265.
Viewed
Full text


Abstract

Cited

  Shared   
  Discussed   
No Suggested Reading articles found!